Membrane association and multimerization of secreton component pulC
Related Experiment Video
Updated: Oct 20, 2026
Transmembrane Domain Oligomerization Propensity determined by ToxR Assay
Published on: May 26, 2011
O M Possot1, M Gérard-Vincent, A P Pugsley
1Unité de Génétique Moléculaire, CNRS URA1773, Institut Pasteur, 75724 Paris Cedex 15, France.

Abstract:
The PulC component of the Klebsiella oxytoca pullulanase secretion machinery (the secreton) was found by subcellular fractionation to be associated with both the cytoplasmic (inner) and outer membranes. Association with the outer membrane was independent of other secreton components, including the outer membrane protein PulD (secretin). The association of PulC with the inner membrane is mediated by the signal anchor sequence located close to its N terminus. These results suggest that PulC forms a bridge between the two membranes that is disrupted when bacteria are broken open for fractionation. Neither the signal anchor sequence nor the cytoplasmic N-terminal region that precedes it was found to be required for PulC function, indicating that PulC does not undergo sequence-specific interactions with other cytoplasmic membrane proteins. Cross-linking of whole cells resulted in the formation of a ca. 110-kDa band that reacted with PulC-specific serum and whose detection depended on the presence of PulD. However, antibodies against PulD failed to react with this band, suggesting that it could be a homo-PulC trimer whose formation requires PulD. The data are discussed in terms of the possible role of PulC in energy transduction for exoprotein secretion.
More Related Videos
 10:01
Directed Assembly of Elastin-like Proteins into defined Supramolecular Structures and Cargo Encapsulation In Vitro
Published on: April 8, 2020
 10:58
SNARE-mediated Fusion of Single Proteoliposomes with Tethered Supported Bilayers in a Microfluidic Flow Cell Monitored by Polarized TIRF Microscopy
Published on: August 24, 2016
Related Concept Videos
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
 01:38
Intralumenal Vesicles and Multivesicular Bodies
 01:29
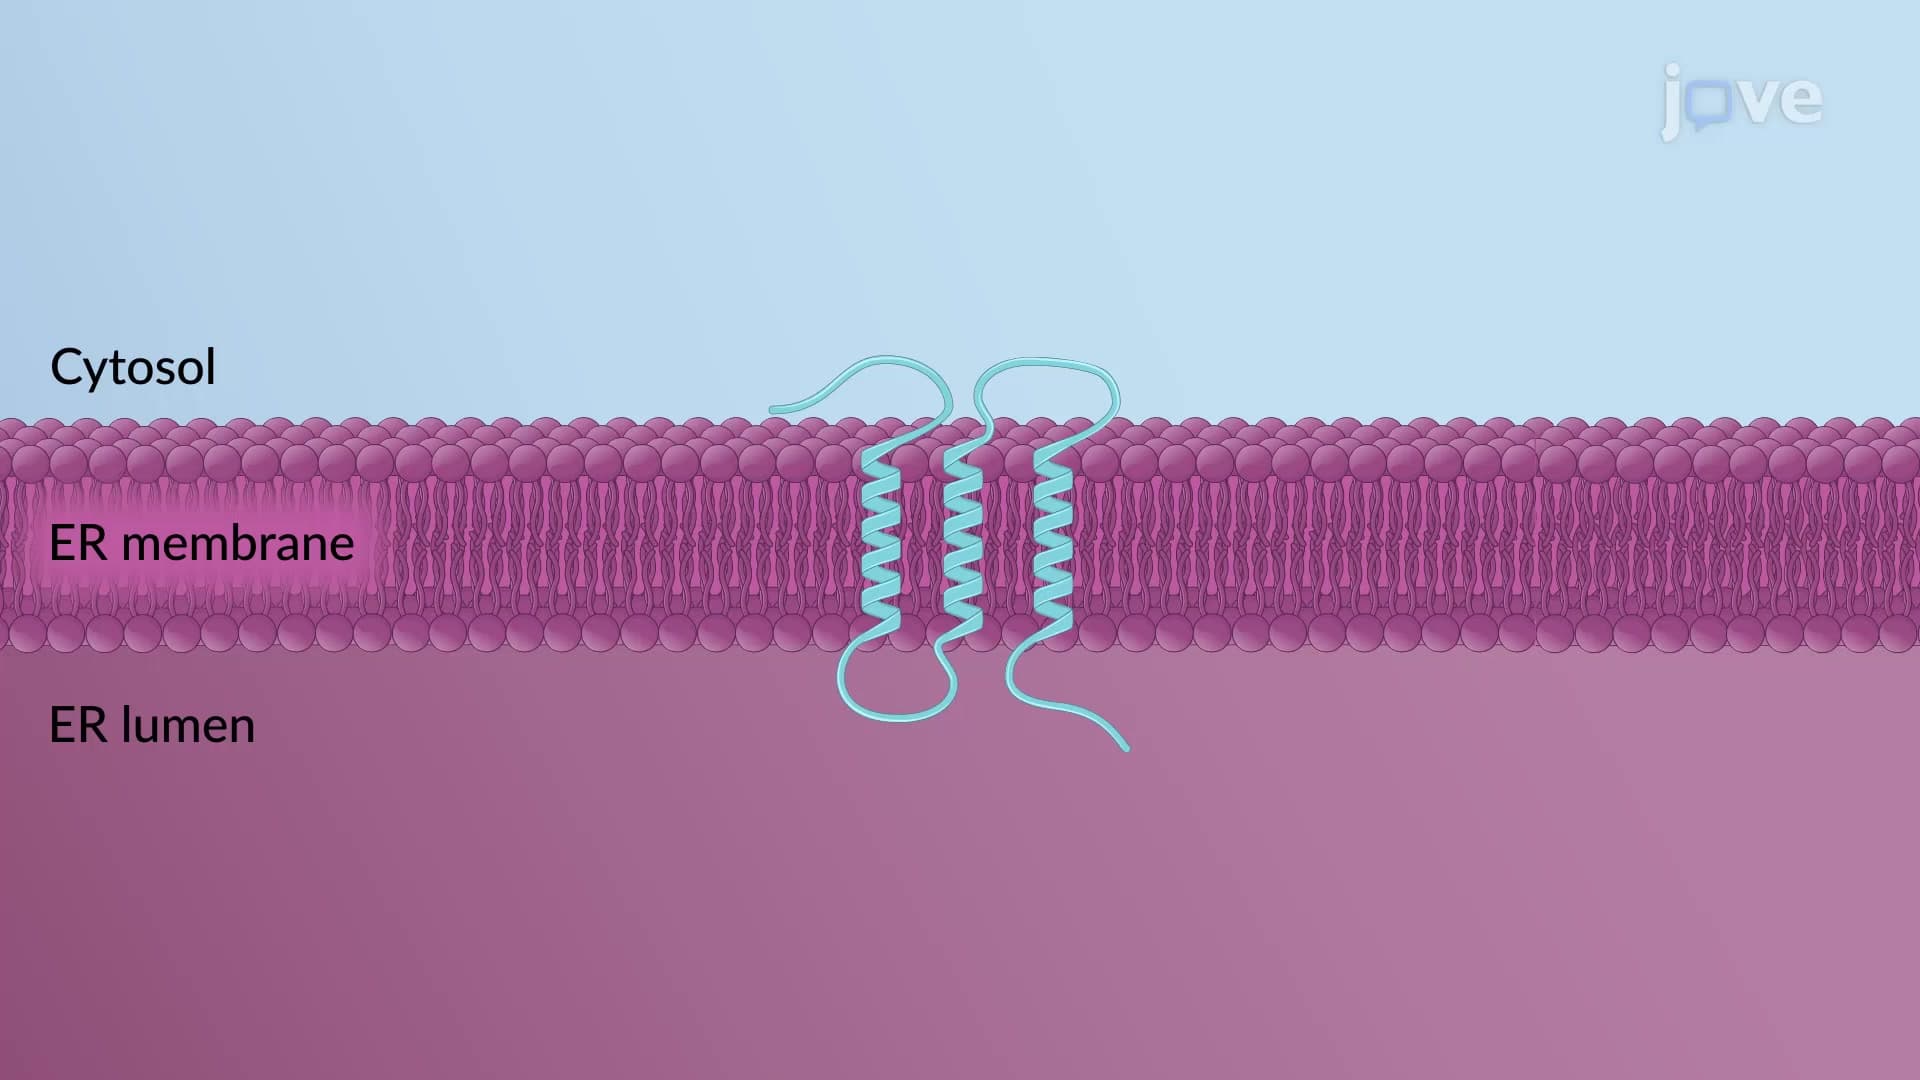
Insertion of Multi-pass Transmembrane Proteins in the RER
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
 01:09
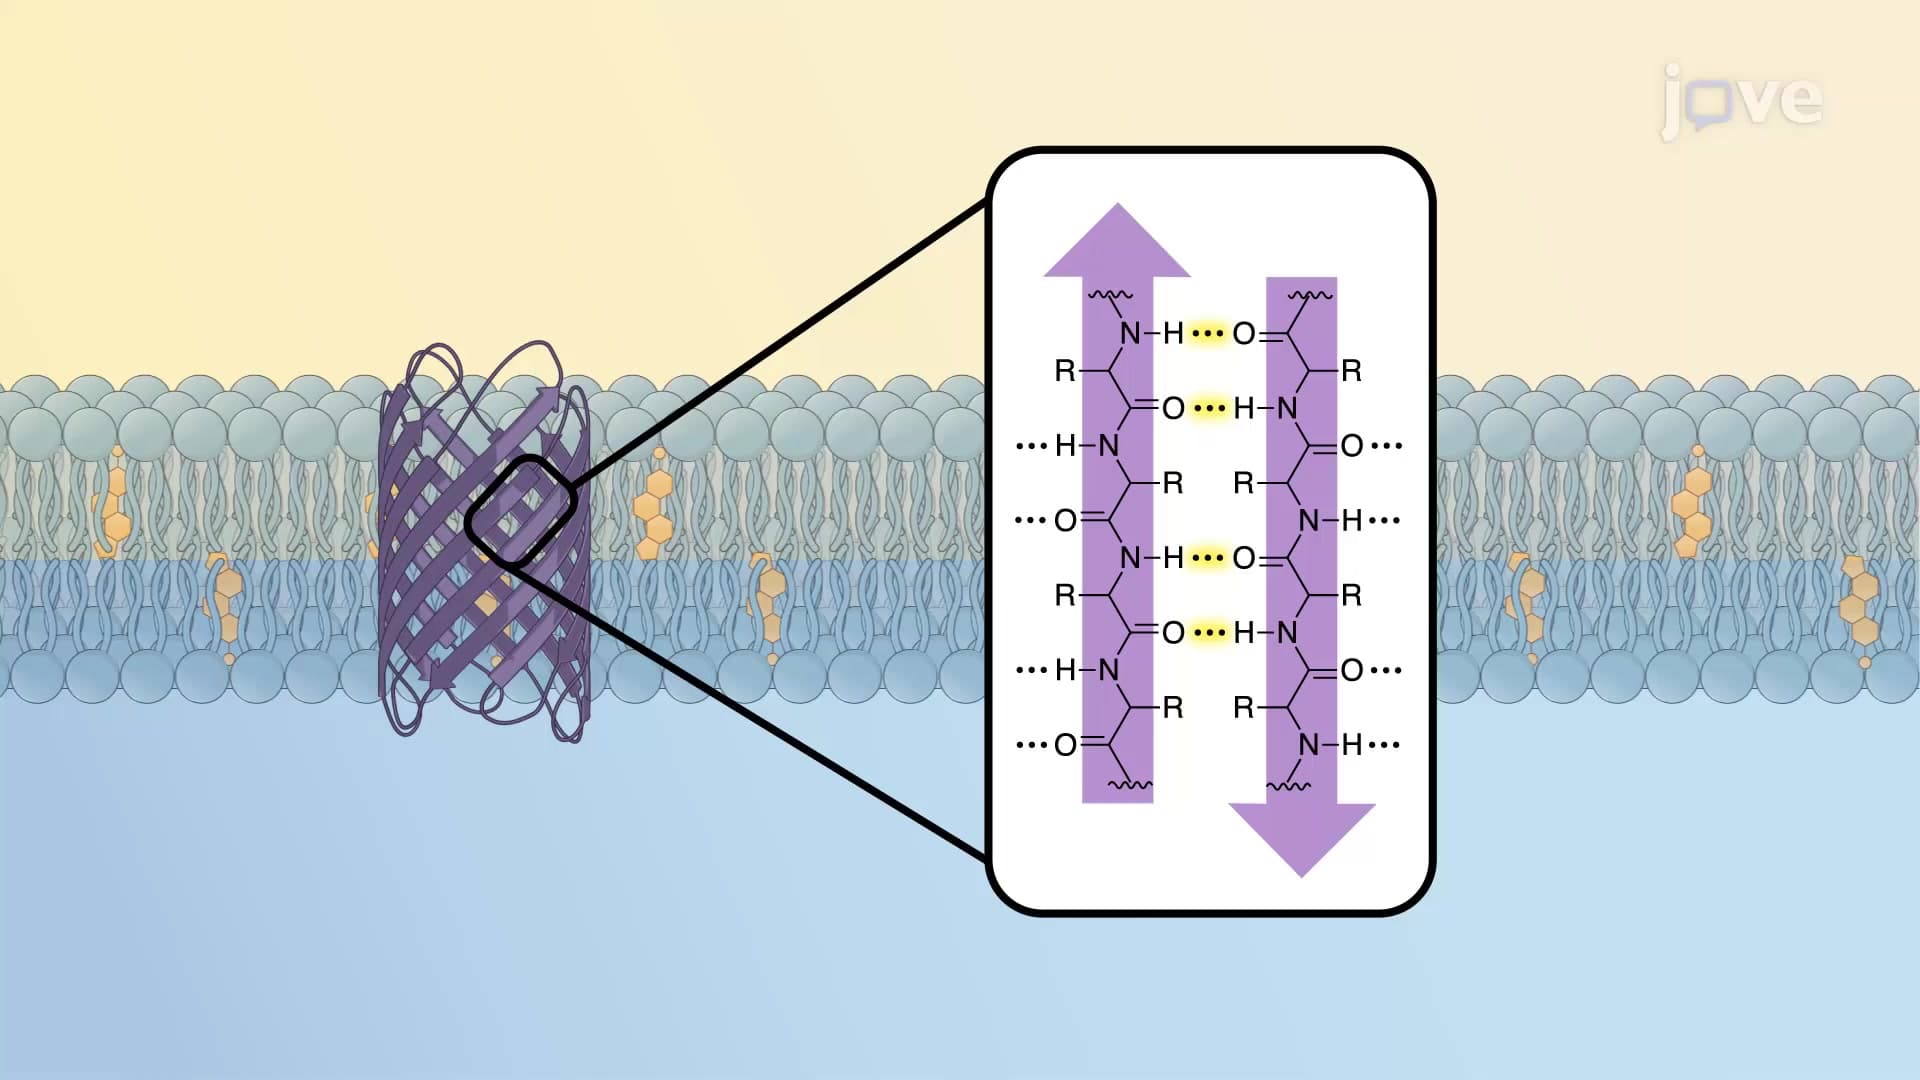
Multi-pass Transmembrane Proteins and β-barrels
α-Helix containing multi-pass transmembrane proteins
Multi-pass transmembrane proteins such as G-protein-linked receptors (GPCRs) and...
 01:28
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...