Related Experiment Video
Updated: Aug 13, 2026

Human T Lymphocyte Isolation, Culture and Analysis of Migration In Vitro
Published on: June 1, 2010
Roles of alpha(4) integrins/VCAM-1 and LFA-1/ICAM-1 in the binding and transendothelial migration of T lymphocytes
C Faveeuw1, M E Di Mauro, A A Price
1Division of Cellular Immunology, National Institute for Medical Research, The Ridgeway, Mill Hill, London NW7 1AA, UK.

Several cell adhesion molecules that mediate the binding of lymphocytes to high endothelial venules (HEV) from flowing blood have been identified but the regulation of lymphocyte migration across the HEV wall into the lymph node (LN) is far from understood. In this study we have used an in vitro model of lymphocyte migration across HEV, and analysed the roles of two integrins in the binding and transendothelial migration of T lymphocytes and T lymphoblasts. The adhesion of T lymphocytes to high endothelial cells (HEC) cultured from rat LN HEV differed from that of T lymphoblasts since the percentage of T lymphoblasts that adhered and transmigrated was higher and was not increased by IFN-gamma pretreatment of HEC. Antibodies to alpha(4) integrins, VCAM-1 or LFA-1 maximally inhibited T lymphocyte adhesion by 40-50%, whereas antibodies to ICAM-1 were less effective (<20% inhibition). The effects of alpha(4) integrin and LFA-1 antibodies were additive, giving >90% inhibition. T lymphocytes which adhered in the presence of LFA-1 antibody showed reduced levels of transmigration and, in the presence of alpha(4) integrin antibody, slightly increased transmigration. Antibodies to alpha(4) integrins, VCAM-1, LFA-1 or ICAM-1 had little effect on T lymphoblast adhesion (maxima of 10-30% inhibition) and T lymphoblasts transmigrated normally in the presence of either alpha(4) integrin or LFA-1 antibodies. However, the effects of alpha(4) integrin and LFA-1 antibodies on T lymphoblast adhesion were synergistic, giving >90% inhibition of adhesion. These results suggest that the majority of T lymphoblasts use either alpha(4) integrins or LFA-1 to bind and transmigrate HEV, and the roles of these integrins on activated T cells are overlapping and redundant. In contrast, either integrin supports half-maximal binding of unactivated T lymphocytes to the surface of HEV and LFA-1 makes a larger contribution than alpha(4) integrins to transendothelial migration.
Several cell adhesion molecules that mediate the binding of lymphocytes to high endothelial venules (HEV) from flowing blood have been identified but the regulation of lymphocyte migration across the HEV wall into the lymph node (LN) is far from understood. In this study we have used an in vitro model of lymphocyte migration across HEV, and analysed the roles of two integrins in the binding and transendothelial migration of T lymphocytes and T lymphoblasts. The adhesion of T lymphocytes to high endothelial cells (HEC) cultured from rat LN HEV differed from that of T lymphoblasts since the percentage of T lymphoblasts that adhered and transmigrated was higher and was not increased by IFN-gamma pretreatment of HEC. Antibodies to alpha(4) integrins, VCAM-1 or LFA-1 maximally inhibited T lymphocyte adhesion by 40-50%, whereas antibodies to ICAM-1 were less effective (<20% inhibition). The effects of alpha(4) integrin and LFA-1 antibodies were additive, giving >90% inhibition. T lymphocytes which adhered in the presence of LFA-1 antibody showed reduced levels of transmigration and, in the presence of alpha(4) integrin antibody, slightly increased transmigration. Antibodies to alpha(4) integrins, VCAM-1, LFA-1 or ICAM-1 had little effect on T lymphoblast adhesion (maxima of 10-30% inhibition) and T lymphoblasts transmigrated normally in the presence of either alpha(4) integrin or LFA-1 antibodies. However, the effects of alpha(4) integrin and LFA-1 antibodies on T lymphoblast adhesion were synergistic, giving >90% inhibition of adhesion. These results suggest that the majority of T lymphoblasts use either alpha(4) integrins or LFA-1 to bind and transmigrate HEV, and the roles of these integrins on activated T cells are overlapping and redundant. In contrast, either integrin supports half-maximal binding of unactivated T lymphocytes to the surface of HEV and LFA-1 makes a larger contribution than alpha(4) integrins to transendothelial migration.
Related Concept Videos
 01:10
Integrins
Some ECM proteins assemble into a basement membrane to which the remaining components adhere. Proteoglycans typically form the bulk of the ECM while fibrous proteins, like collagen,...
 01:15
Activation of Integrins
In "outside-in signaling," external factors in the extracellular space bind to exposed ligand binding sites on integrins. This causes the inactive protein to undergo a conformational change to become active. Integrins are often clustered on the cell membrane. Repetitive and regularly spaced ligand binding events provide an effective stimulus.
 01:17
Intracellular Signaling Affects Focal Adhesions
Some...
 01:20
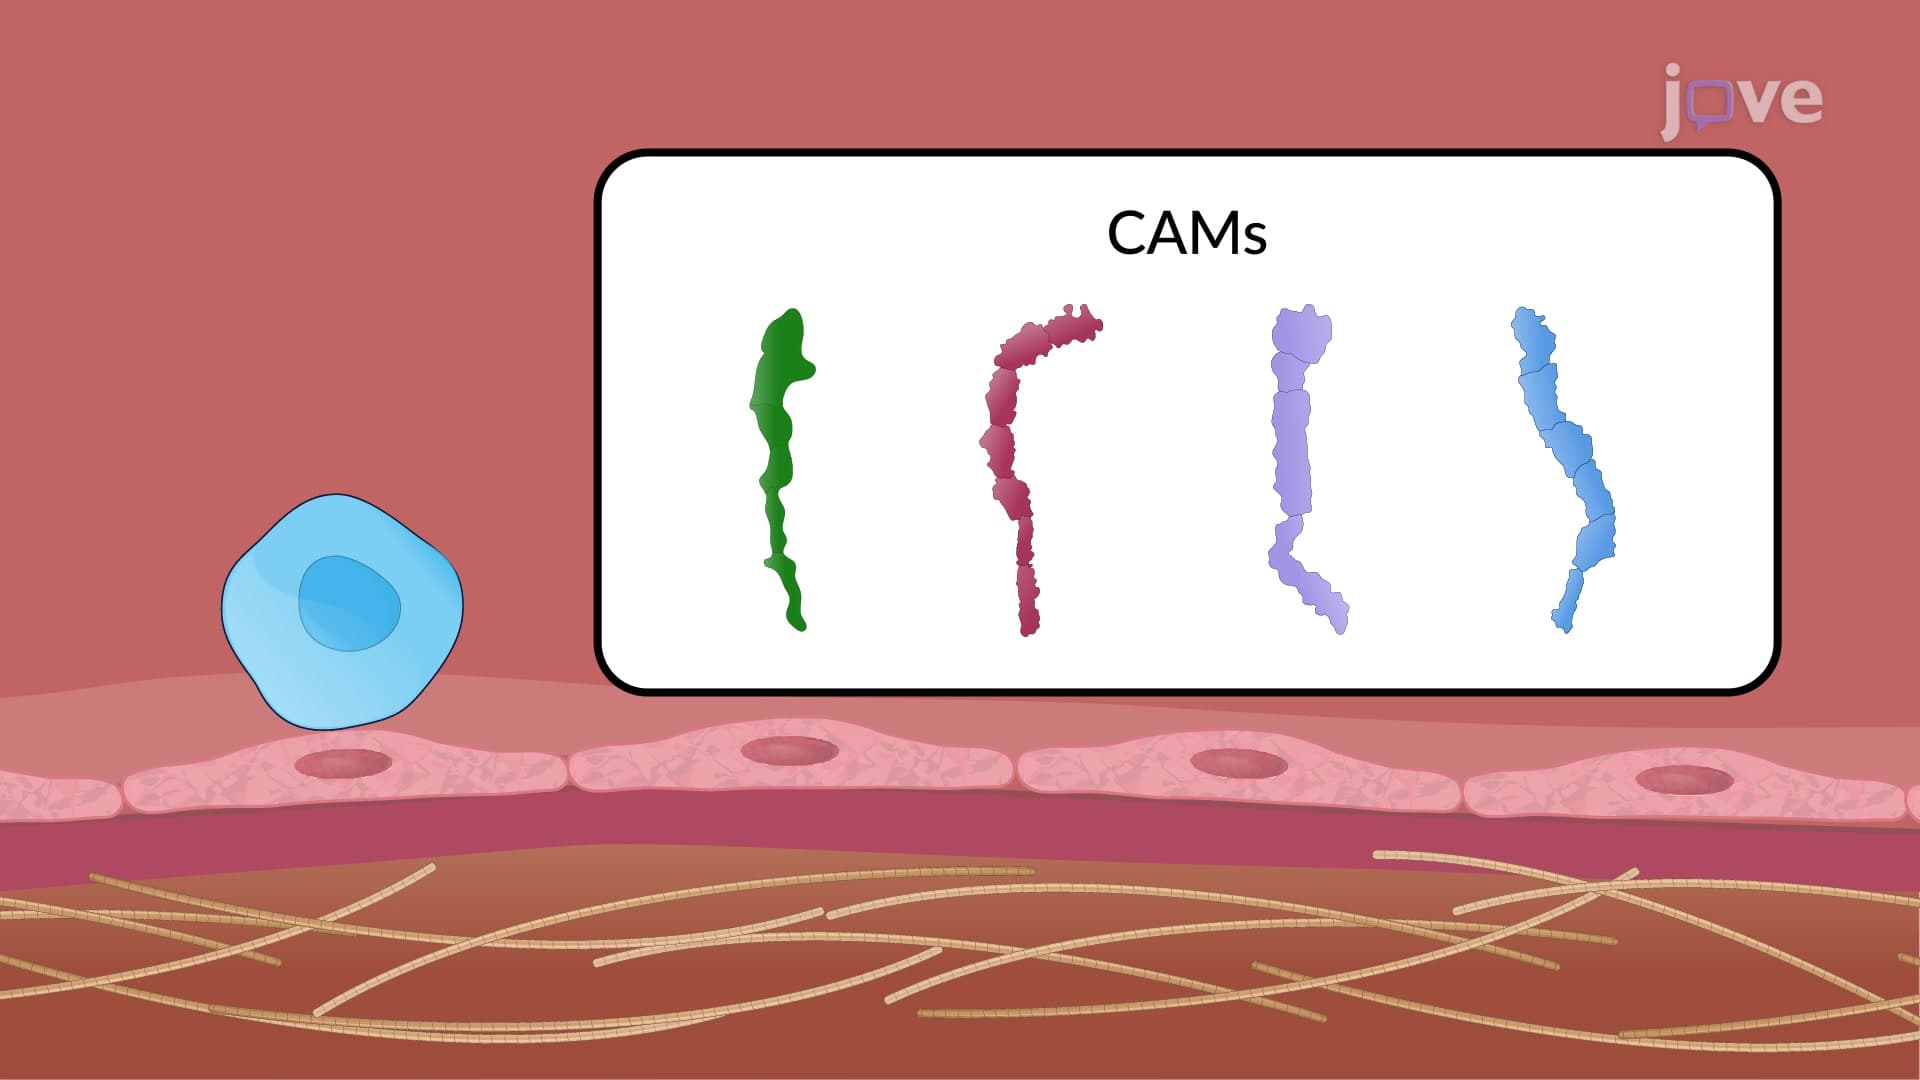
Cell Adhesion Molecules - Types and Functions
CAM Families
The Integrin family of proteins is primarily involved in a...
 01:31
Immunoglobulin-like Cell Adhesion Molecules
Ig-CAMs exhibit either homophilic binding (to other Ig-CAMs) or heterophilic binding (to other ligands such as integrins). While most Ig-CAMs...
01:20Cell Adhesion Molecules - Types and Functions
CAM Families
The Integrin family of proteins is primarily involved in a...