Related Experiment Video
Updated: Oct 11, 2026
The Use of the Patch-Clamp Technique to Study the Thermogenic Capacity of Mitochondria
Published on: May 3, 2021
Chimeric proteins between UCP1 and UCP3: the middle third of UCP1 is necessary and sufficient for activation by fatty
1Division of Endocrinology, RN-320, Department of Medicine, Beth Israel Deaconess Medical Center, Harvard Medical School, 99 Brookline Avenue, Boston, Massachusetts 02215, USA.

Abstract:
Uncoupling protein (UCP) 1 and UCP3 are mitochondrial inner membrane proteins which both mediate proton leak and thus decrease the mitochondrial transmembrane proton gradient. However, UCP1 and UCP3 differ in their biochemical regulation. UCP1 is activated by free fatty acids and inhibited by purine nucleotides. Using heterologous expression studies in yeast, UCP3 was found to lack both fatty acid activation and purine nucleotide inhibition. To assess which domains are responsible for the regulation of UCP1 by free fatty acids and by purine nucleotides and the absence of such regulation in UCP3, chimeric proteins were generated. Given that uncoupling proteins, like all members of the mitochondrial carrier family, possess a tripartite structure and consist of three repeated domains of approximately 100 residues, swaps in the three repeated domains were made between UCP1 and UCP3. Regulation of the resulting six different chimeric proteins by free fatty acids and purine nucleotides was studied after heterologous expression in yeast mitochondria. In this study, it is shown that activation of UCP1 by free fatty acids is mediated by the second repeated domain, since substitution of the second repeat of UCP1 by the equivalent repeat of UCP3 abolishes fatty acid activation. In contrast, replacing the second repeat of UCP3 by the corresponding repeated domain of UCP1 results in fatty acid activation similar to wild type UCP1. The lack of free fatty acid activation of UCP3 is not due to the absence of the histidine pair H145 and H147 found in the second repeated domain of UCP1. Furthermore, the findings with respect to purine nucleotide inhibition are consistent with a significant role of the C-terminal repeated domain of UCP1 in mediating purine nucleotide inhibition.
Related Concept Videos
 01:57
Protein Complexes with Interchangeable Parts
The SCF ubiquitin ligase is a protein complex of five individual proteins. This complex attaches ubiquitin to other target proteins to mark them for degradation. In order to...
 01:31
Regulation of the Unfolded Protein Response
 01:37
The Unfolded Protein Response
 01:29
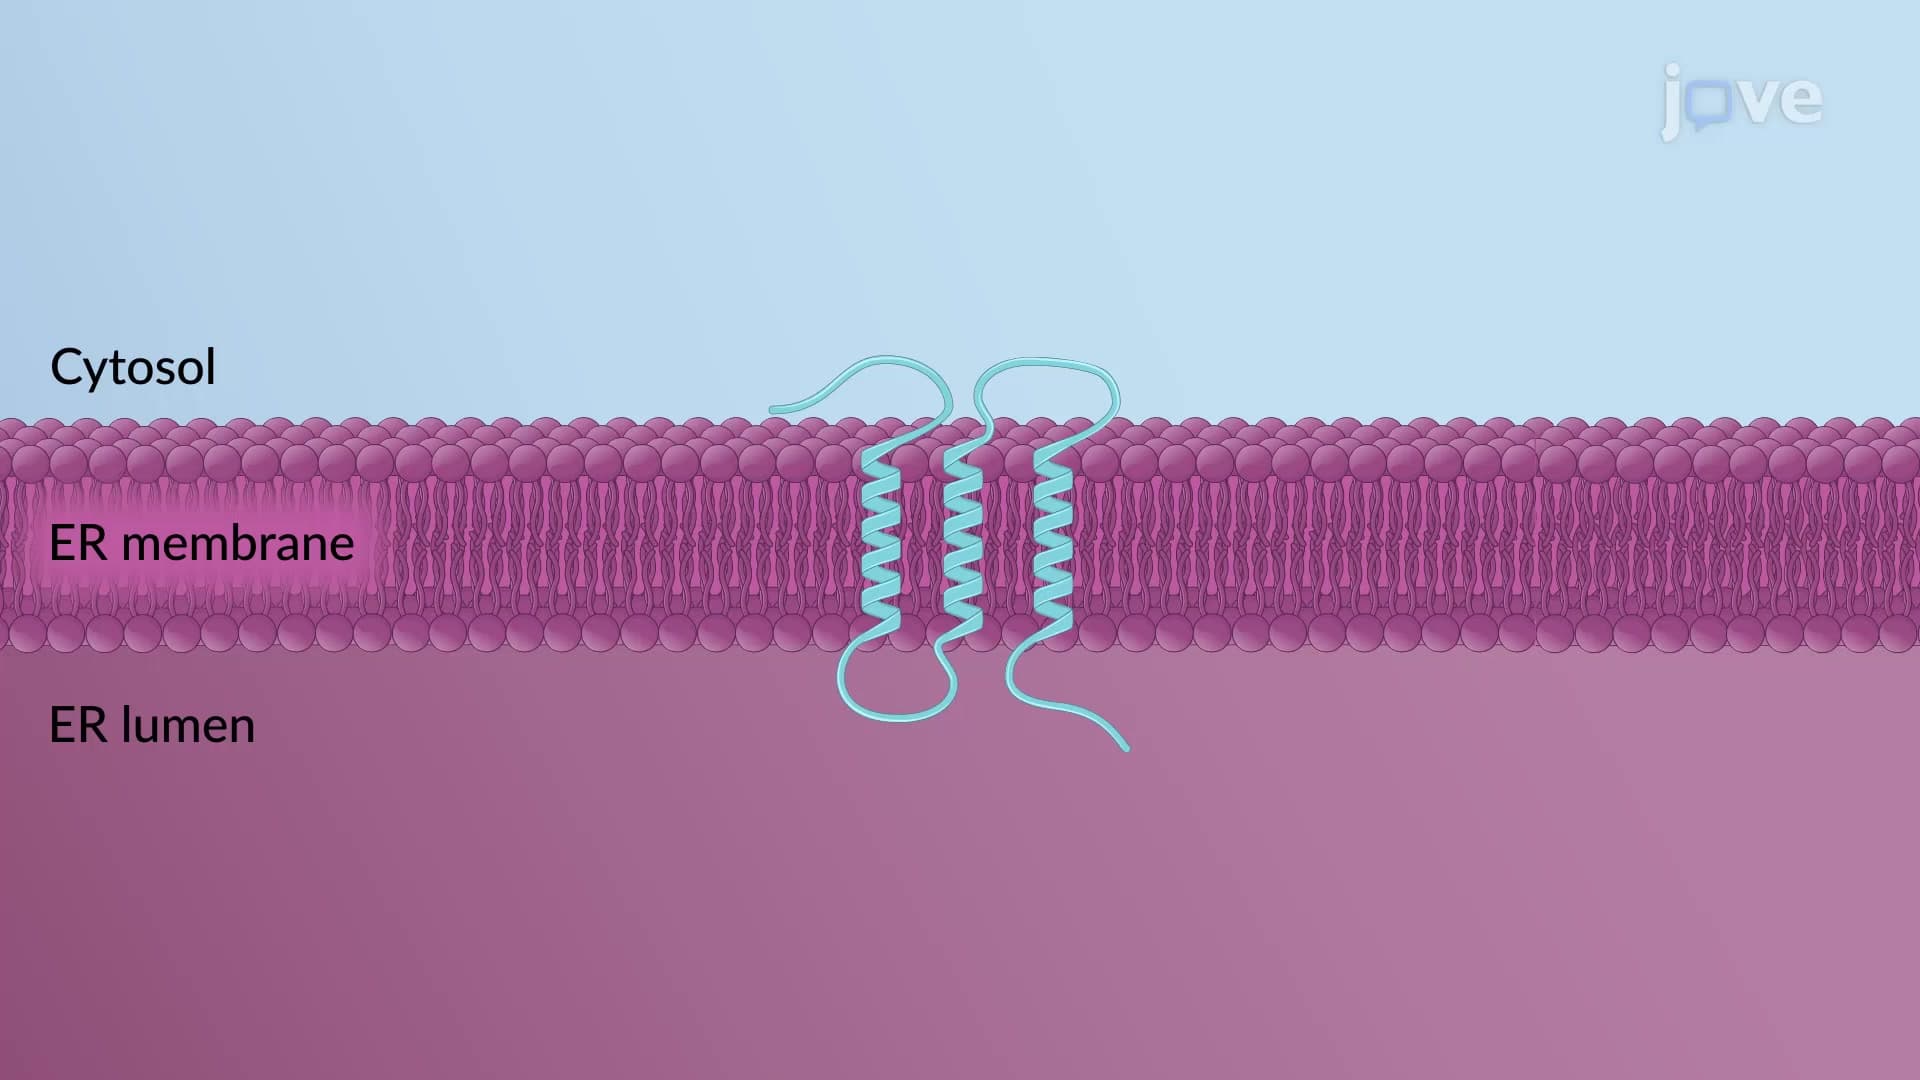
Insertion of Multi-pass Transmembrane Proteins in the RER
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
 01:39
Mitochondrial Precursor Proteins
Most of the mitochondrial precursors...
 01:24
Protein Transport to the Stroma
Protein complexes called the translocon of the outer chloroplast membrane or TOC complex, and the translocon of the inner chloroplast membrane or TIC complex mediate the...