Related Experiment Video
Updated: Oct 11, 2026
Functional Evaluation of Olfactory Pathways in Living Xenopus Tadpoles
Published on: December 11, 2018
Amphibian respiration and olfaction and their relationships: from Robert Townson (1794) to the present
1Zoophysiological Laboratory, August Krogh Institute, Copenhagen, Denmark.

Abstract:
The present review examines the developments in the elucidation of the mechanisms of amphibian respiration and olfaction. Research in these two areas has largely proceeded along independent lines, despite the fact that ventilation of the nasobuccopharyngeal cavity is a basic element in both functions. The English naturalist Robert Townson demonstrated, in the 1790s, that amphibians, contrary to general belief, ventilated the lungs by a pressure-pump mechanism. Frogs and other amphibians respire by alternatively dilating and contracting the buccopharyngeal cavity. During dilatation, with the mouth and glottis closed, air is sucked in through the open nostrils to fill the cavity. During contraction of the throat, with nostrils closed and glottis open, the air in the buccopharyngeal cavity is pressed into the lungs. During expiration, the glottis and nostrils open and air is expelled from the lungs 'by their own contraction from a state of distention'. Herholdt (1801), a Danish army surgeon, independently described the buccal pressure-pump mechanism in frogs, his experiments being confirmed by the commissioners of the Société Philomatique in Paris. Haro (1842) reintroduced a suction mechanism for amphibian respiration, which Panizza (1845) refuted: excision of the tympanic membranes prevented lung inflation, the air in the buccopharyngeal cavity leaving through the tympanum holes. Closure of the holes with the fingers restored lung inflation. The importance of cutaneous respiration in frogs and other amphibians was discovered by Spallanzani (1803), who found that frogs might survive excision of the lungs and that the amounts of exhaled carbon dioxide were small compared with those eliminated through the skin. Edwards (1824) confirmed and extended Spallanzani's findings, and Regnault & Reiset (1849) attempted to establish the relative importance of skin and lungs as respiratory organs in frogs. The problem was solved by Krogh (1904a) who measured respiration through the skin and lungs separately and simultaneously. Krogh (1904a) confirmed that carbon dioxide was chiefly eliminated through the skin, correlated with its high diffusion rate in water and tissue, whereas the pattern of oxygen uptake varied seasonally, the pulmonary uptake being lower than the cutaneous during autumn and winter, but substantially higher during the breeding period. Dolk & Postma (1927) confirmed this respiratory pattern. More recently, Hutchison and coworkers have examined the relative role of pulmonary and cutaneous gas exchange in a large number of amphibians, equipped with head masks for the separate measurement of the lung respiration in normally ventilating animals (Vinegar & Hutchison, 1965; Guimond & Hutchison, 1968; Hutchison, Whitford & Kohl, 1968; Whitford & Hutchison, 1963, 1965, 1966). As early as 1758, Rösel von Rosenhof suggested that the lungs of frogs in water functioned as hydrostatic organs that permitted the animal to float at the surface or rest on the bottom of the pond. The suggestion was inspired by observations made in the second half of the seventeenth century by members of the Royal Academy of Sciences in Paris. The French anatomists demonstrated that a tortoise, presumably the European freshwater turtle Emys orbicularis, could regulate its buoyancy by changing the volume of the lungs, to descend passively or ascend in the water. The hydrostatic function of the lungs has been repeatedly rediscovered, by Emery (1869) in the frog, by Marcacci (1895) in frogs, toads and salamanders, by Whipple (1906b) in a newt, by Willem (1920, 1931) in frogs and Xenopus laevis, by Speer 1942) in several anurans and urodeles, and finally by de Jongh (1972) in Xenopus laevis. In the second half of the nineteenth century a number of important papers appeared which confirmed and extended Townson's (1794) and Panizza's (1845) analysis of the normal respiratory movements in frogs. (ABSTRACT TRUNCATED)
Related Concept Videos
 01:25
Olfaction
The olfactory receptors are embedded in the cilia of the...
 01:03
Olfactory Receptors: Location and Structure
 01:20
Physiology of Smell and Olfactory Pathway
The olfactory...
 01:23
Physiological Control of Respiration
Breathing, a seemingly passive process, is regulated by the respiratory center in the brainstem. This center coordinates the involuntary control of respirations, which means it occurs without conscious effort, ensuring a smooth and uninterrupted pattern.
Regulation of Ventilation
The body maintains ventilation by monitoring levels of carbon dioxide (CO2), oxygen (O2), and hydrogen ion concentration (pH) in the arterial blood. Among these factors, the level of CO2 plays a crucial...
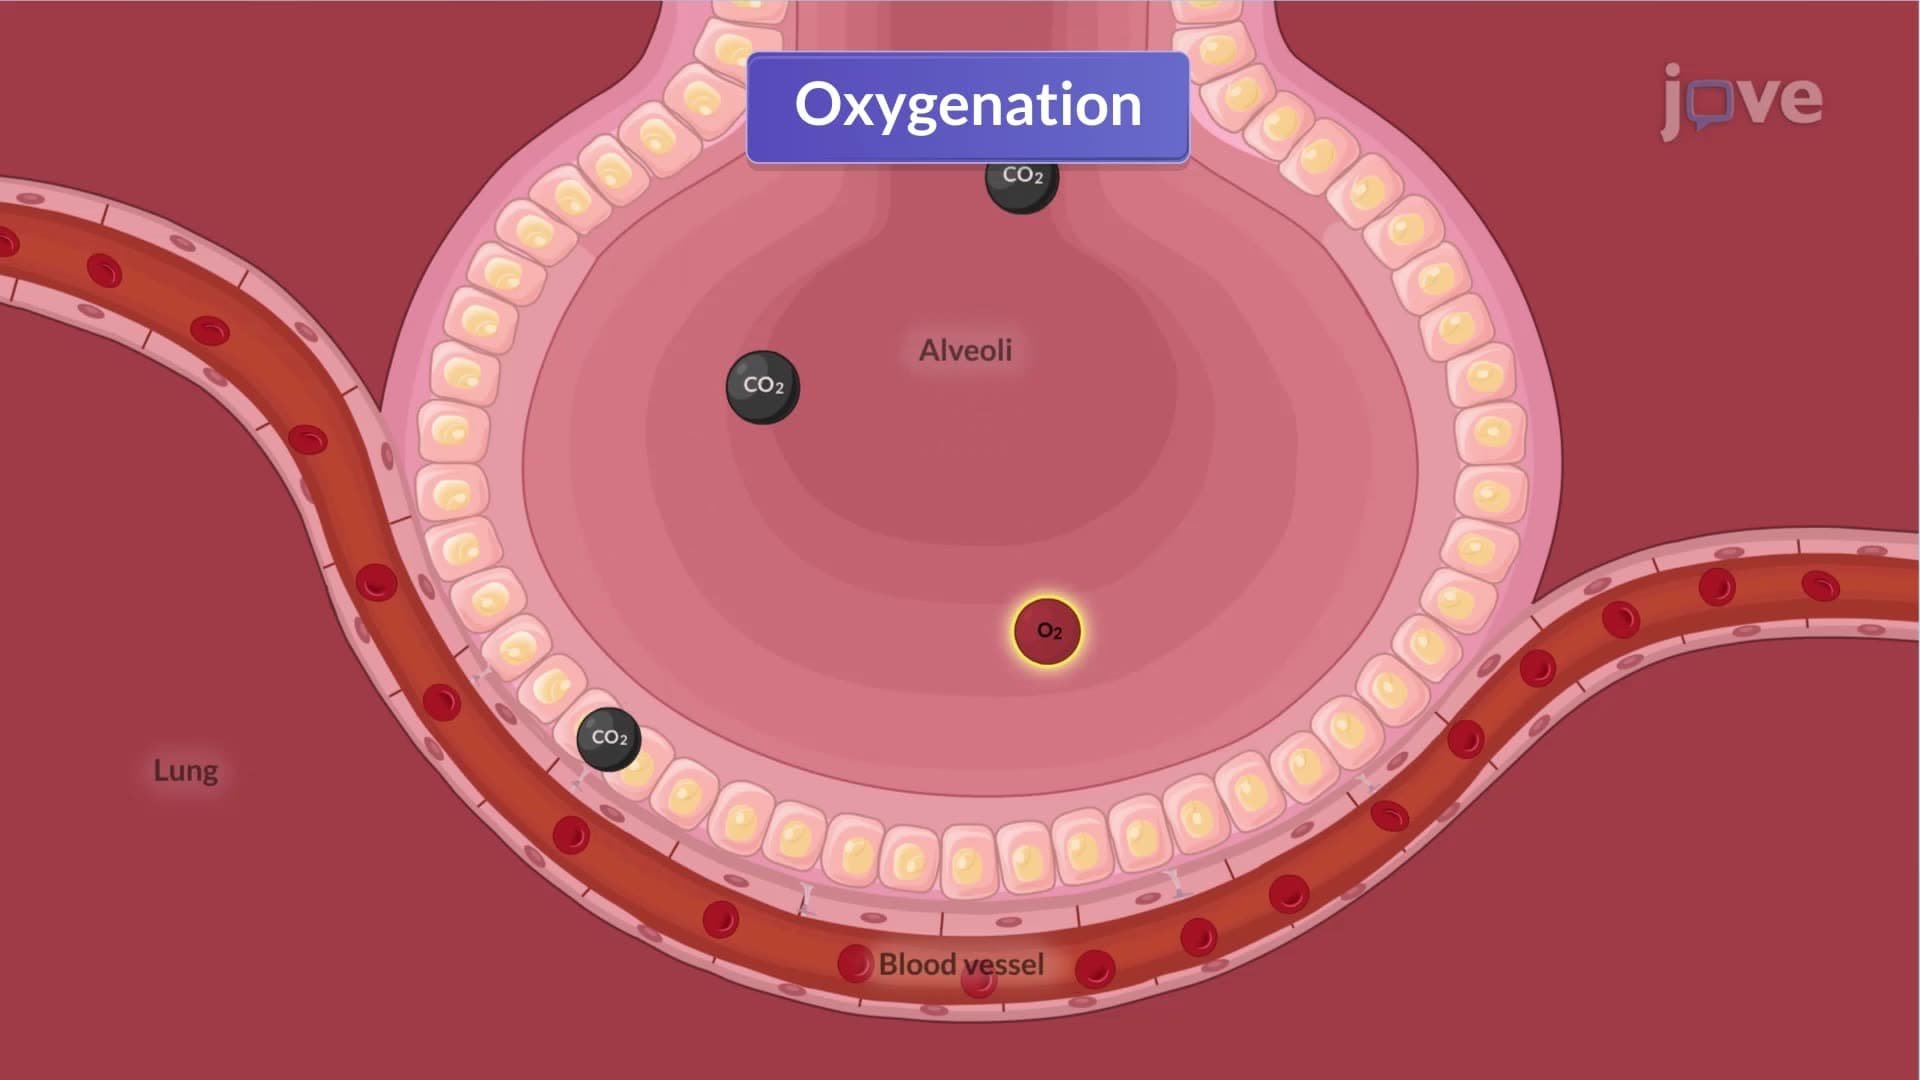 01:27
Physiology of Respiration I: Functions of the Respiratory System
Fundamental Processes in Respiration:
 01:23
Overview of Respiratory System
What is the Respiratory System?
The respiratory system consists of a series of organs responsible for taking in oxygen and expelling carbon dioxide. The primary function of the respiratory system is to...