Related Experiment Video
Updated: Oct 10, 2026
Pharmacophore Modeling for Targets with Extensive Ligand Libraries: A Case Study on SARS-CoV-2 Mpro
Published on: September 26, 2025
Role of aromatic residues at the lipid-water interface in micelle-bound bacteriophage M13 major coat protein
C T Yuen1, A R Davidson, C M Deber
1Division of Structural Biology and Biochemistry, Research Institute, Hospital for Sick Children, 555 University Avenue, Toronto, Ontario, Canada M5G 1X8.

Abstract:
Analyses of transmembrane domains of proteins have revealed that aromatic residues tend to cluster at or near the lipid-water interface of the membrane. To assess protein-membrane interactions of such residues, a viable mutant library was generated of the major coat protein of bacteriophage M13 (a model single membrane-spanning protein) in which one or the other of its interfacial tyrosine residues (Tyr-21 and Tyr-24) is mutated. Using the interfacial tryptophan (Trp-26) as an intrinsic probe, blue shifts in fluorescence emission spectra and quenching constants indicated that mutants with a polar amino acid substitution (such as Y24D or Y24N) are less buried in a deoxycholate micelle environment than in the wild type protein. These polar mutants also exhibited alpha-helix to beta-structure transition temperatures in incremental-heating circular dichroism studies relatively lower than those of wild type and nonpolar mutants (such as Y21V, Y21I, and Y24A), indicating that specific side chains in the lipid-water interface influence local protein-micelle interactions. Mutant Y21F exhibited the highest transition temperature, suggesting that phenylalanine is ostensibly the most effective interfacial anchoring residue. Using phage viability as the assay in a combination of site-directed and saturation mutagenesis experiments, it was further observed that both Tyr residues could not simultaneously be "knocked out". The overall results support the notion that an interfacial Tyr is a primary recognition element for precise strand positioning in vivo, a function that apparently cannot be performed optimally by residues with simple aliphatic character.
Insights
Aromatic residues like tyrosine cluster at membrane interfaces. Mutating these residues in M13 phage coat protein affects protein-micelle interactions and stability, with tyrosine proving crucial for proper in vivo positioning.
Area of Science:
- Biochemistry
- Structural Biology
- Membrane Biophysics
Background:
- Aromatic residues are observed to aggregate near the lipid-water interface in transmembrane protein domains.
- Understanding the role of these interfacial residues in protein-membrane interactions is crucial for deciphering membrane protein function.
Purpose of the Study:
- To investigate the role of interfacial tyrosine residues (Tyr-21 and Tyr-24) in the major coat protein of bacteriophage M13 (a model single membrane-spanning protein).
- To assess how mutations in these tyrosine residues impact protein-micelle interactions and structural stability.
Main Methods:
- Generation of a viable mutant library of the M13 major coat protein with specific mutations at Tyr-21 and Tyr-24.
- Utilizing intrinsic fluorescence of tryptophan (Trp-26) to probe changes in the micelle environment of mutants.
- Employing incremental-heating circular dichroism studies to determine alpha-helix to beta-structure transition temperatures.
- Performing site-directed and saturation mutagenesis experiments with phage viability as the assay.
Main Results:
- Polar mutations (e.g., Y24D, Y24N) resulted in reduced burial within deoxycholate micelles compared to wild-type protein.
- Polar mutants exhibited lower transition temperatures, indicating decreased structural stability.
- Nonpolar mutations and phenylalanine substitution (Y21F) showed increased stability, with Y21F being the most effective interfacial anchor.
- Simultaneous knockout of both tyrosine residues was not viable, highlighting their essentiality.
Conclusions:
- Specific side chains at the lipid-water interface significantly influence local protein-micelle interactions and protein stability.
- Interfacial tyrosine residues are critical for precise in vivo strand positioning, a function not optimally replaced by aliphatic residues.
Related Concept Videos
 01:26
DNA Bacteriophages
 01:23
Bacteriophages of the Human Virome
 01:30
Lytic Cycle of Bacteriophages
 01:19
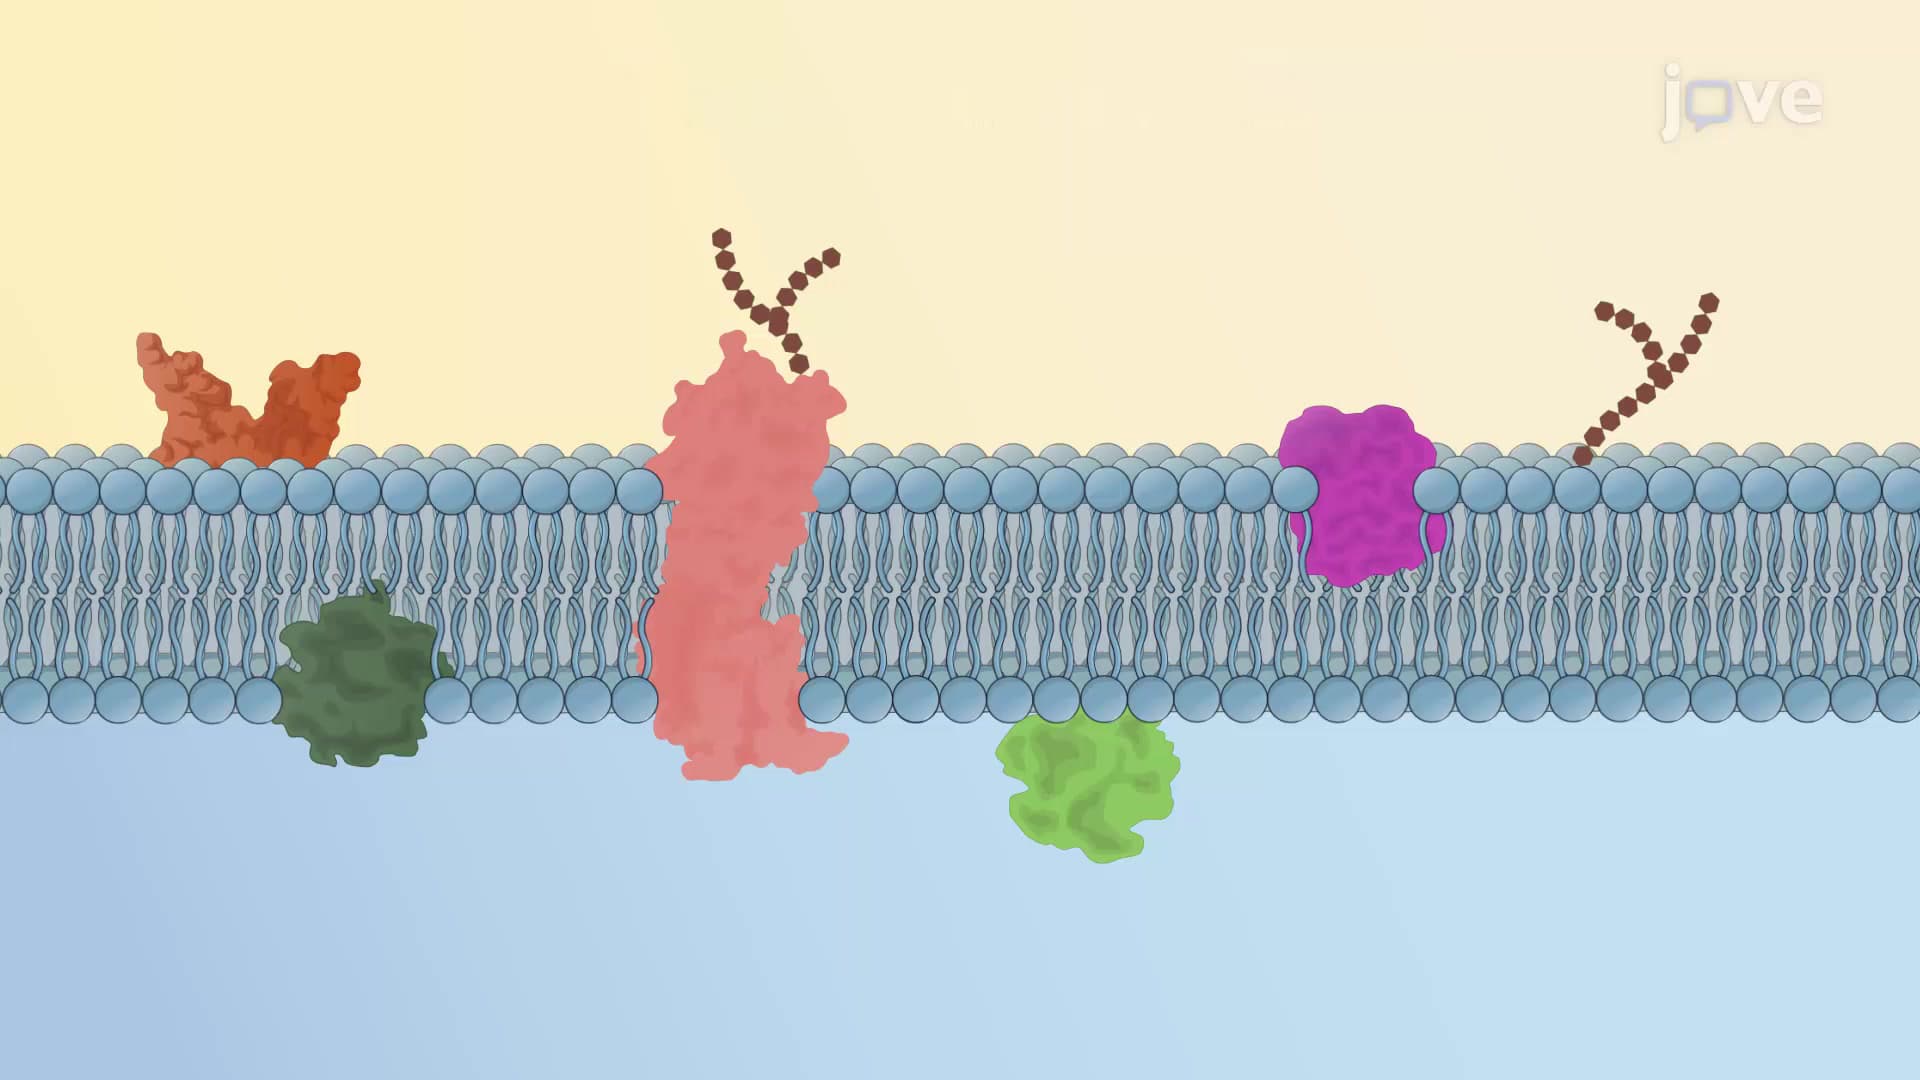
Fluid Mosaic Model
 01:32
Pinching-off of Coated Vesicles
 01:33
Coat Assembly and GTPases
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...