Related Experiment Video
Updated: Jul 14, 2026

Bacterial Inner-membrane Display for Screening a Library of Antibody Fragments
Published on: October 15, 2016
Specificity of signal peptide recognition in tat-dependent bacterial protein translocation
N Blaudeck1, G A Sprenger, R Freudl
1Institut für Biotechnologie 1, Forschungszentrum Jülich GmbH, D-52425 Jülich, Germany.

Abstract:
The bacterial twin arginine translocation (Tat) pathway translocates across the cytoplasmic membrane folded proteins which, in most cases, contain a tightly bound cofactor. Specific amino-terminal signal peptides that exhibit a conserved amino acid consensus motif, S/T-R-R-X-F-L-K, direct these proteins to the Tat translocon. The glucose-fructose oxidoreductase (GFOR) of Zymomonas mobilis is a periplasmic enzyme with tightly bound NADP as a cofactor. It is synthesized as a cytoplasmic precursor with an amino-terminal signal peptide that shows all of the characteristics of a typical twin arginine signal peptide. However, GFOR is not exported to the periplasm when expressed in the heterologous host Escherichia coli, and enzymatically active pre-GFOR is found in the cytoplasm. A precise replacement of the pre-GFOR signal peptide by an authentic E. coli Tat signal peptide, which is derived from pre-trimethylamine N-oxide (TMAO) reductase (TorA), allowed export of GFOR, together with its bound cofactor, to the E. coli periplasm. This export was inhibited by carbonyl cyanide m-chlorophenylhydrazone, but not by sodium azide, and was blocked in E. coli tatC and tatAE mutant strains, showing that membrane translocation of the TorA-GFOR fusion protein occurred via the Tat pathway and not via the Sec pathway. Furthermore, tight cofactor binding (and therefore correct folding) was found to be a prerequisite for proper translocation of the fusion protein. These results strongly suggest that Tat signal peptides are not universally recognized by different Tat translocases, implying that the signal peptides of Tat-dependent precursor proteins are optimally adapted only to their cognate export apparatus. Such a situation is in marked contrast to the situation that is known to exist for Sec-dependent protein translocation.
Related Concept Videos
 01:20
Cotranslational Protein Translocation
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
 01:26
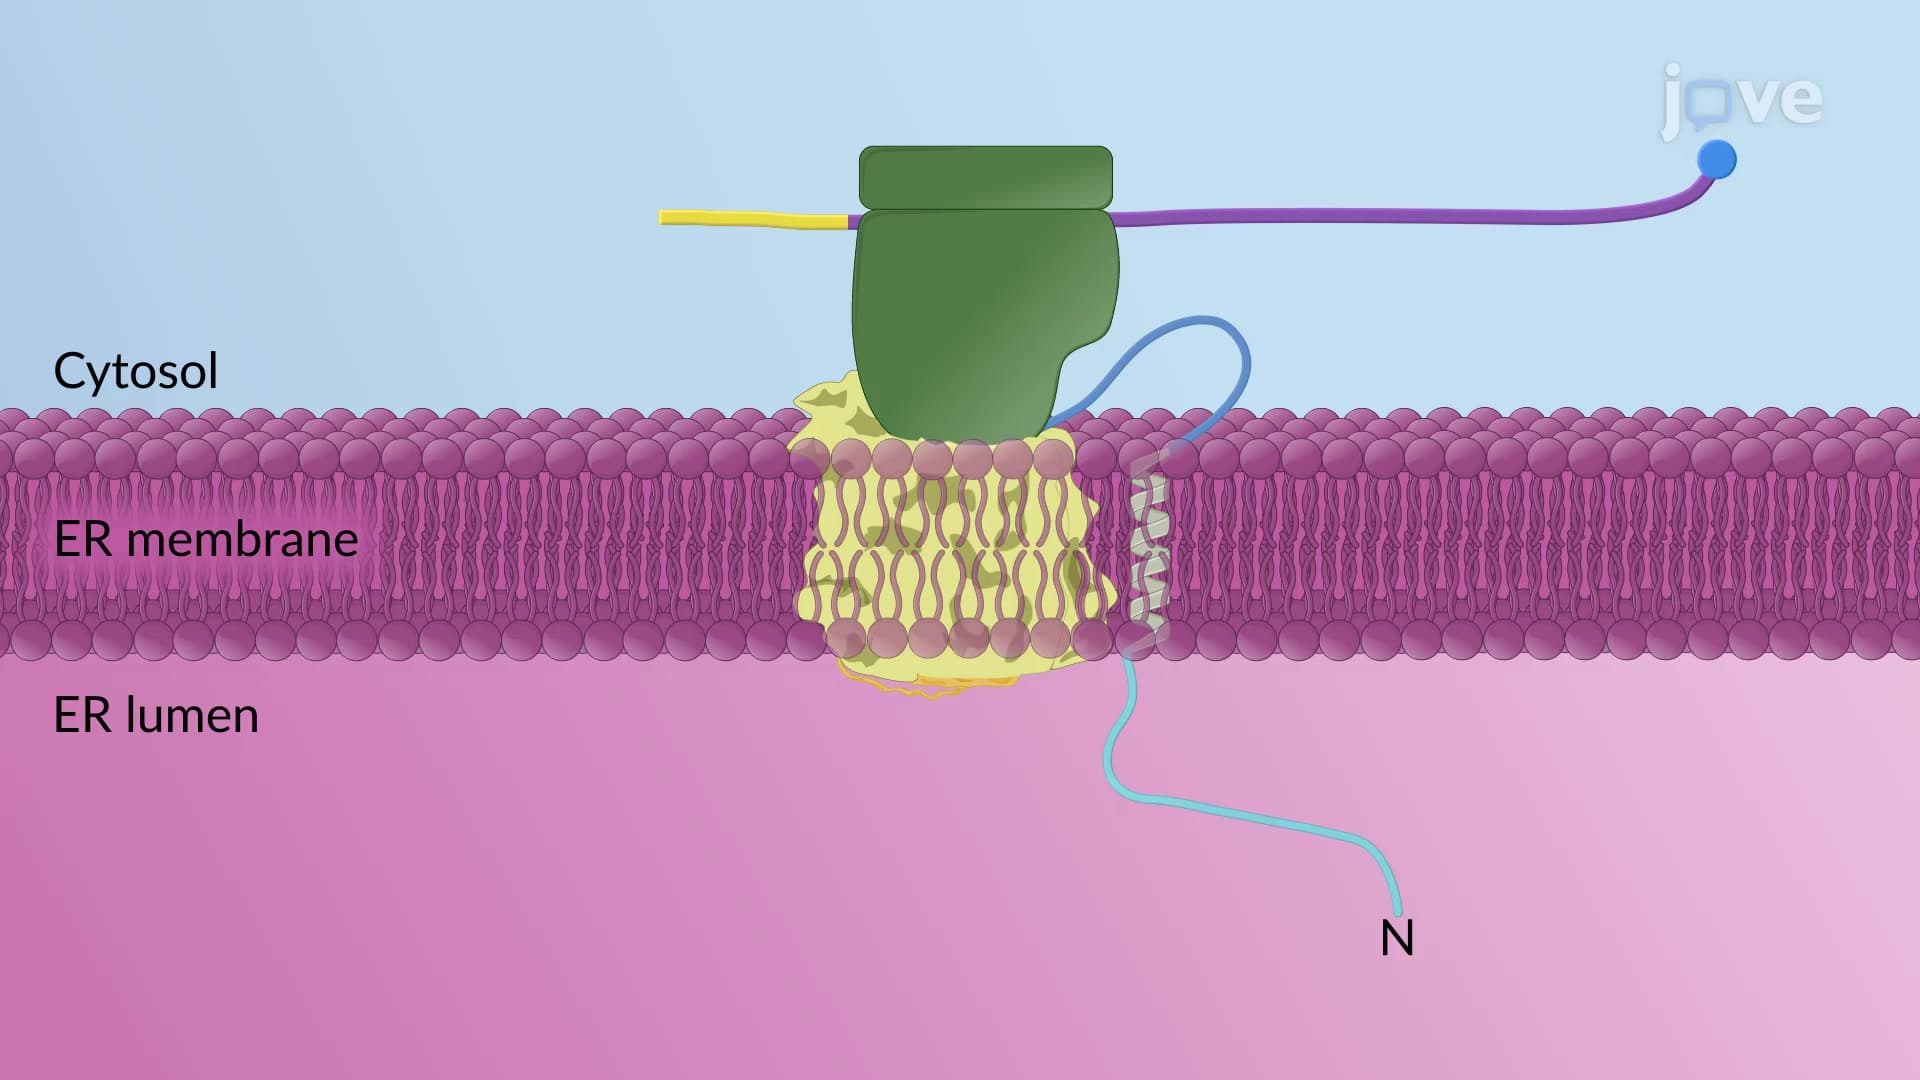
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:45
Tail-anchoring of Proteins in the ER Membrane
 01:28
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.
 01:22
Protein Transport to the Thylakoids
 01:26
Bacterial Translocation and Protein Secretion