Related Experiment Video
Updated: Oct 8, 2026
Simultaneous Measurement of Superoxide/Hydrogen Peroxide and NADH Production by Flavin-containing Mitochondrial Dehydrogenases
Published on: February 24, 2018
Order and disorder in mitochondrial aldehyde dehydrogenase
T D Hurley1, S Perez-Miller, H Breen
1Department of Biochemistry and Molecular Biology, Program in Medical Biophysics, Indiana University School of Medicine, 635 Barnhill Drive, 46202-5122, Indianapolis, IN, USA. thurley@iupui.edu

Abstract:
One of the most notable and currently unexplained features of the mitochondrial form of aldehyde dehydrogenase is its property of half-of-the-sites reactivity. An appropriate description of this phenomenon can be to consider this as the extreme example of negative cooperativity. This implies, therefore, that a pathway of communication must exist between active sites in order to convey the structural consequences of ligand binding. Data from four different structures of human ALDH2 collected during the past 2 years may shed some light on one possible pathway for the propagation of structural information. We recently published a 2.6 A structure of a binary complex between ALDH2 and NAD(+) in which the predominant conformation of the cofactor differed between different subunits in the structure. We now have three unpublished structures, a wild-type apo-enzyme structure at 2.25 A resolution, a wild-type structure complexed with NADH at 2.45 A resolution, and a site-directed mutant of ALDH2 where Arg475 is mutated to Gln, as an apo-enzyme to 2.75 A resolution. A detailed comparison of their structures reveals that a disorder-to-order transition occurs upon coenzyme binding in the area immediately surrounding the adenosine-binding site (residues 224-233 and 246-262). These residues correspond to the two helices that surround the adenine ring of the cofactor. Since the helix comprised of residues 246-262 contacts its dimer related helix across the subunit interface, this could induce as of yet unidentified subtle changes in structure that impair productive binding of the cofactor in the second subunit. The unique characteristics and three-dimensional structure of the R475Q variant of ALDH2 supports a role in subunit communication for these residues. This mutated enzyme displays positive cooperativity for cofactor binding. The structure of the apo-enzyme shows that the average thermal parameters for the residues involved in adenosine binding are drastically elevated as is a stretch of amino acids surrounding the site of mutation (residues 471-480). We hypothesize that cofactor binding displays a Hill coefficient of approximately 2 because binding of coenzyme to one subunit in a dimer orders the residues responsible for cofactor binding in the second, thus promoting binding. The difference between these alterations being positively versus negatively cooperative is likely related to the magnitude of the structural changes. Further work is in progress to confirm this hypothesis as it may shed light on the dominant effects of the E487K allelic variant, since Glu487 interacts with Arg475.
More Related Videos
 06:53
Visualization of Mitochondrial Respiratory Function using Cytochrome C Oxidase / Succinate Dehydrogenase (COX/SDH) Double-labeling Histochemistry
Published on: November 23, 2011
 05:27
Inner Mitochondrial Membrane Sensitivity to Na+ Reveals Partially Segmented Functional CoQ Pools
Published on: July 20, 2022
Related Concept Videos
 01:48
ATP Synthase: Mechanism
 01:39
Mitochondrial Protein Sorting
Most of these mitochondrial proteins are encoded by the nucleus and imported to the mitochondria as unfolded or loosely folded precursors. Mitochondrial precursors...
 01:46
Electron Transport Chain: Complex I and II
ROS generation is regulated and maintained at moderate levels necessary...
 01:43
Electron Transport Chain: Complex III and IV
 01:19
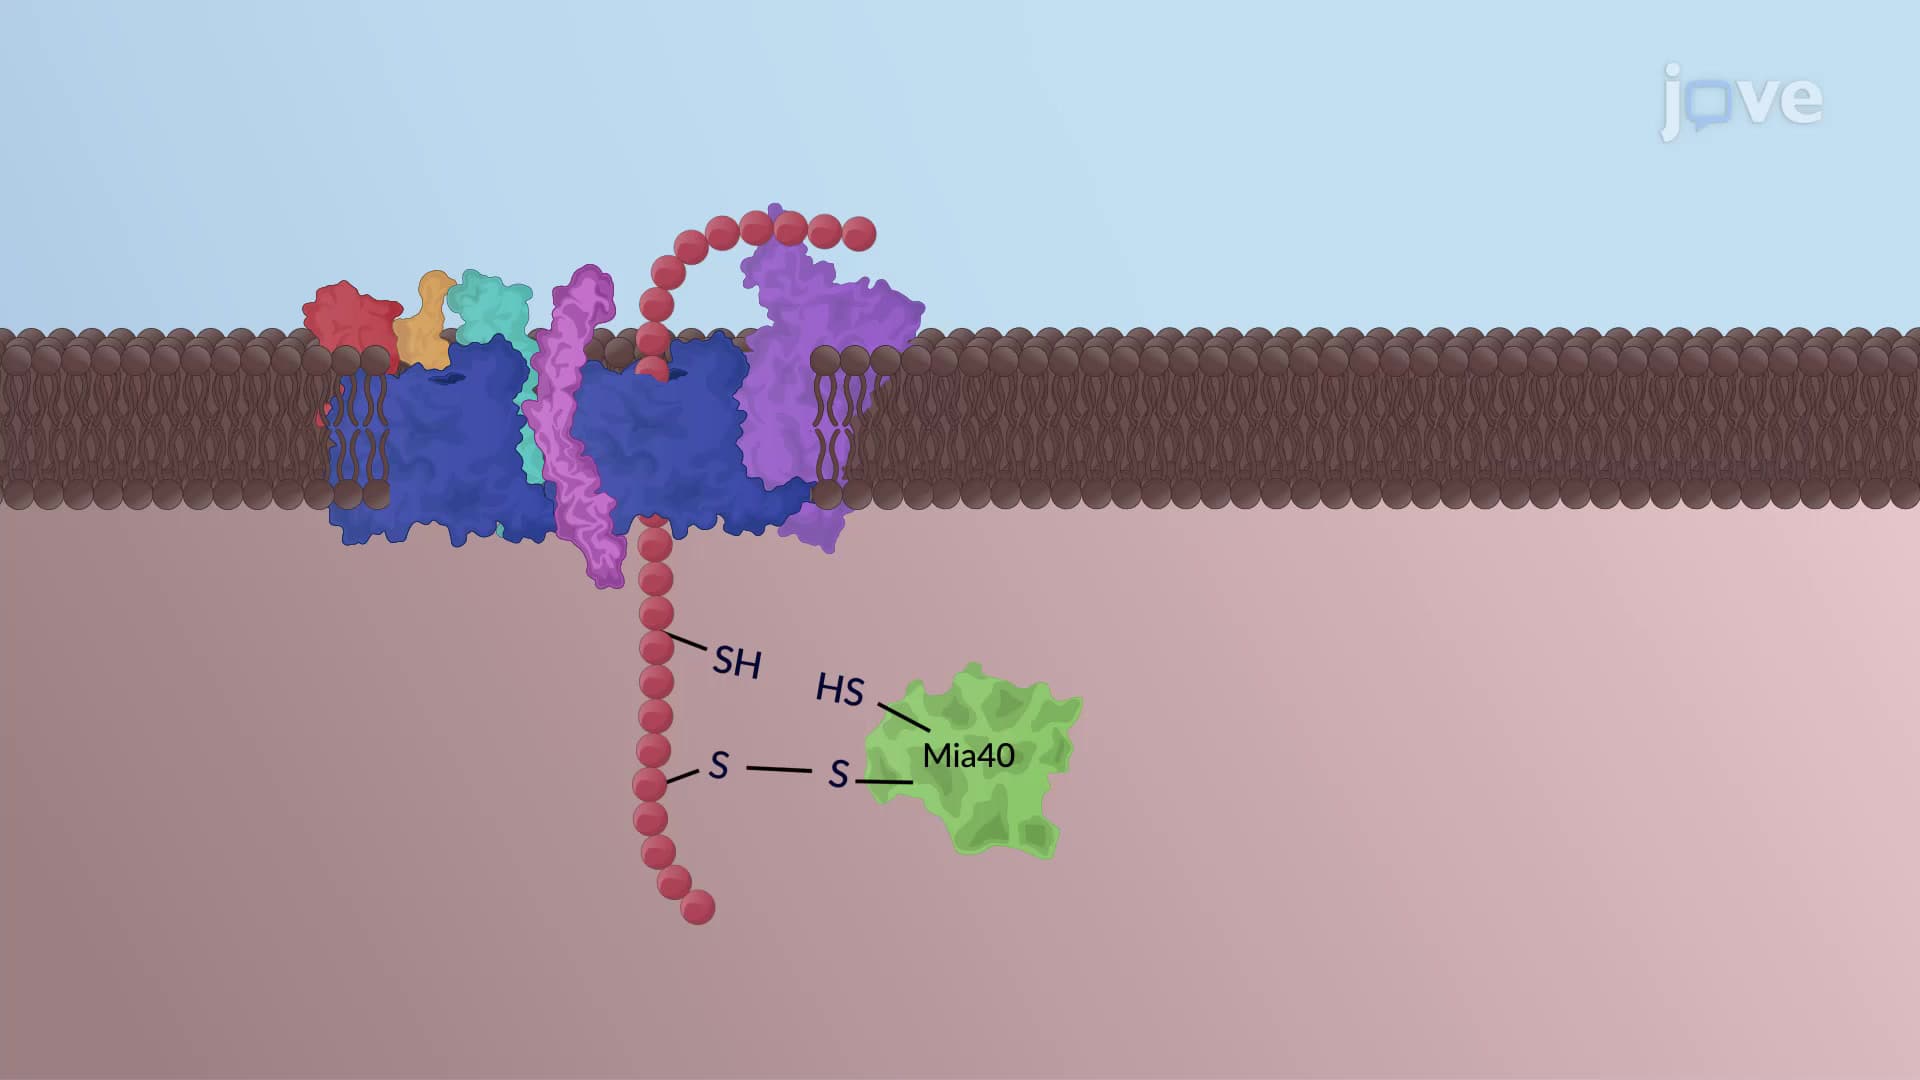
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:28
Electron Transport Chains
The ETC is comprised of...