Related Experiment Video
Updated: Aug 16, 2026

Isolation of F1-ATPase from the Parasitic Protist Trypanosoma brucei
Published on: January 22, 2019
F-ATPase: forced full rotation of the rotor despite covalent cross-link with the stator
K Gumbiowski1, D Cherepanov, M Muller
1Universität Osnabrück, FB Biologie, Abt. Biophysik, Barbarastrasse 11, 49069 Osnabrück, Germany.

Abstract:
In ATP synthase (F(O)F(1)-ATPase) ion flow through the membrane-intrinsic portion, F(O), drives the central "rotor", subunits c(10)epsilongamma, relative to the "stator" ab(2)delta(alphabeta)(3). This converts ADP and P(i) into ATP. Vice versa, ATP hydrolysis drives the rotation backwards. Covalent cross-links between rotor and stator subunits have been shown to inhibit these activities. Aiming at the rotary compliance of subunit gamma we introduced disulfide bridges between gamma (rotor) and alpha or beta (stator). We engineered cysteine residues into positions located roughly at the "top," "center," and "bottom" parts of the coiled-coil portion of gamma and suitable residues on alpha or beta. This part of gamma is located at the center of the (alphabeta)(3) domain with its C-terminal part at the top of F(1) and the bottom part close to the F(O) complex. Disulfide bridge formation under oxidizing conditions was quantitative as shown by SDS-polyacrylamide gel electrophoresis and immunoblotting. As expected both the ATPase activities and the yield of rotating subunits gamma dropped to zero when the cross-link was formed at the center (gammaL262C <--> alphaA334C) and bottom (gammaCys(87) <--> betaD380C) positions. But much to our surprise disulfide bridging impaired neither ATP hydrolysis activity nor the full rotation of gamma and the enzyme-generated torque of oxidized F(1), which had been engineered at the top position (gammaA285C <--> alphaP280C). Apparently the high torque of this rotary engine uncoiled the alpha-helix and forced amino acids at the C-terminal portion of gamma into full rotation around their dihedral (Ramachandran) angles. This conclusion was supported by molecular dynamics simulations: If gammaCys(285)-Val(286) are attached covalently to (alphabeta)(3) and gammaAla(1)-Ser(281) is forced to rotate, gammaGly(282)-Ala(284) can serve as cardan shaft.
Related Concept Videos
 01:08
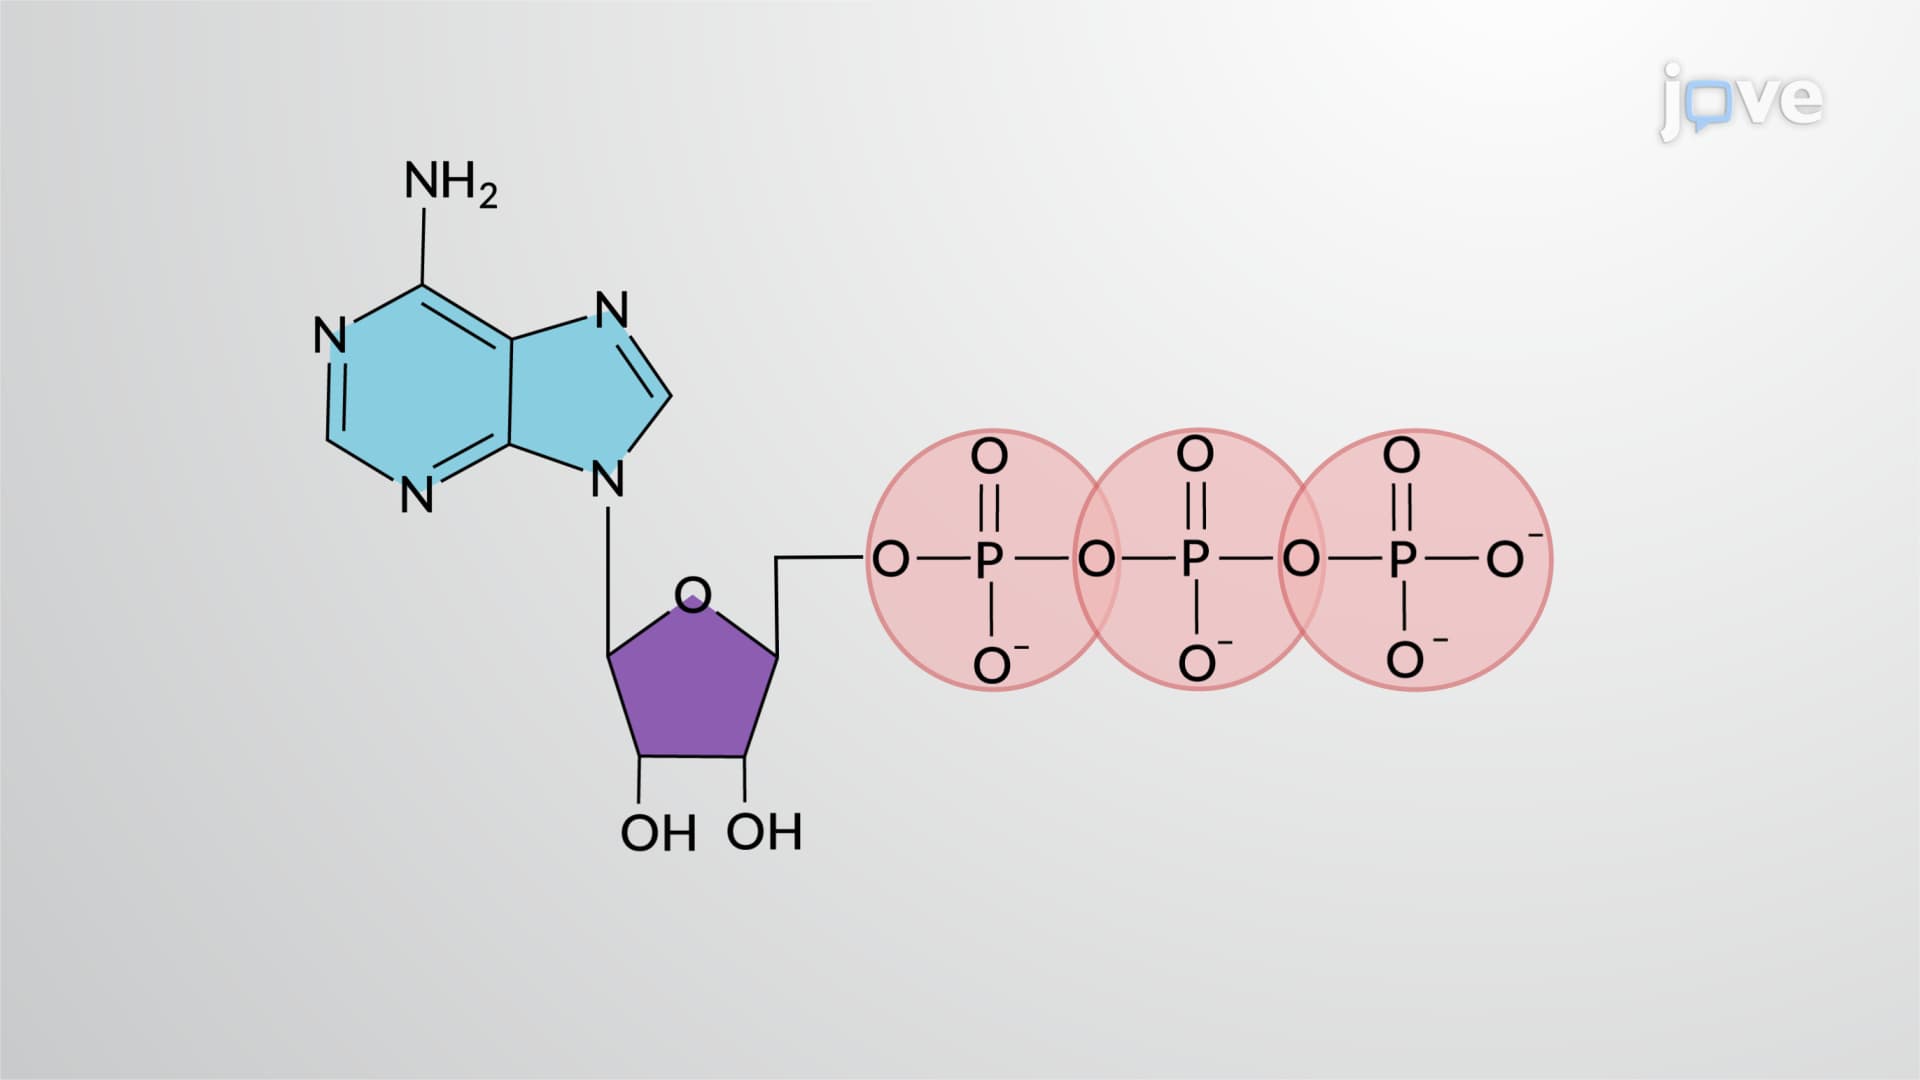
Hydrolysis of ATP
If one phosphate group is removed, a molecule of ADP—adenosine diphosphate—remains, along with inorganic phosphate. ADP can be further hydrolyzed to AMP—adenosine monophosphate—by the removal of a second...
 01:27
ATP Driven Pumps I: An Overview
There are four main types of ATP-driven pumps - P-type, V-type, F-type, and ABC transporter. All these pumps are of varying complexities and are...
 01:48
ATP Synthase: Mechanism
 01:18
ATP Synthase: Structure
 01:34
ATP Driven Pumps II: P-type Pumps
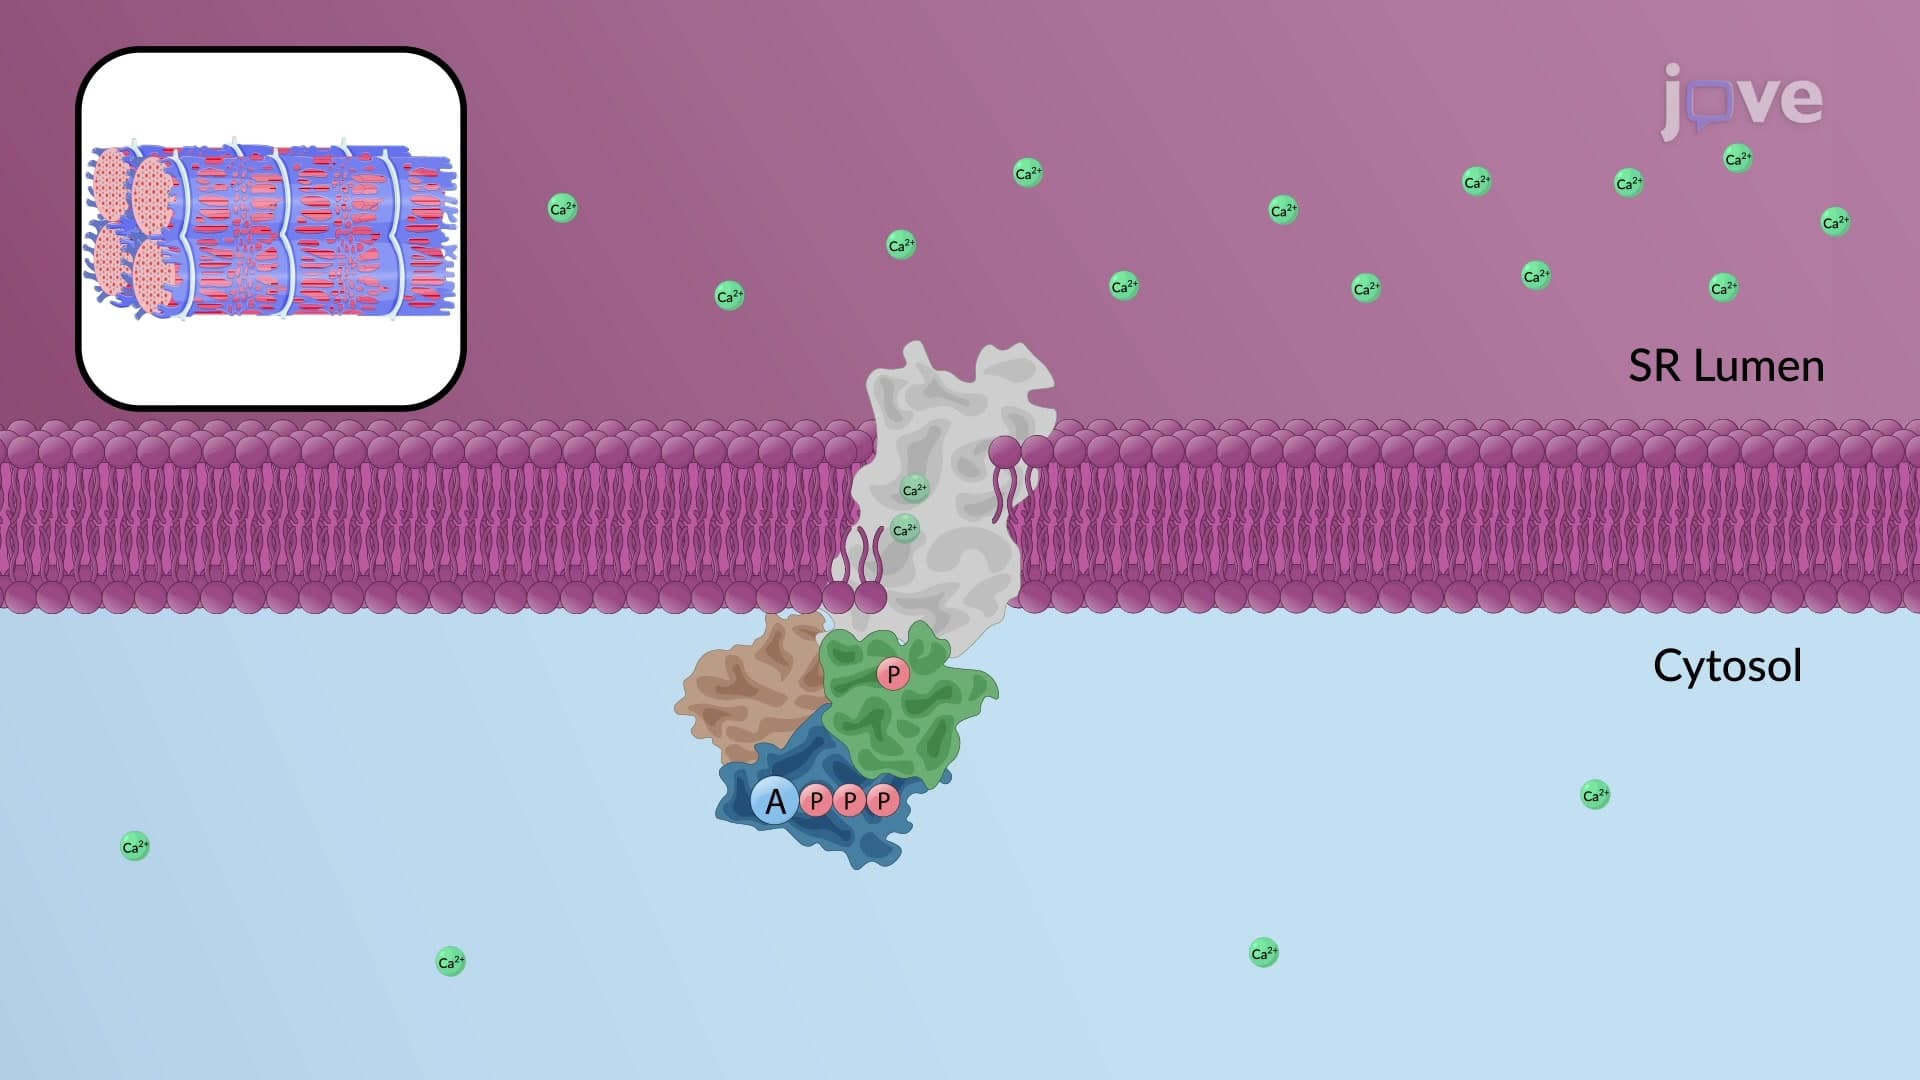
A typical P-type pump has three cytosolic domains: nucleotide-binding (N), phosphorylation (P), and activator (A) domains. These domains are connected to the membrane-spanning helices by short amino acid segments. ATP hydrolysis and covalent phosphoenzyme intermediate formation are crucial parts of the catalytic cycle. At the highly...
 01:30
ATP Driven Pumps III: V-type Pumps
The peripheral or cytosolic V1 domain with eight subunits is involved in ATP hydrolysis. The integral or transmembrane V0 domain containing at least five subunits...