Related Experiment Video
Updated: Oct 3, 2026

Detection of Toxin Translocation into the Host Cytosol by Surface Plasmon Resonance
Published on: January 3, 2012
Translocation activity of C-terminal domain of pestivirus Erns and ribotoxin L3 loop
1Department of Mammalian Virology, Institute for Animal Science and Health (ID-Lelystad), P.O. Box 65, 8200 AB, Lelystad, The Netherlands. j.p.m.langedijk.id.wag-ur.nl

Abstract:
The pestivirus envelope glycoprotein E(rns) has RNase activity and therefore was suspected to enter cells to cleave RNA. The protein contains an RNase domain with a C-terminal extension, which shows homology with a membrane-active peptide. The modular architecture and the C-terminal homology suggested that the C terminus could be responsible for the presumed translocation. Peptides corresponding to the C-terminal domain of E(rns) and also the homologous L3 loop of ribotoxin II were indeed able to translocate across the eukaryotic cell membrane and were targeted to the nucleoli. The entire E(rns) protein was also able to translocate into the cell. Furthermore, other labeled proteins and even active enzymes could be transported inside the cell when they were attached to the C-terminal E(rns) peptide. Translocation was energy-independent and not mediated by a protein receptor. The peptides showed no specificity for cell type or species.
More Related Videos
 09:13
Using Reverse Genetics to Manipulate the NSs Gene of the Rift Valley Fever Virus MP-12 Strain to Improve Vaccine Safety and Efficacy
Published on: November 1, 2011
 10:11
Modeling The Lifecycle Of Ebola Virus Under Biosafety Level 2 Conditions With Virus-like Particles Containing Tetracistronic Minigenomes
Published on: September 27, 2014
Related Concept Videos
 03:08
LTR Retrotransposons
The internal coding region of LTR retrotransposons and their mechanism of transposition closely resembles a...
 01:20
Cotranslational Protein Translocation
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
 01:26
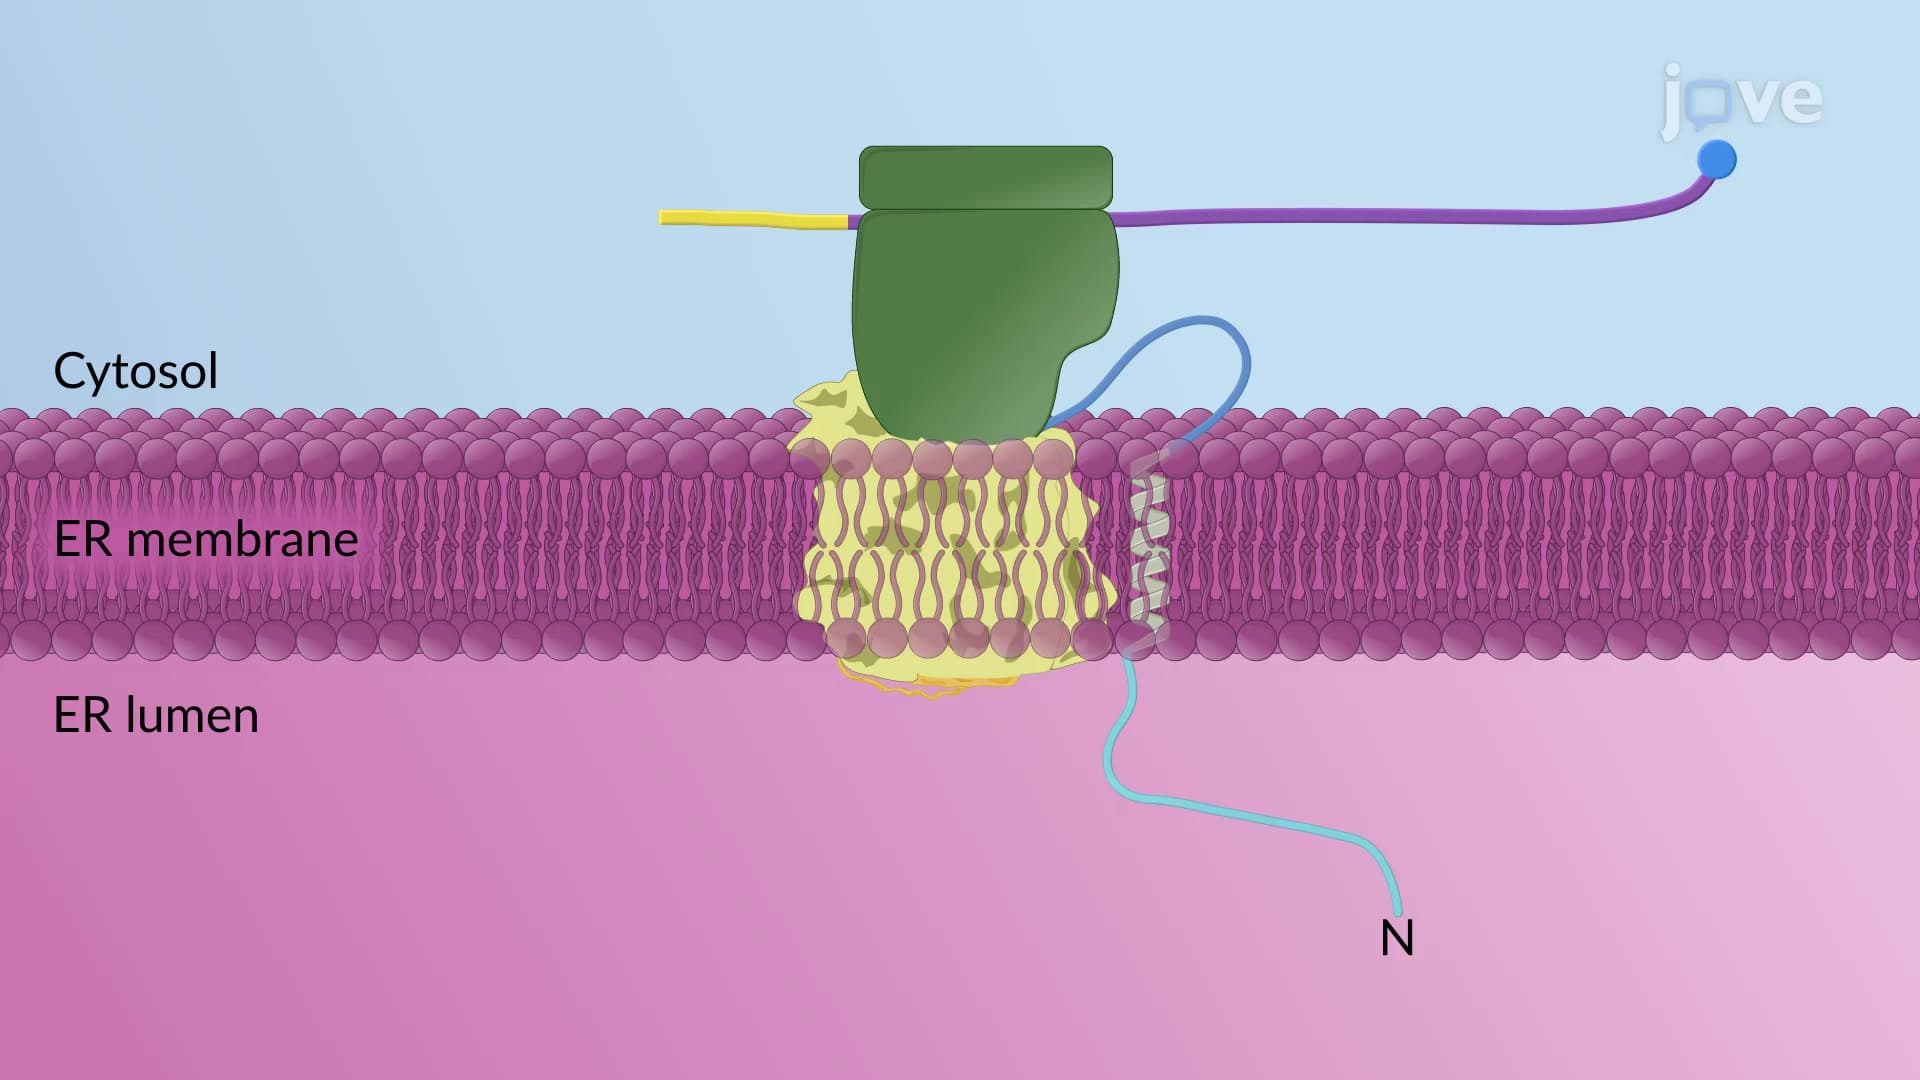
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:27
Post-translational Translocation of Proteins to the RER
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
 03:18
Non-LTR Retrotransposons
 01:28
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.