Related Experiment Video
Updated: Aug 11, 2026

From Constructs to Crystals – Towards Structure Determination of β-barrel Outer Membrane Proteins
Published on: July 4, 2016
Monomer-monomer interactions drive the prepore to pore conversion of a beta-barrel-forming cholesterol-dependent
Eileen M Hotze1, Alejandro P Heuck, Daniel M Czajkowsky
1Department of Microbiology and Immunology, the University of Oklahoma Health Sciences Center, Oklahoma City, Oklahoma 73104, USA.

Abstract:
Perfringolysin O (PFO), a cholesterol-dependent cytolysin, forms large oligomeric pore complexes comprised of up to 50 PFO molecules. In the present studies a mutant of PFO (PFO(Y181A)) has been identified that traps PFO in a multimeric prepore complex that cannot insert its transmembrane beta-hairpins and therefore cannot form a pore. Remarkably, PFO(Y181A) can be induced to insert its transmembrane beta-hairpins if functional PFO is incorporated into the PFO(Y181A) oligomeric prepore complex. Furthermore, the transition from prepore to pore appears to be an "all or none" process; partial insertion of the transmembrane beta-barrel does not occur. Therefore, cooperative interactions between the monomers of the prepore drive the prepore to pore conversion that results in the formation of the transmembrane beta-barrel.
Insights
A mutant perfringolysin O (PFO) protein gets stuck in a prepore complex. Adding normal PFO triggers the mutant to form a complete pore, showing cooperative binding is key.
Area of Science:
- Microbiology
- Biochemistry
- Molecular Biology
Background:
- Perfringolysin O (PFO) is a cholesterol-dependent cytolysin.
- PFO forms large oligomeric pore complexes involving up to 50 PFO molecules.
Purpose of the Study:
- To investigate the mechanism of PFO pore formation.
- To identify mutations that trap PFO in a prepore state.
- To understand the transition from prepore to pore complex.
Main Methods:
- Site-directed mutagenesis to create PFO(Y181A) mutant.
- Biochemical assays to analyze PFO oligomerization and pore formation.
- Characterization of the PFO(Y181A) prepore complex.
Main Results:
- A PFO mutant (PFO(Y181A)) was identified that forms stable prepore complexes.
- The PFO(Y181A) prepore complex cannot insert transmembrane beta-hairpins.
- Incorporation of functional PFO into the PFO(Y181A) prepore induces beta-hairpin insertion and pore formation.
- The prepore to pore transition is an 'all or none' process, with no partial insertion observed.
Conclusions:
- Cooperative interactions between PFO monomers drive the transition from prepore to pore.
- This cooperative mechanism is essential for the formation of the transmembrane beta-barrel structure.
- The PFO(Y181A) mutant serves as a valuable tool for studying the PFO pore assembly pathway.
Related Concept Videos
 01:23
Membrane Fluidity
 01:26
Membrane Fluidity
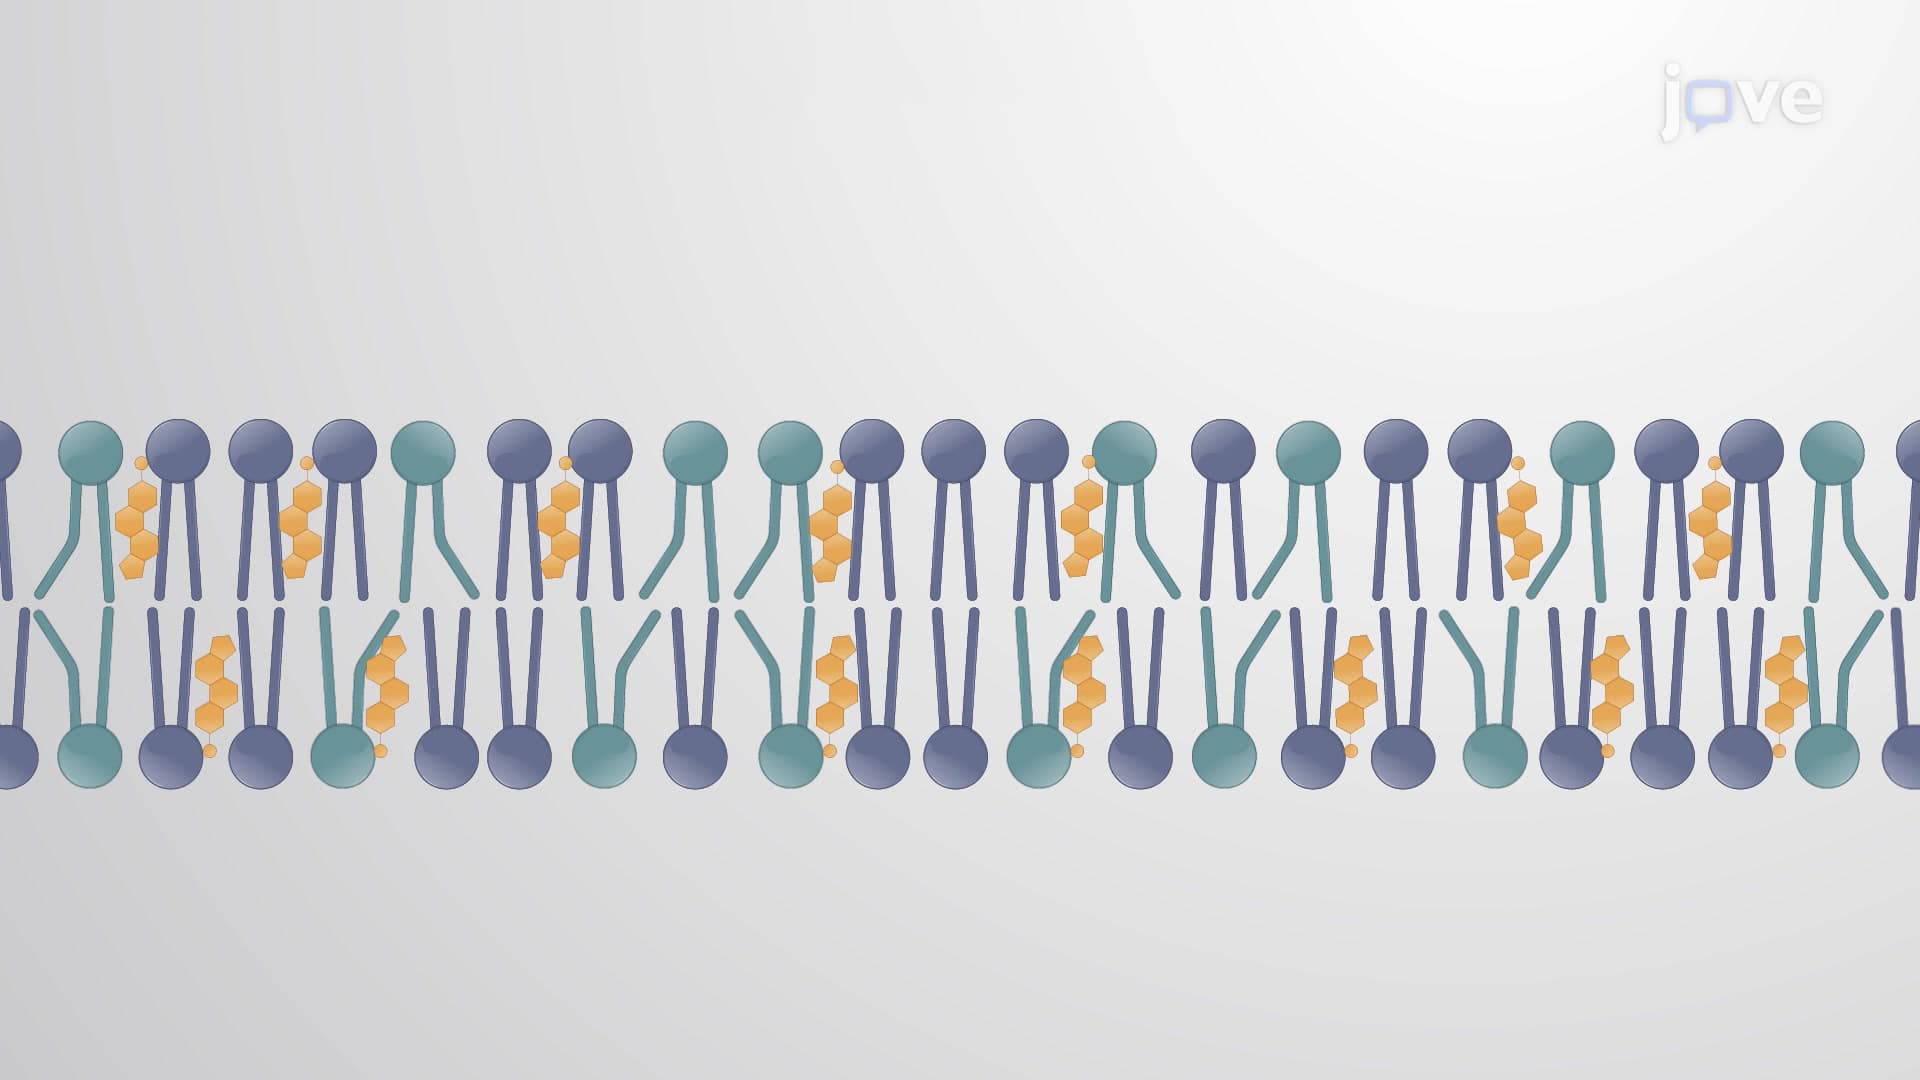
Mosaic nature of the membrane
The mosaic characteristic of the membrane helps the plasma membrane remain fluid. The integral proteins and lipids exist as separate but loosely-attached molecules in the membrane. The membrane is a relatively...
 01:12
Porin Insertion in the Outer Mitochondrial Membrane
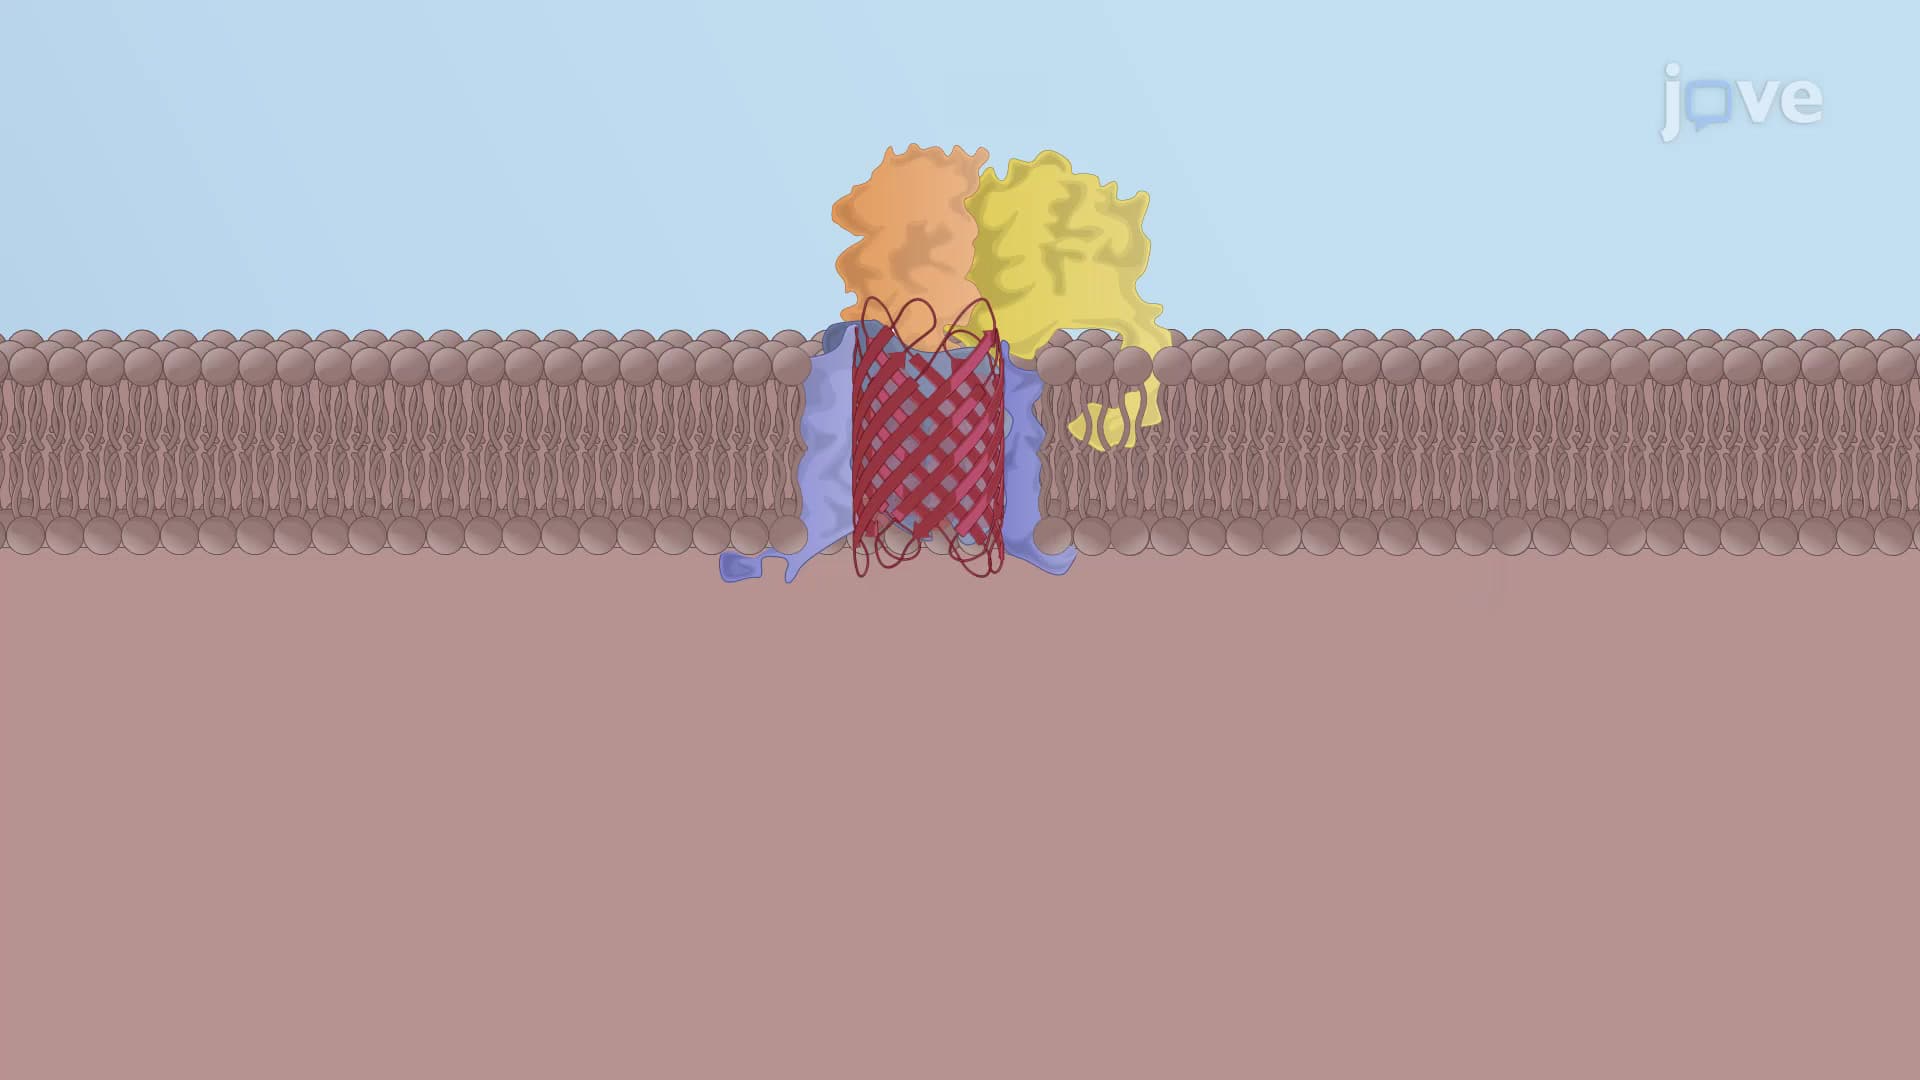
Three models describe the assembly of porins by the SAM complex and their insertion into the outer membrane. Model 1 suggests that porins are assembled outside the SAM channel as the...
 01:09
Multi-pass Transmembrane Proteins and β-barrels
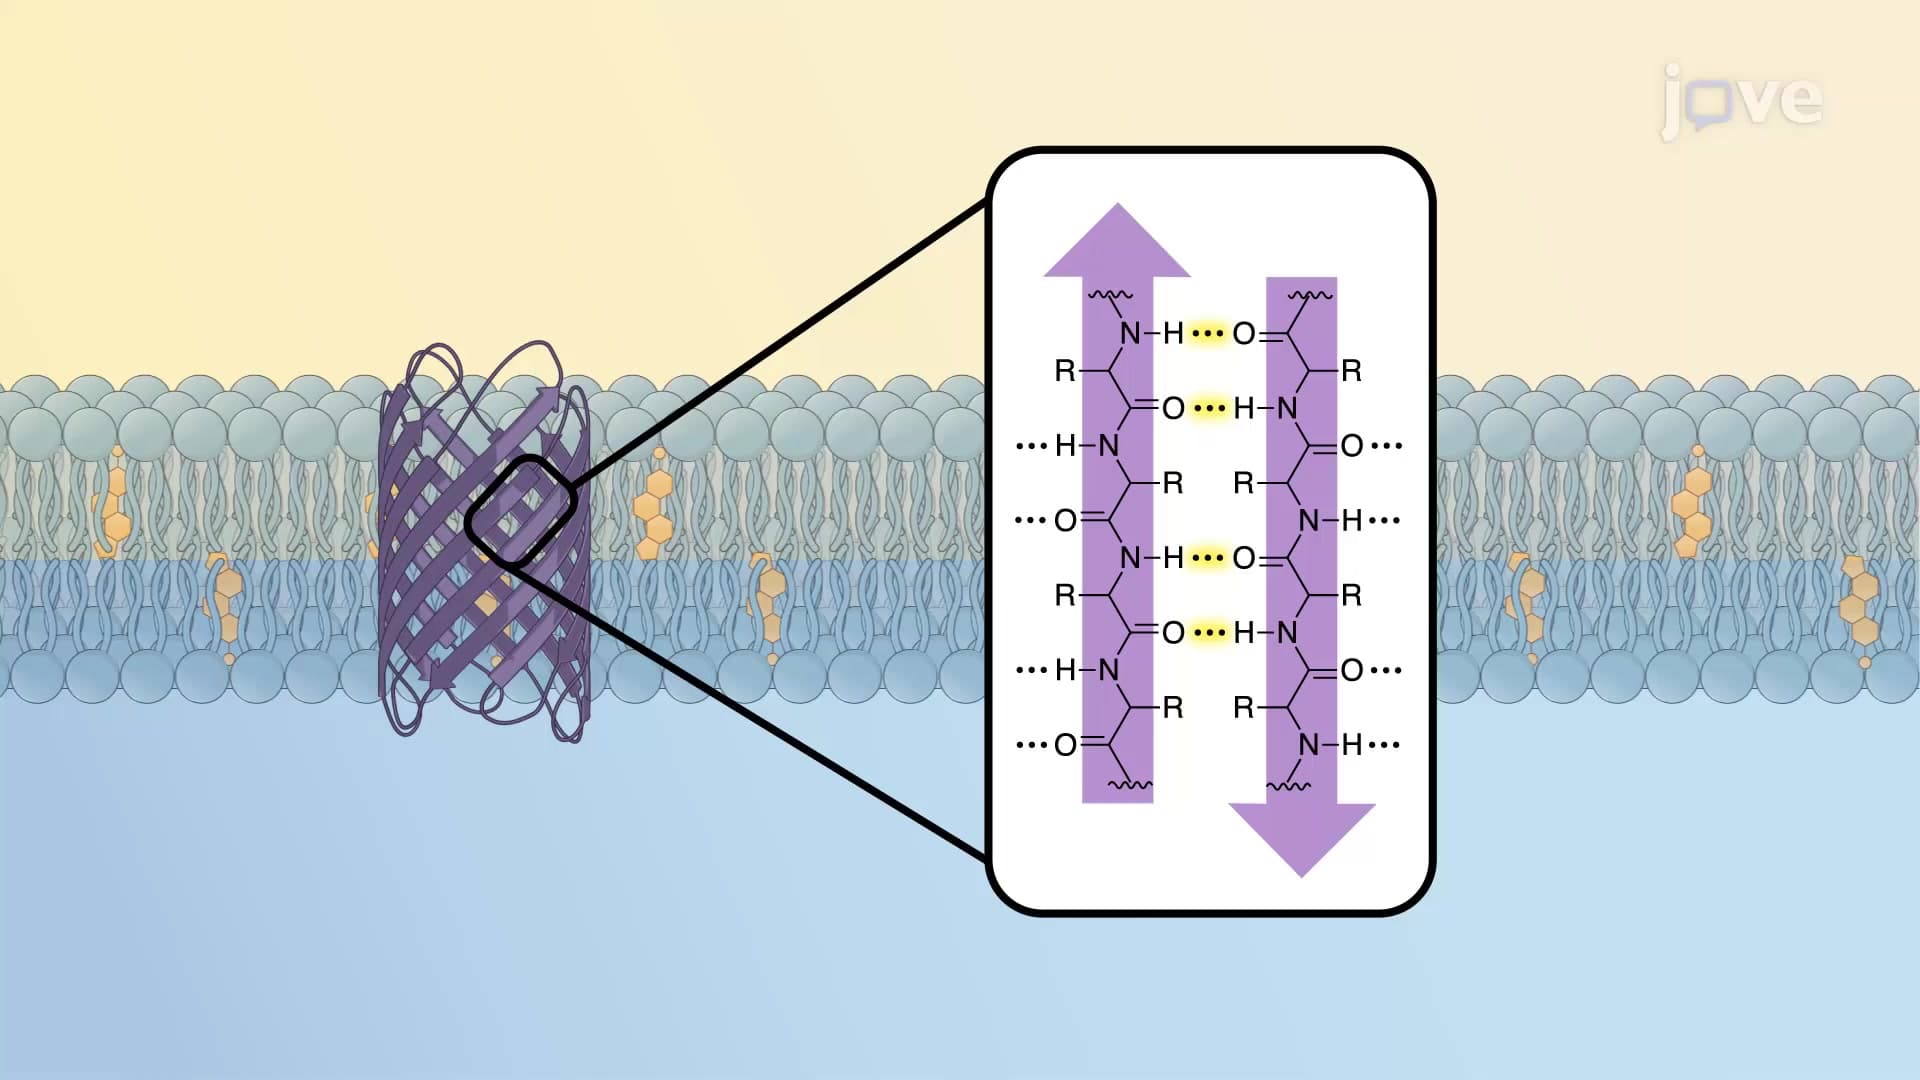
α-Helix containing multi-pass transmembrane proteins
Multi-pass transmembrane proteins such as G-protein-linked receptors (GPCRs) and...
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...
 01:21
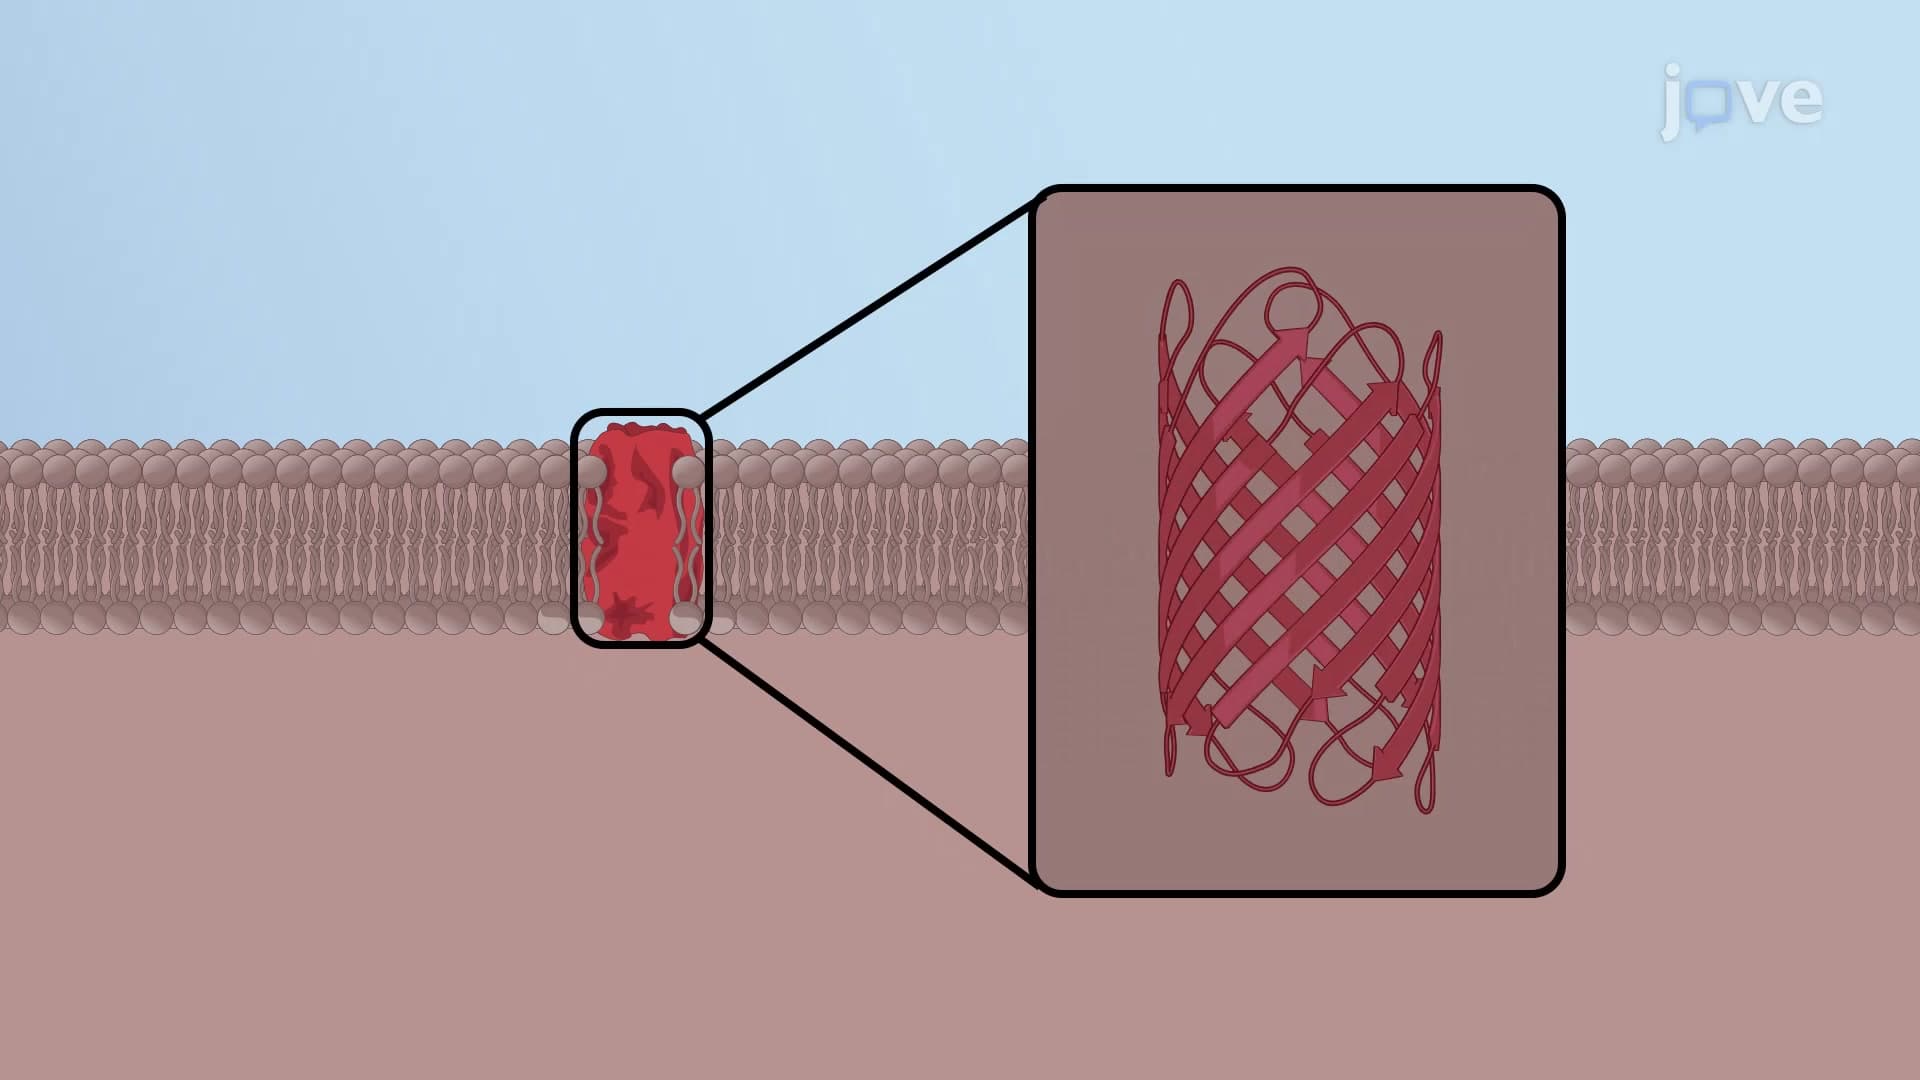
Structure of Porins