Related Experiment Video
Updated: Sep 29, 2026
Identification of Hemolytic and Phospholipase Activity in Crude Extracts from Sea Anemones by Straightforward Bioassays
Published on: March 29, 2022
Two-step membrane binding by Equinatoxin II, a pore-forming toxin from the sea anemone, involves an exposed aromatic
Qi Hong1, Ion Gutierrez-Aguirre, Ariana Barlic
1School of Biochemistry and Genetics, University of Newcastle upon Tyne, Framlington Place, United Kingdom.

Abstract:
Equinatoxin II (EqtII) belongs to a unique family of 20-kDa pore-forming toxins from sea anemones. These toxins preferentially bind to membranes containing sphingomyelin and create cation-selective pores by oligomerization of 3-4 monomers. In this work we have studied the binding of EqtII to lipid membranes by the use of lipid monolayers and surface plasmon resonance (SPR). The binding is a two-step process, separately mediated by two regions of the molecule. An exposed aromatic cluster involving tryptophans 112 and 116 mediates the initial attachment that is prerequisite for the next step. Steric shielding of the aromatic cluster or mutation of Trp-112 and -116 to phenylalanine significantly reduces the toxin-lipid interaction. The second step is promoted by the N-terminal amphiphilic helix, which translocates into the lipid phase. The two steps were distinguished by the use of a double cysteine mutant having the N-terminal helix fixed to the protein core by a disulfide bond. The kinetics of membrane binding derived from the SPR experiments could be fitted to a two-stage binding model. Finally, by using membrane-embedded quenchers, we showed that EqtII does not insert deeply in the membrane. The first step of the EqtII binding is reminiscent of the binding of the evolutionarily distant cholesterol-dependant cytolysins, which share a similar structural motif in the membrane attachment domain.
More Related Videos
 11:44
Synthesis and Structure Determination of µ-Conotoxin PIIIA Isomers with Different Disulfide Connectivities
Published on: October 2, 2018
 10:31
A Liposome Membrane Permeability Assay for Investigating the Effects of Phosphatidylinositol Phosphate Groups on Membranotropic Action of Venom PLA2
Published on: September 26, 2025
Related Concept Videos
 01:09
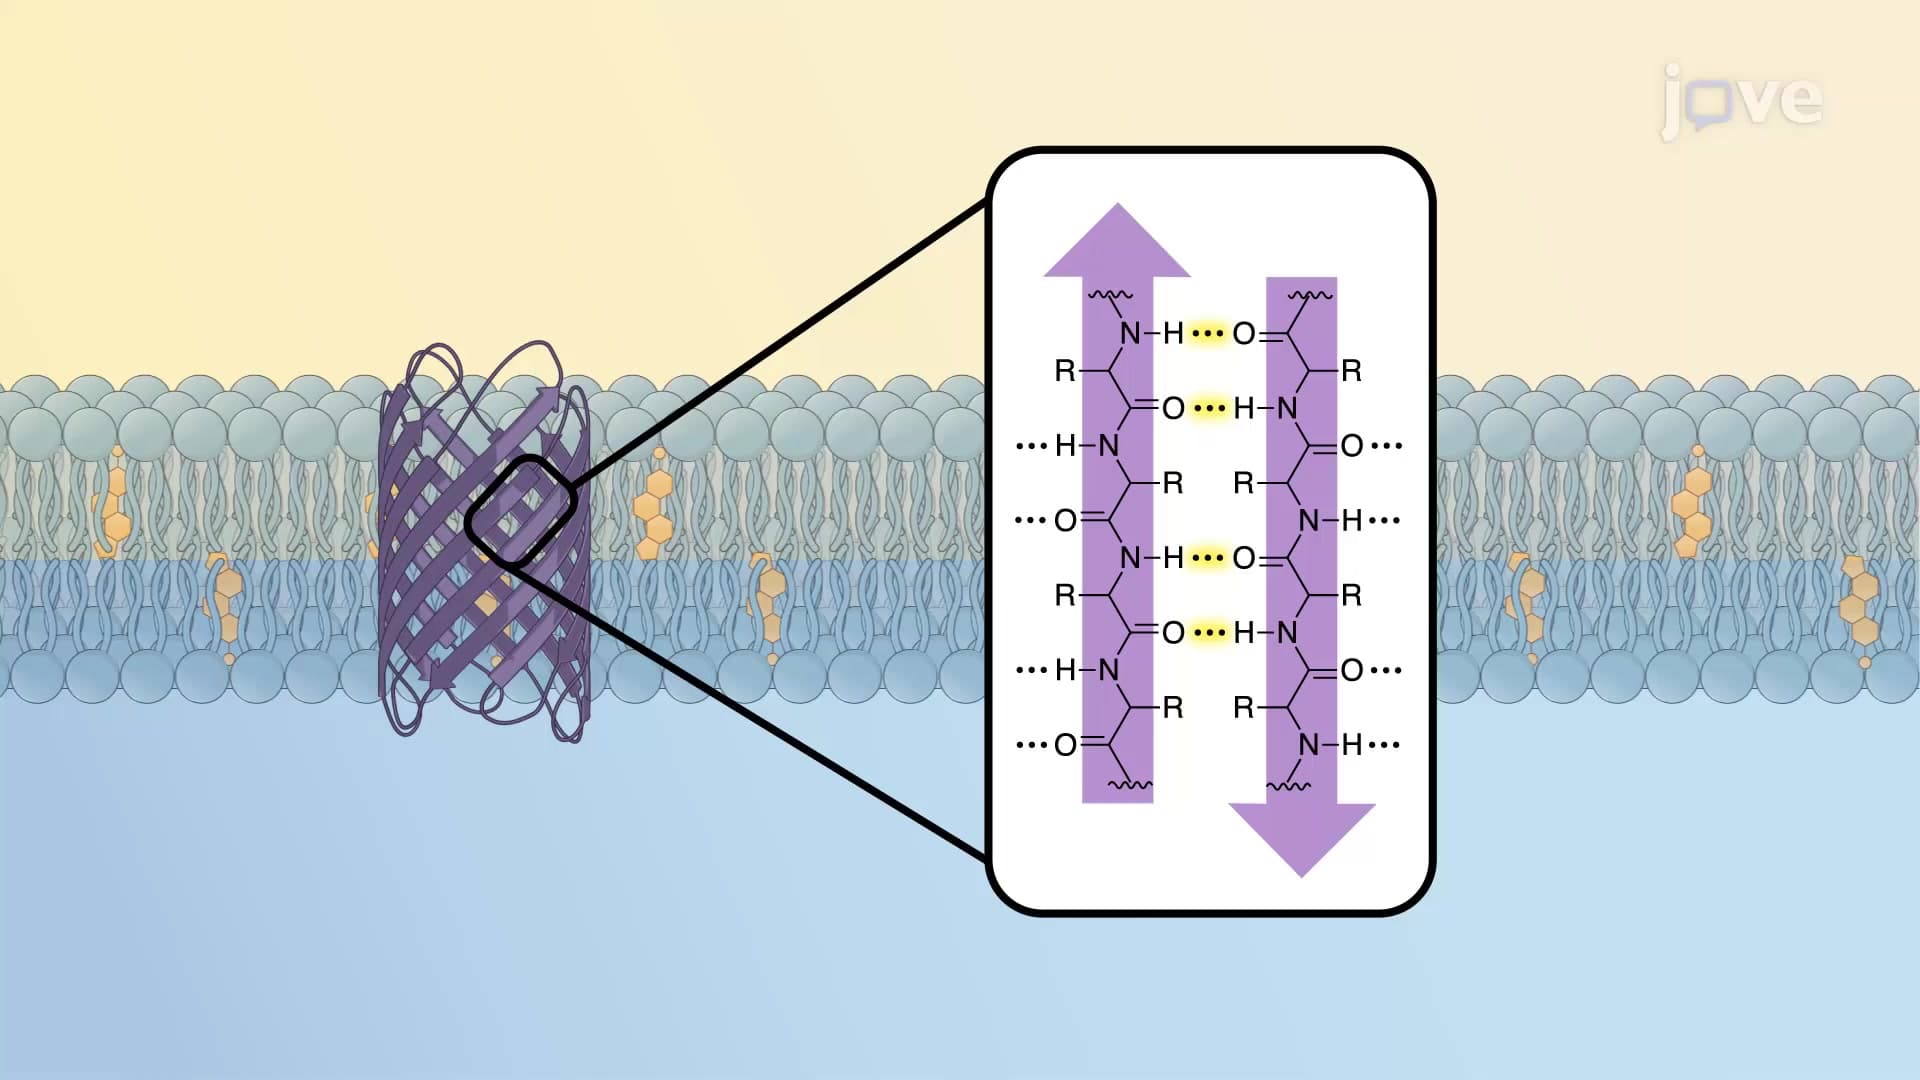
Multi-pass Transmembrane Proteins and β-barrels
α-Helix containing multi-pass transmembrane proteins
Multi-pass transmembrane proteins such as G-protein-linked receptors (GPCRs) and...
 01:26
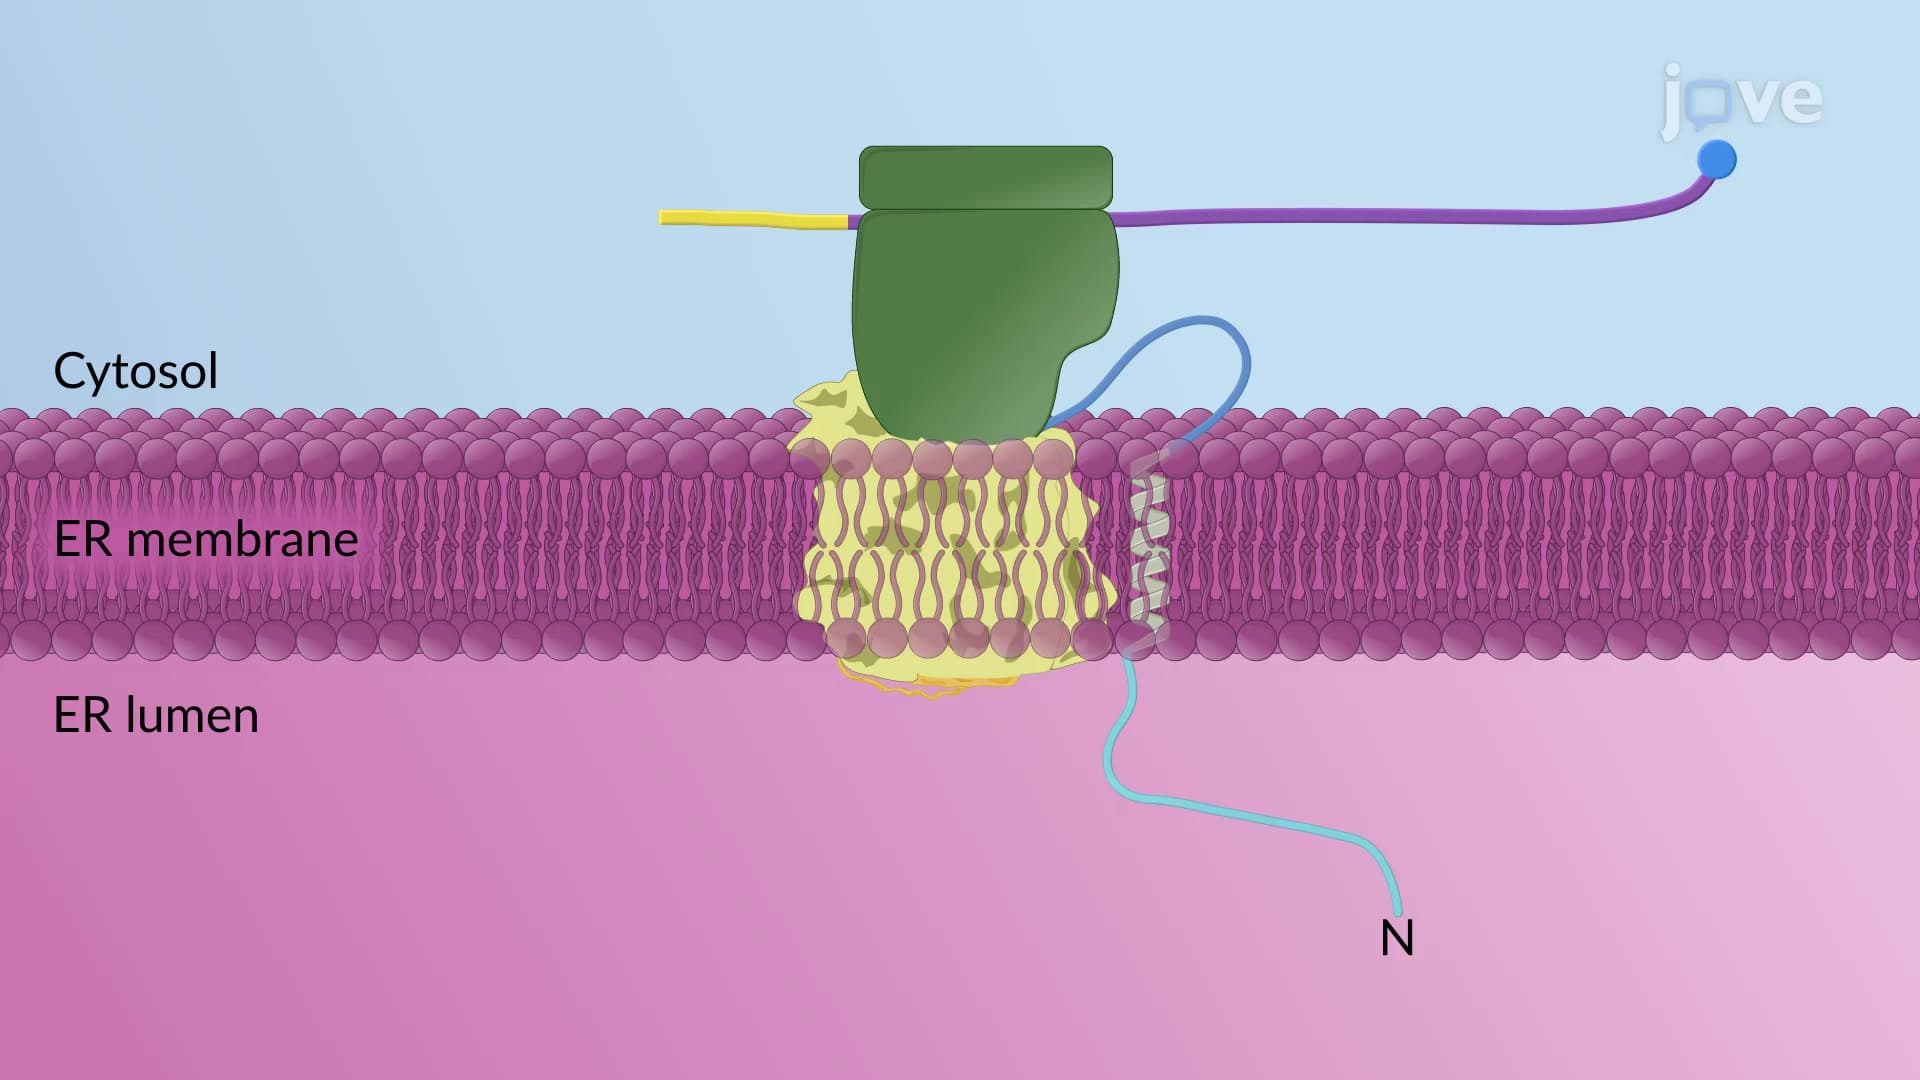
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:32
Pinching-off of Coated Vesicles
 01:12
Clathrin Coated Vesicles
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
 01:21
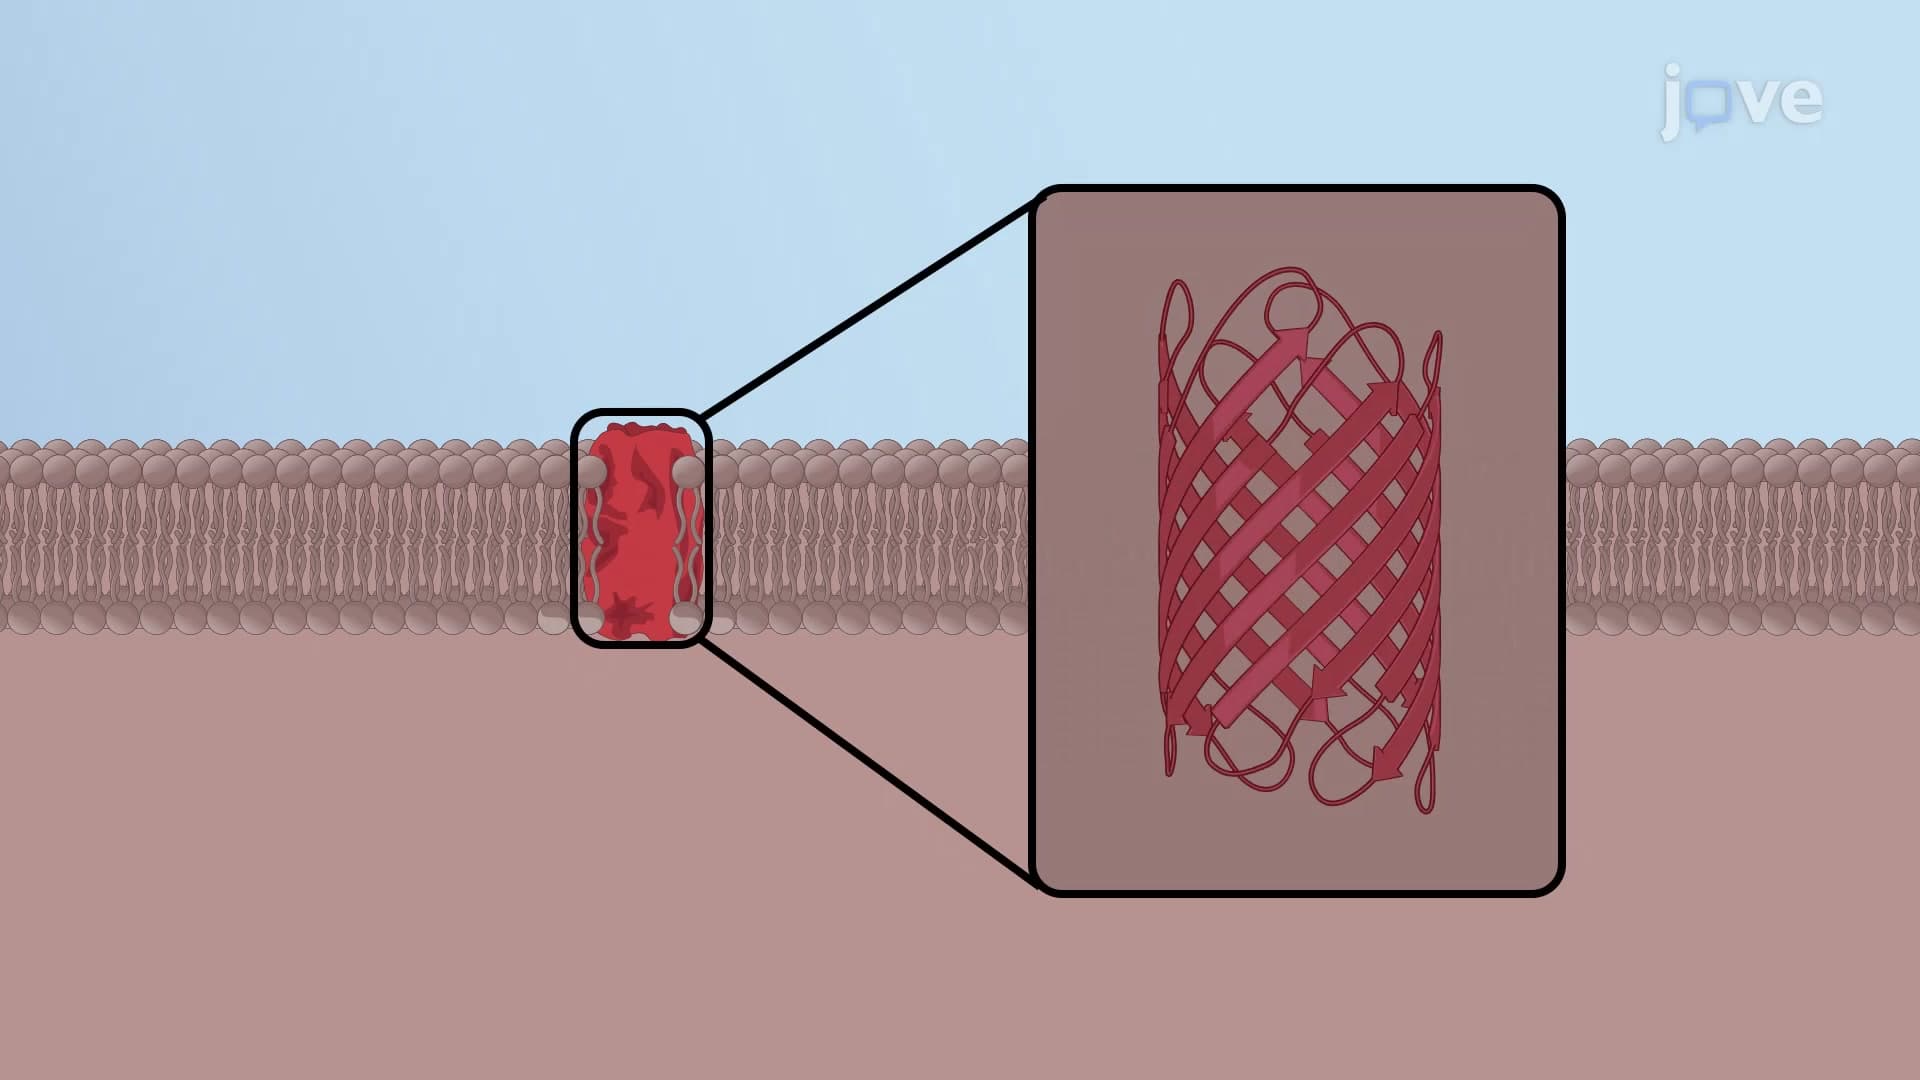
Structure of Porins