Related Experiment Video
Updated: Sep 27, 2026

Fabrication and Characterization of Colorectal Cancer Organoids from SW1222 Cell Line in Ultrashort Self-Assembling Peptide Matrix
Published on: May 3, 2024
Self-assembly is important for TIP47 function in mannose 6-phosphate receptor transport
Paul M Sincock1, Ian G Ganley, Jeffrey P Krise
1Department of Biochemistry, Stanford University School of Medicine, Stanford, CA 94305-5307, USA.

Abstract:
TIP47 (tail-interacting protein of 47 kDa) binds to the cytoplasmic domains of mannose 6-phosphate receptors and is required for their transport from endosomes to the trans-Golgi network in vitro and in living cells. TIP47 occurs in cytosol as an oligomer; it chromatographs with an apparent mass of approximately 300 kDa and displays an S-value of approximately 13. Recombinant TIP47 forms homo-oligomers that are likely to represent hexamers, as determined by chemical cross-linking. Removal of TIP47 residues 1-151 yields a protein that behaves as a monomer upon gel filtration, yet is fully capable of binding mannose 6-phosphate receptor cytoplasmic domains. The presence of an oligomerization domain in the N-terminus of TIP47 was confirmed by expression of N-terminal residues 1-133 or 1-257 in mammalian cells. Co-expression of full-length TIP47 with either of these fragments led to the formation of higher-order aggregates of wild-type TIP47. Furthermore, the N-terminal domains expressed alone also occurred as oligomers. These studies reveal an N-terminal oligomerization domain in TIP47, and show that oligomerization is not required for TIP47 recognition of mannose 6-phosphate receptors. However, oligomerization is required for TIP47 stimulation of mannose 6-phosphate receptor transport from endosomes to the trans-Golgi in vivo.
Insights
Tail-interacting protein of 47 kDa (TIP47) binds mannose 6-phosphate receptors. Its N-terminal domain drives TIP47 oligomerization, essential for receptor transport but not binding.
Area of Science:
- Cell Biology
- Molecular Biology
- Protein Trafficking
Background:
- Mannose 6-phosphate receptors (MPRs) mediate lysosomal enzyme targeting.
- Tail-interacting protein of 47 kDa (TIP47) interacts with MPR cytoplasmic domains.
- TIP47 is implicated in MPR transport from endosomes to the trans-Golgi network.
Purpose of the Study:
- To investigate the role of TIP47 oligomerization in MPR binding and transport.
- To identify the domain responsible for TIP47 oligomerization.
- To elucidate the functional significance of TIP47 oligomerization in cellular trafficking.
Main Methods:
- In vitro binding assays using recombinant TIP47 fragments.
- Gel filtration and chemical cross-linking to assess TIP47 oligomeric state.
- Mammalian cell expression systems to study protein interactions and aggregation.
- In vivo transport assays to evaluate MPR trafficking.
Main Results:
- TIP47 exists as a homo-oligomer (likely hexamer) in the cytosol.
- An N-terminal domain (residues 1-151) is responsible for TIP47 oligomerization.
- TIP47 oligomerization is not required for binding to MPRs.
- TIP47 oligomerization is essential for stimulating MPR transport in vivo.
Conclusions:
- TIP47 possesses an N-terminal oligomerization domain.
- Oligomerization is separable from MPR binding function.
- TIP47 oligomerization is a critical regulatory step for MPR-mediated protein transport.
Related Concept Videos
 01:24
Oligosaccharide Assembly
Multiple sugar molecules that may or may...
 01:33
Coat Assembly and GTPases
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
 01:30
Assembly of Signaling Complexes
Interaction domains in cell signaling
Interaction domains recognize exposed features of their binding partners containing post-translationally modified sequences,...
 02:41
Protein Complex Assembly
Many viruses self-assemble into a fully functional unit using the infected host cell to...
 01:29
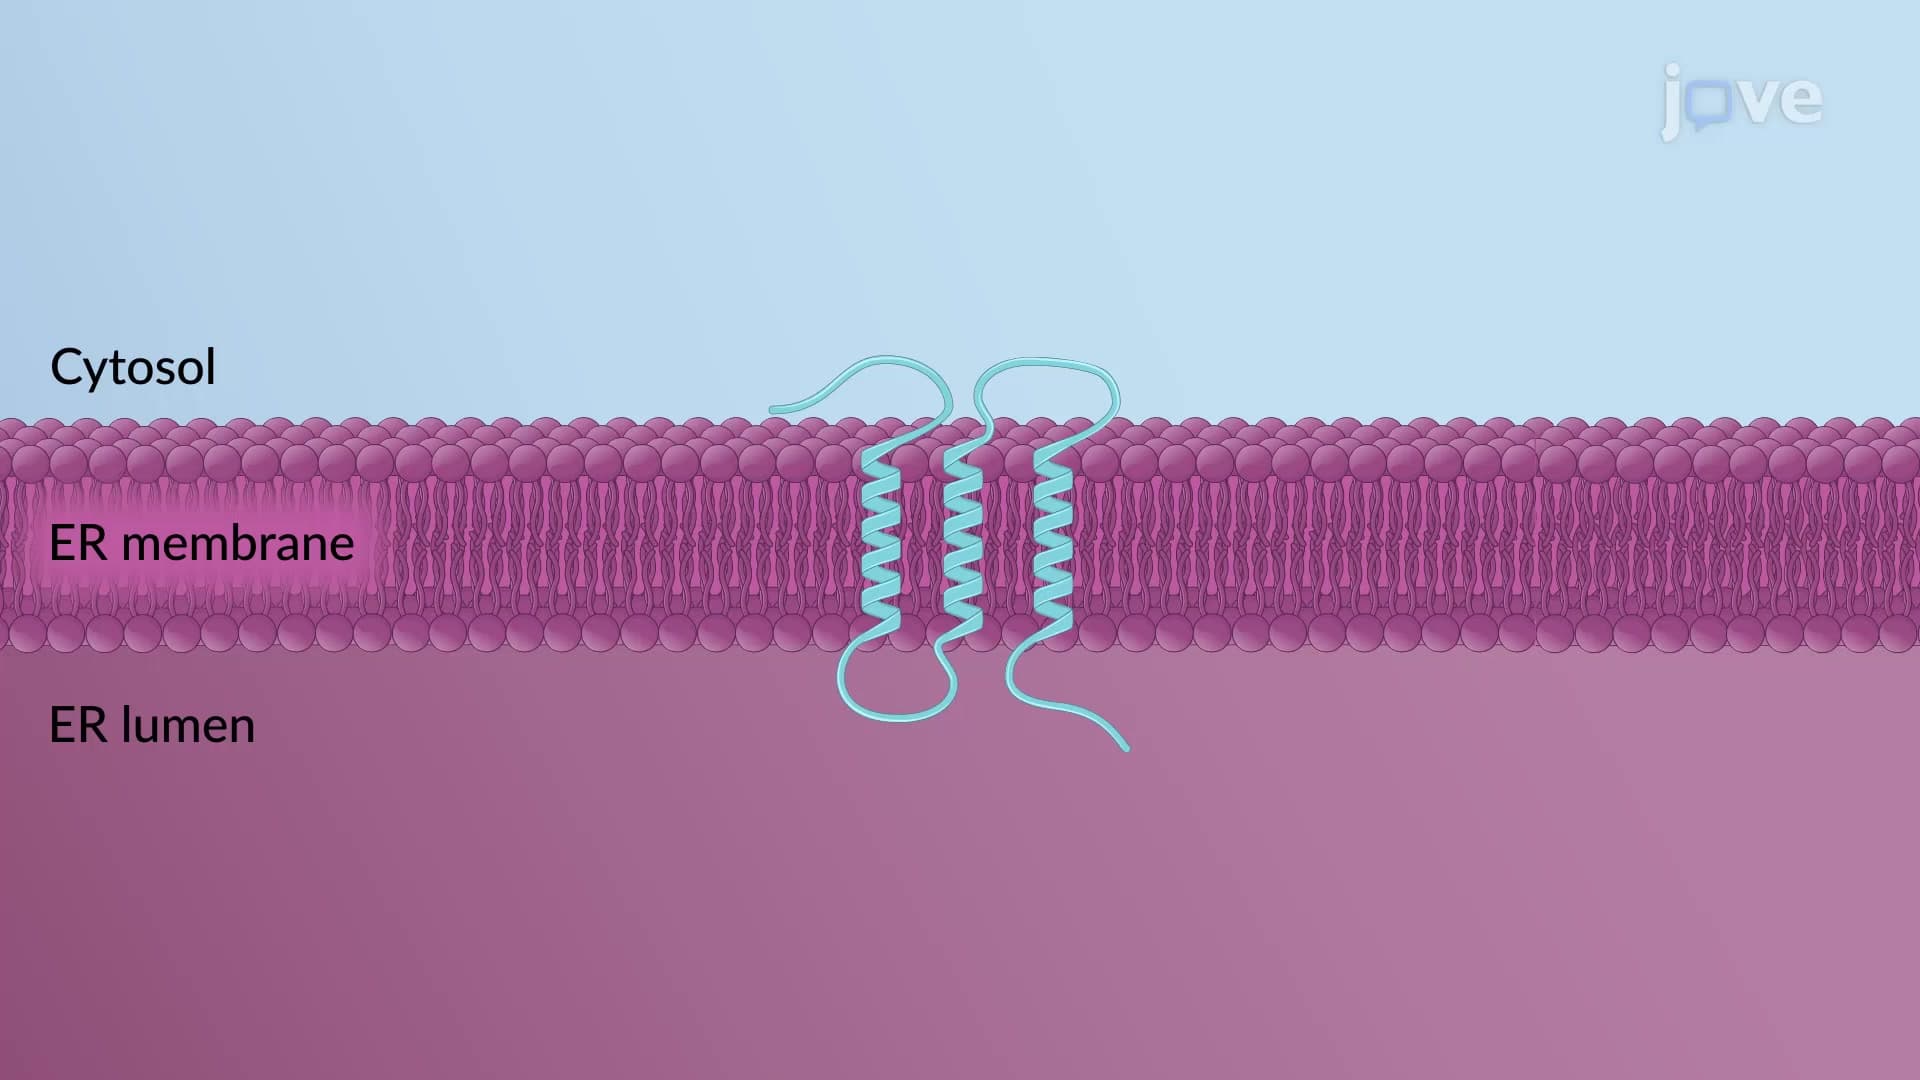
Insertion of Multi-pass Transmembrane Proteins in the RER
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
 01:32
Assembly of Complex Microtubule Structures