Related Experiment Video
Updated: Aug 10, 2026

Determination of Molecular Structures of HIV Envelope Glycoproteins using Cryo-Electron Tomography and Automated Sub-tomogram Averaging
Published on: December 1, 2011
HIV-1 envelope proteins complete their folding into six-helix bundles immediately after fusion pore formation
Ruben M Markosyan1, Fredric S Cohen, Grigory B Melikyan
1Department of Molecular Biophysics and Physiology, Rush Medical College, Chicago, Illinois 60612, USA.

Abstract:
Fusion proteins of many viruses, including HIV-1 envelope protein (Env), fold into six-helix bundle structures. Fusion between individual Env-expressing cells and target cells was studied by fluorescence microscopy, and a temperature jump technique, to determine whether folding of Env into a bundle is complete by the time fusion pores have formed. Lowering temperature to 4 degrees C immediately after a pore opened halted pore growth, which quickly resumed when temperature was raised again. HIV gp41-derived peptides that inhibit bundle formation (C34 or N36) caused the cold-arrested pore to quickly and irreversibly close, demonstrating that bundle formation is not complete by the time a pore has formed. In contrast, lowering the temperature to an intermediate value also halted pore growth, but the pore was not closed by the bundle-inhibiting peptides, and it enlarged when temperature was again elevated. This latter result shows that bundle formation is definitely required for the fusion process, but surprisingly, some (if not all) bundle formation occurs after a pore has formed. It is concluded that an essential function of the bundle is to stabilize the pore against collapse and ensure its growth.
Related Concept Videos
 02:41
Protein Complex Assembly
Many viruses self-assemble into a fully functional unit using the infected host cell to...
 03:00
Molecular Chaperones and Protein Folding
The...
 01:12
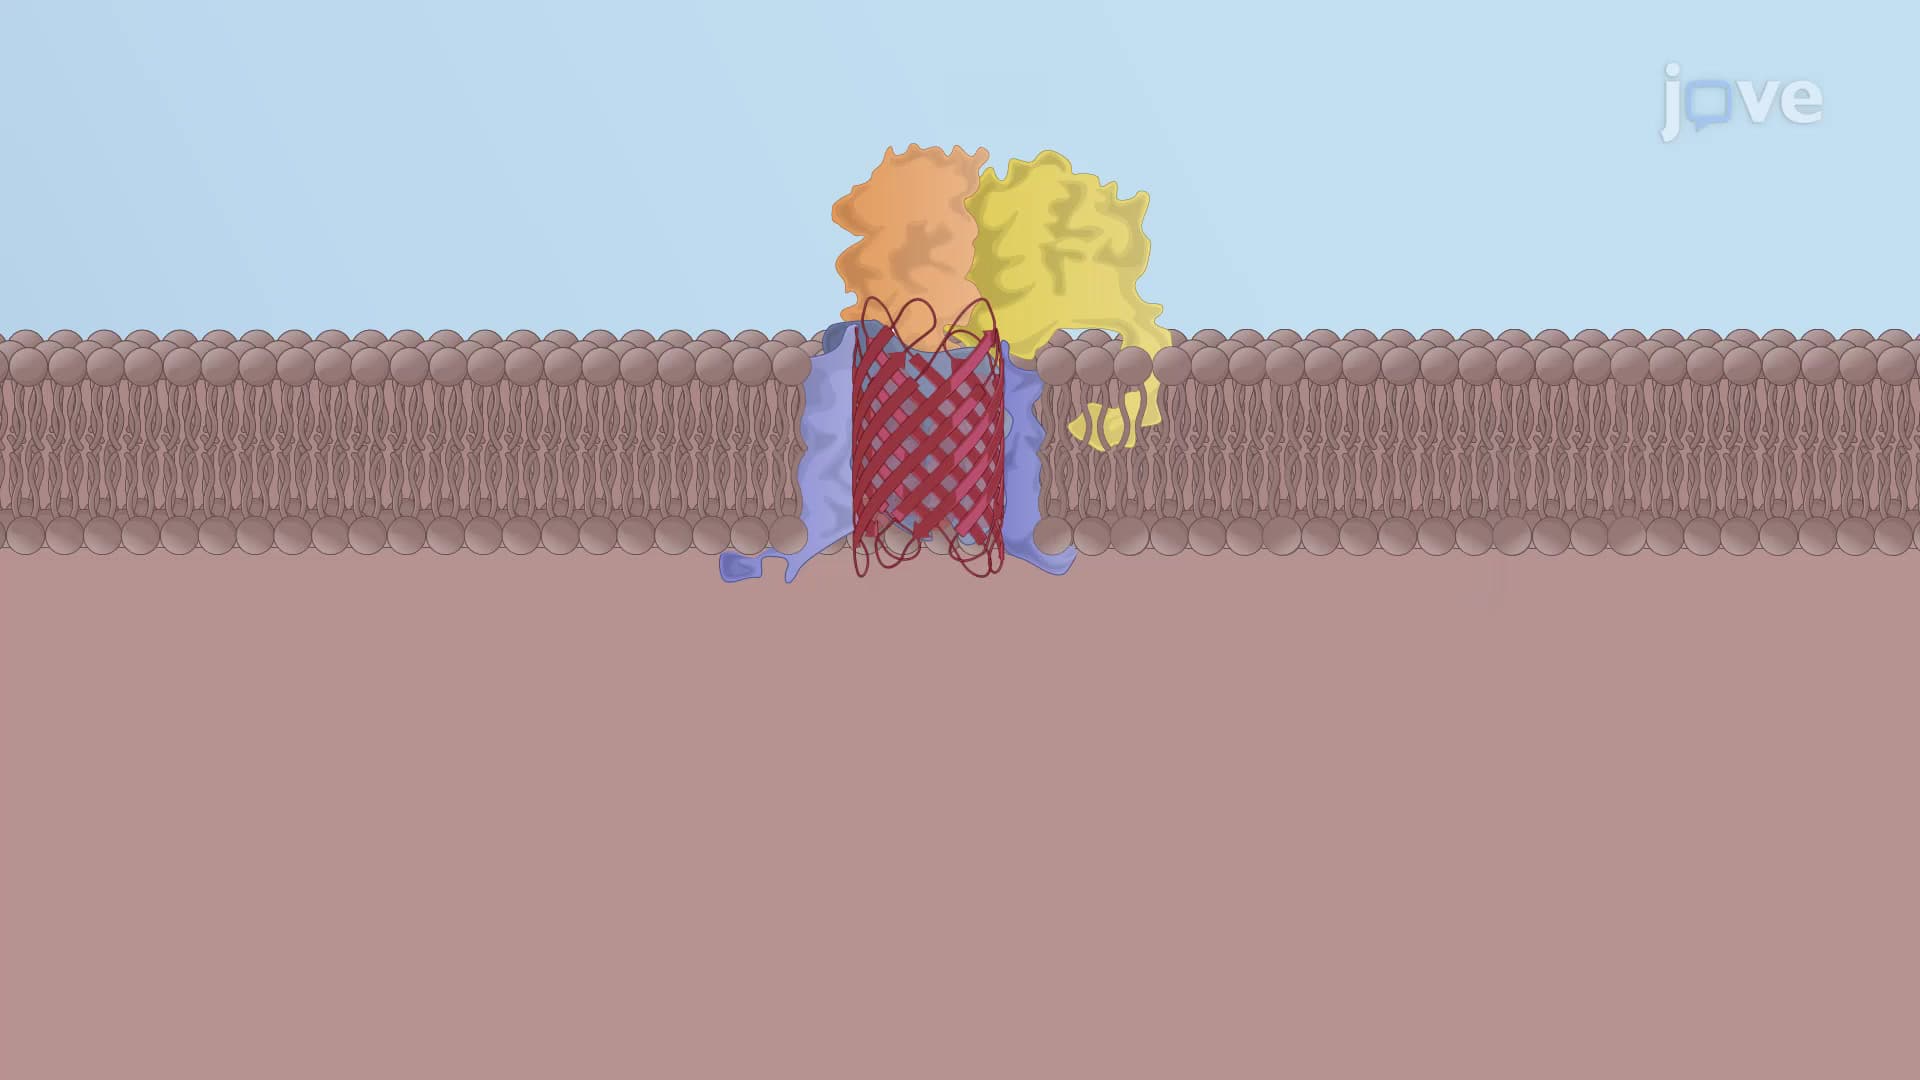
Porin Insertion in the Outer Mitochondrial Membrane
Three models describe the assembly of porins by the SAM complex and their insertion into the outer membrane. Model 1 suggests that porins are assembled outside the SAM channel as the...
 01:43
SNAREs and Membrane Fusion
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 01:45
Vesicular Tubular Clusters
With the help of motor proteins such...
 01:19
Inhibitors of Virion Maturation and Assembly