Related Experiment Video
Updated: Jul 8, 2026
Homogeneous Glycoconjugate Produced by Combined Unnatural Amino Acid Incorporation and Click-Chemistry for Vaccine Purposes
Published on: December 19, 2020
The BTB protein MEL-26 is a substrate-specific adaptor of the CUL-3 ubiquitin-ligase
Lionel Pintard1, John H Willis, Andrew Willems
1Institute of Biochemistry ETH, Hönggerberg 8093, Zürich, Switzerland. lionel.pintard@bc.biol.ethz.ch

Abstract:
Many biological processes, such as development and cell cycle progression are tightly controlled by selective ubiquitin-dependent degradation of key substrates. In this pathway, the E3-ligase recognizes the substrate and targets it for degradation by the 26S proteasome. The SCF (Skp1-Cul1-F-box) and ECS (Elongin C-Cul2-SOCS box) complexes are two well-defined cullin-based E3-ligases. The cullin subunits serve a scaffolding function and interact through their C terminus with the RING-finger-containing protein Hrt1/Roc1/Rbx1, and through their N terminus with Skp1 or Elongin C, respectively. In Caenorhabditis elegans, the ubiquitin-ligase activity of the CUL-3 complex is required for degradation of the microtubule-severing protein MEI-1/katanin at the meiosis-to-mitosis transition. However, the molecular composition of this cullin-based E3-ligase is not known. Here we identified the BTB-containing protein MEL-26 as a component required for degradation of MEI-1 in vivo. Importantly, MEL-26 specifically interacts with CUL-3 and MEI-1 in vivo and in vitro, and displays properties of a substrate-specific adaptor. Our results suggest that BTB-containing proteins may generally function as substrate-specific adaptors in Cul3-based E3-ubiquitin ligases.
Insights
Researchers identified MEL-26 as a key component of the Cul3-based E3-ubiquitin ligase complex. This complex is essential for the degradation of the MEI-1 protein during cell cycle transitions in C. elegans.
Area of Science:
- Molecular Biology
- Cell Biology
- Biochemistry
Background:
- Ubiquitin-dependent degradation controls crucial biological processes like development and cell cycle.
- E3-ligases, including SCF and ECS complexes, mediate substrate targeting for proteasomal degradation.
- The CUL-3 complex's role in MEI-1 degradation during the meiosis-to-mitosis transition in C. elegans is known, but its composition is unclear.
Purpose of the Study:
- To identify the molecular components of the CUL-3 E3-ubiquitin ligase complex responsible for MEI-1 degradation.
- To elucidate the function of BTB-containing proteins in Cul3-based E3-ligase complexes.
Main Methods:
- Yeast two-hybrid screening or co-immunoprecipitation to identify interacting proteins.
- In vivo and in vitro binding assays to confirm interactions between MEL-26, CUL-3, and MEI-1.
- Functional assays in C. elegans to assess the role of MEL-26 in MEI-1 degradation.
Main Results:
- MEL-26 was identified as a necessary component for MEI-1 degradation in vivo.
- MEL-26 directly interacts with both CUL-3 and MEI-1.
- MEL-26 functions as a substrate-specific adaptor within the Cul3-based E3-ubiquitin ligase complex.
Conclusions:
- BTB-containing proteins, exemplified by MEL-26, are likely general substrate-specific adaptors for Cul3-based E3-ubiquitin ligases.
- This finding expands our understanding of the regulation of protein degradation by cullin-based E3-ligases.
- The study provides a molecular basis for the selective degradation of MEI-1 during C. elegans development.
Related Concept Videos
 01:57
Protein Complexes with Interchangeable Parts
The SCF ubiquitin ligase is a protein complex of five individual proteins. This complex attaches ubiquitin to other target proteins to mark them for degradation. In order to...
 01:38
Intralumenal Vesicles and Multivesicular Bodies
 01:19
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
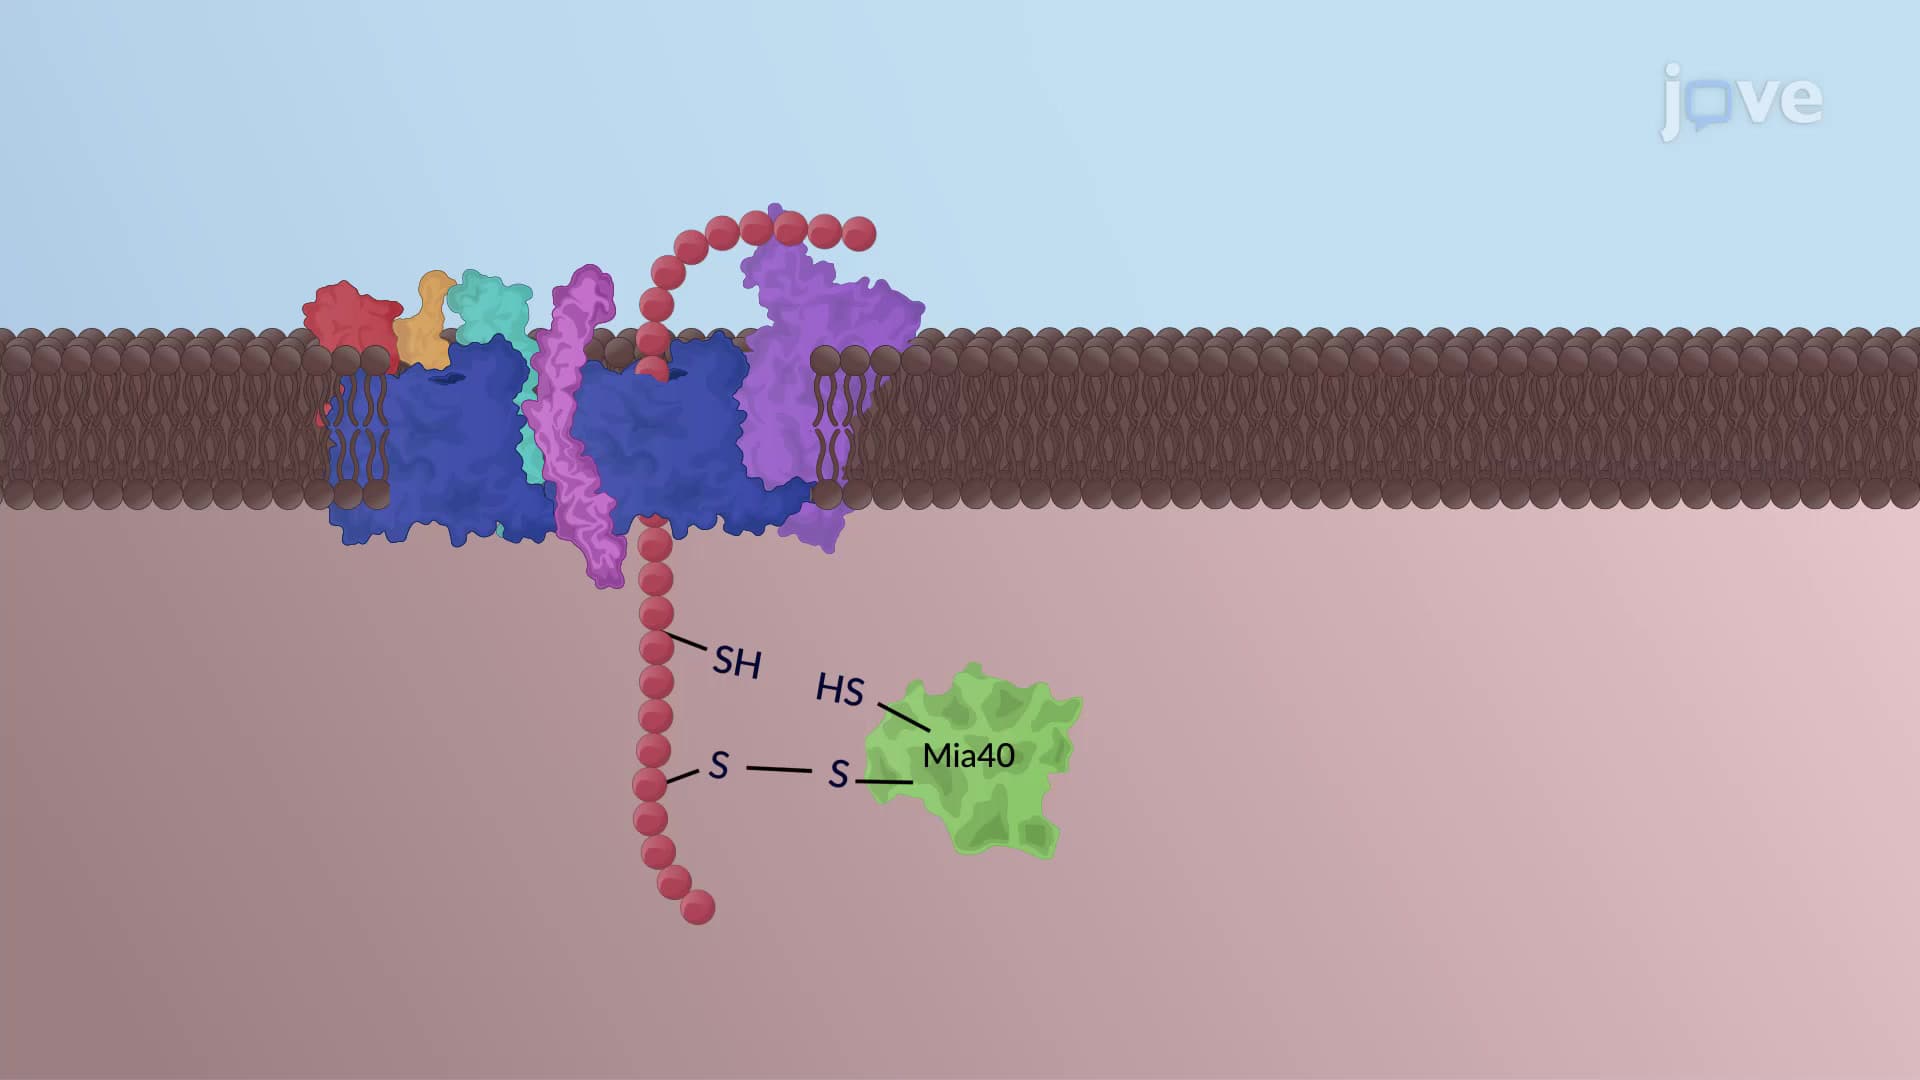
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:34
Protein Transport into the Inner Mitochondrial Membrane
Transport of mitochondrial precursors across the TIM23 channel is driven by...
 01:28
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.
 01:26
Bacterial Translocation and Protein Secretion