
Dimerization kinetics of the IgE-class antibodies by divalent haptens. II. The interactions between intact IgE and
R Schweitzer-Stenner1, A Licht, I Pecht
1Institute of Experimental Physics, University of Bremen, Germany.

Interactions between a monoclonal, DNP-specific IgE molecules (hybridoma A2) and divalent DNP-haptens in solution cause aggregation of the former predominantly into closed rings of two IgE and two divalent haptens (Schweitzer-Stenner, R., A. Licht, I. Lüscher, and I. Pecht. 1987. Biochemistry. 26:3602-3612). The time course of this process was now investigated by titrating the A2-IgE with divalent DNP-haptens having long and rigid oligoproline spacers (di(N epsilon-2,4-dinitrophenyl)-6-amino-hexanoate-aspartyl-(prolyl)n-L-ly- syl; n = 24, 27, 33). Binding was expressed in quenching of the IgE intrinsic tryptophan emission. As shown in the preceding paper, hapten addition to the IgE-A2 at rates faster than a distinct threshold value led to nonequilibrium titrations (NETs) from which kinetic processes slower than 2 s-1 can be resolved. Analysis of these titrations shows that the dimeric rings open at rates of approximately 10(-2) s-1, independent of the divalent hapten's spacer length. The ring closure rate, however, decreases with spacer length. The latter observation was qualitatively rationalized in terms of the diffusion process of a Gaussian chain which relates the ring closure rate constant to the expectation value for the distance between the free ends of the respective open chain.
Interactions between a monoclonal, DNP-specific IgE molecules (hybridoma A2) and divalent DNP-haptens in solution cause aggregation of the former predominantly into closed rings of two IgE and two divalent haptens (Schweitzer-Stenner, R., A. Licht, I. Lüscher, and I. Pecht. 1987. Biochemistry. 26:3602-3612). The time course of this process was now investigated by titrating the A2-IgE with divalent DNP-haptens having long and rigid oligoproline spacers (di(N epsilon-2,4-dinitrophenyl)-6-amino-hexanoate-aspartyl-(prolyl)n-L-ly- syl; n = 24, 27, 33). Binding was expressed in quenching of the IgE intrinsic tryptophan emission. As shown in the preceding paper, hapten addition to the IgE-A2 at rates faster than a distinct threshold value led to nonequilibrium titrations (NETs) from which kinetic processes slower than 2 s-1 can be resolved. Analysis of these titrations shows that the dimeric rings open at rates of approximately 10(-2) s-1, independent of the divalent hapten's spacer length. The ring closure rate, however, decreases with spacer length. The latter observation was qualitatively rationalized in terms of the diffusion process of a Gaussian chain which relates the ring closure rate constant to the expectation value for the distance between the free ends of the respective open chain.
More Related Videos
Related Concept Videos
 01:10
Antibody Structure
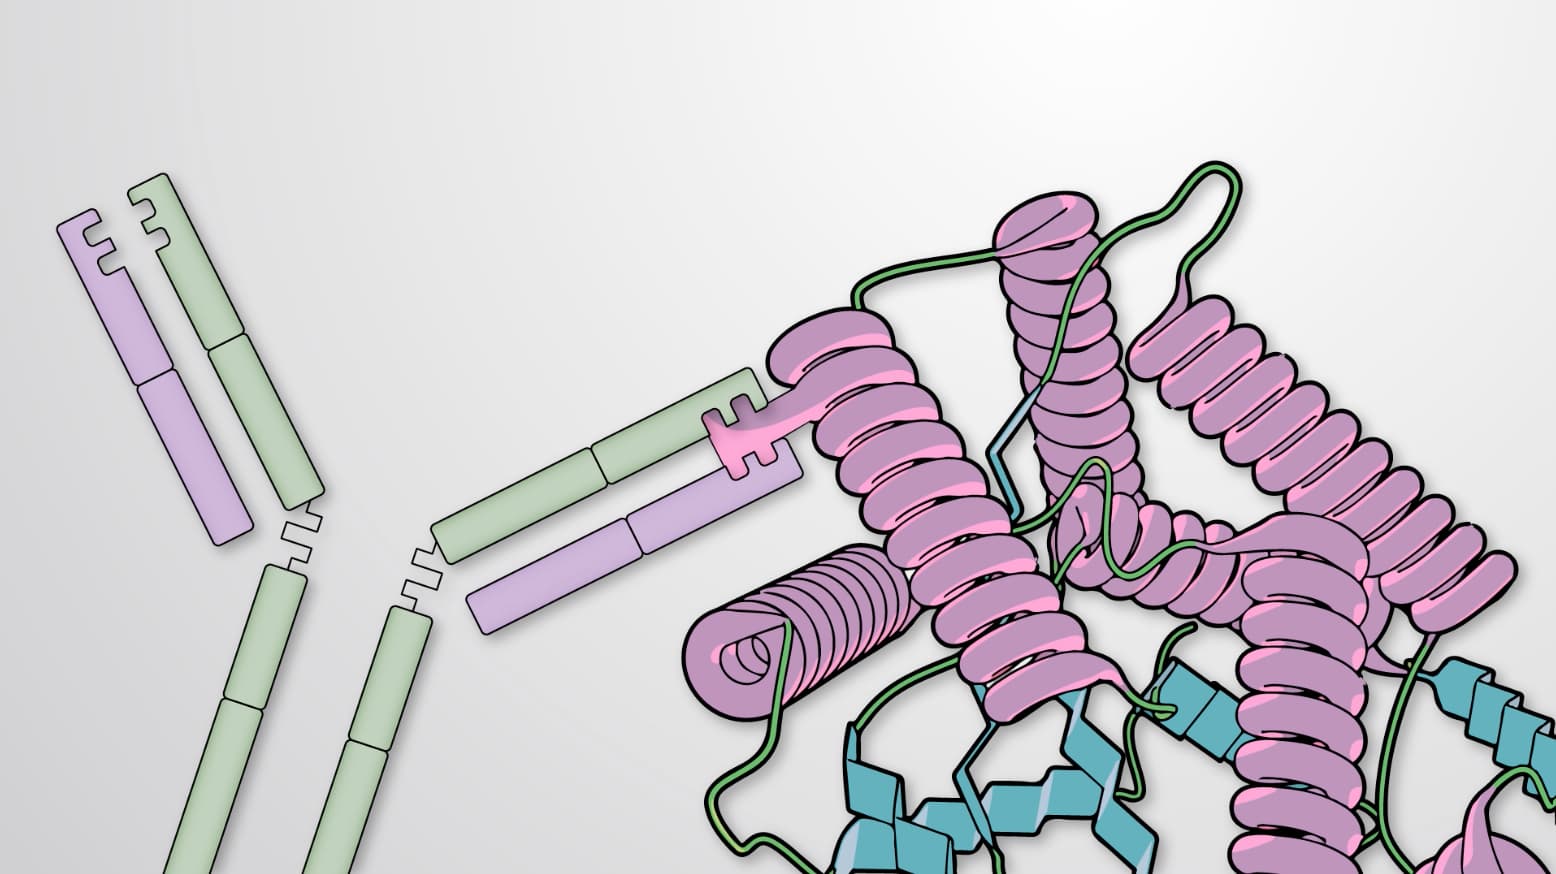
Antibodies, also known as immunoglobulins (Ig), are essential players of the adaptive immune system. These antigen-binding proteins are produced by B cells and make up 20 percent of the total blood plasma by weight. In mammals, antibodies fall into five different classes, which each elicits a different biological response upon antigen binding.
The Y-Shaped Structure of Antibodies Consists of Four Polypeptide Chains
Antibodies consist of four polypeptide chains: two identical heavy...
 01:41
Affinity and Avidity
 01:26
Antigens Involved in Adaptive Immunity
Complete Antigens
Complete antigens possess both immunogenicity and reactivity.
 01:25
Antibody Structure and Classes
The basic structure of an antibody consists of four protein chains: two identical heavy chains and two identical light chains. These chains are held together by disulfide bonds and other non-covalent interactions, forming a Y-shaped structure.
 01:01
Hypersensitivity Reactions: Cytolytic Reactions
 01:19
Hypersensitivity Reactions: Immune-Complex Reactions