Related Experiment Video
Updated: Aug 31, 2026

In Vitro Reconstitution of Self-Organizing Protein Patterns on Supported Lipid Bilayers
Published on: July 28, 2018
Dependence of M13 major coat protein oligomerization and lateral segregation on bilayer composition
Fábio Fernandes1, Luís M S Loura, Manuel Prieto
1Centro de Química-Física Molecular, Instituto Superior Técnico, Lisboa, Portugal.

Abstract:
M13 major coat protein was derivatized with BODIPY (n-(4,4-difluoro-5,7-dimethyl-4-bora-3a,4a-diaza-s-indacene-3-yl)methyl iodoacetamide), and its aggregation was studied in 1,2-dioleoyl-sn-glycero-3-phosphocholine (DOPC) and DOPC/1,2-dioleoyl-sn-glycero-3-[phospho-rac-(1-glycerol)] (DOPG) or 1,2-dioleoyl-sn-glycero-3-phosphoethanolamine (DOPE)/DOPG (model systems of membranes with hydrophobic thickness matching that of the protein) using photophysical methodologies (time-resolved and steady-state self-quenching, absorption, and emission spectra). It was concluded that the protein is essentially monomeric, even in the absence of anionic phospholipids. The protein was also incorporated in pure bilayers of lipids with a strong mismatch with the protein transmembrane length, 1,2-dierucoyl-sn-glycero-3-phosphocholine (DEuPC, longer lipid) and 1,2-dimyristoleoyl-sn-glycero-3-phosphocholine (DMoPC, shorter lipid), and in lipidic mixtures containing DOPC and one of these lipids. The protein was aggregated in the pure vesicles of mismatching lipid but remained essentially monomeric in the mixtures as detected from BODIPY fluorescence emission self-quenching. From fluorescence resonance energy transfer (FRET) measurements (donor-n-(iodoacetyl)aminoethyl-1-sulfonaphthylamine (IAEDANS)-labeled protein; acceptor-BODIPY labeled protein), it was concluded that in the DEuPC/DOPC and DMoPC/DOPC lipid mixtures, domains enriched in the protein and the matching lipid (DOPC) are formed.
Related Concept Videos
 01:33
Coat Assembly and GTPases
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
 01:19
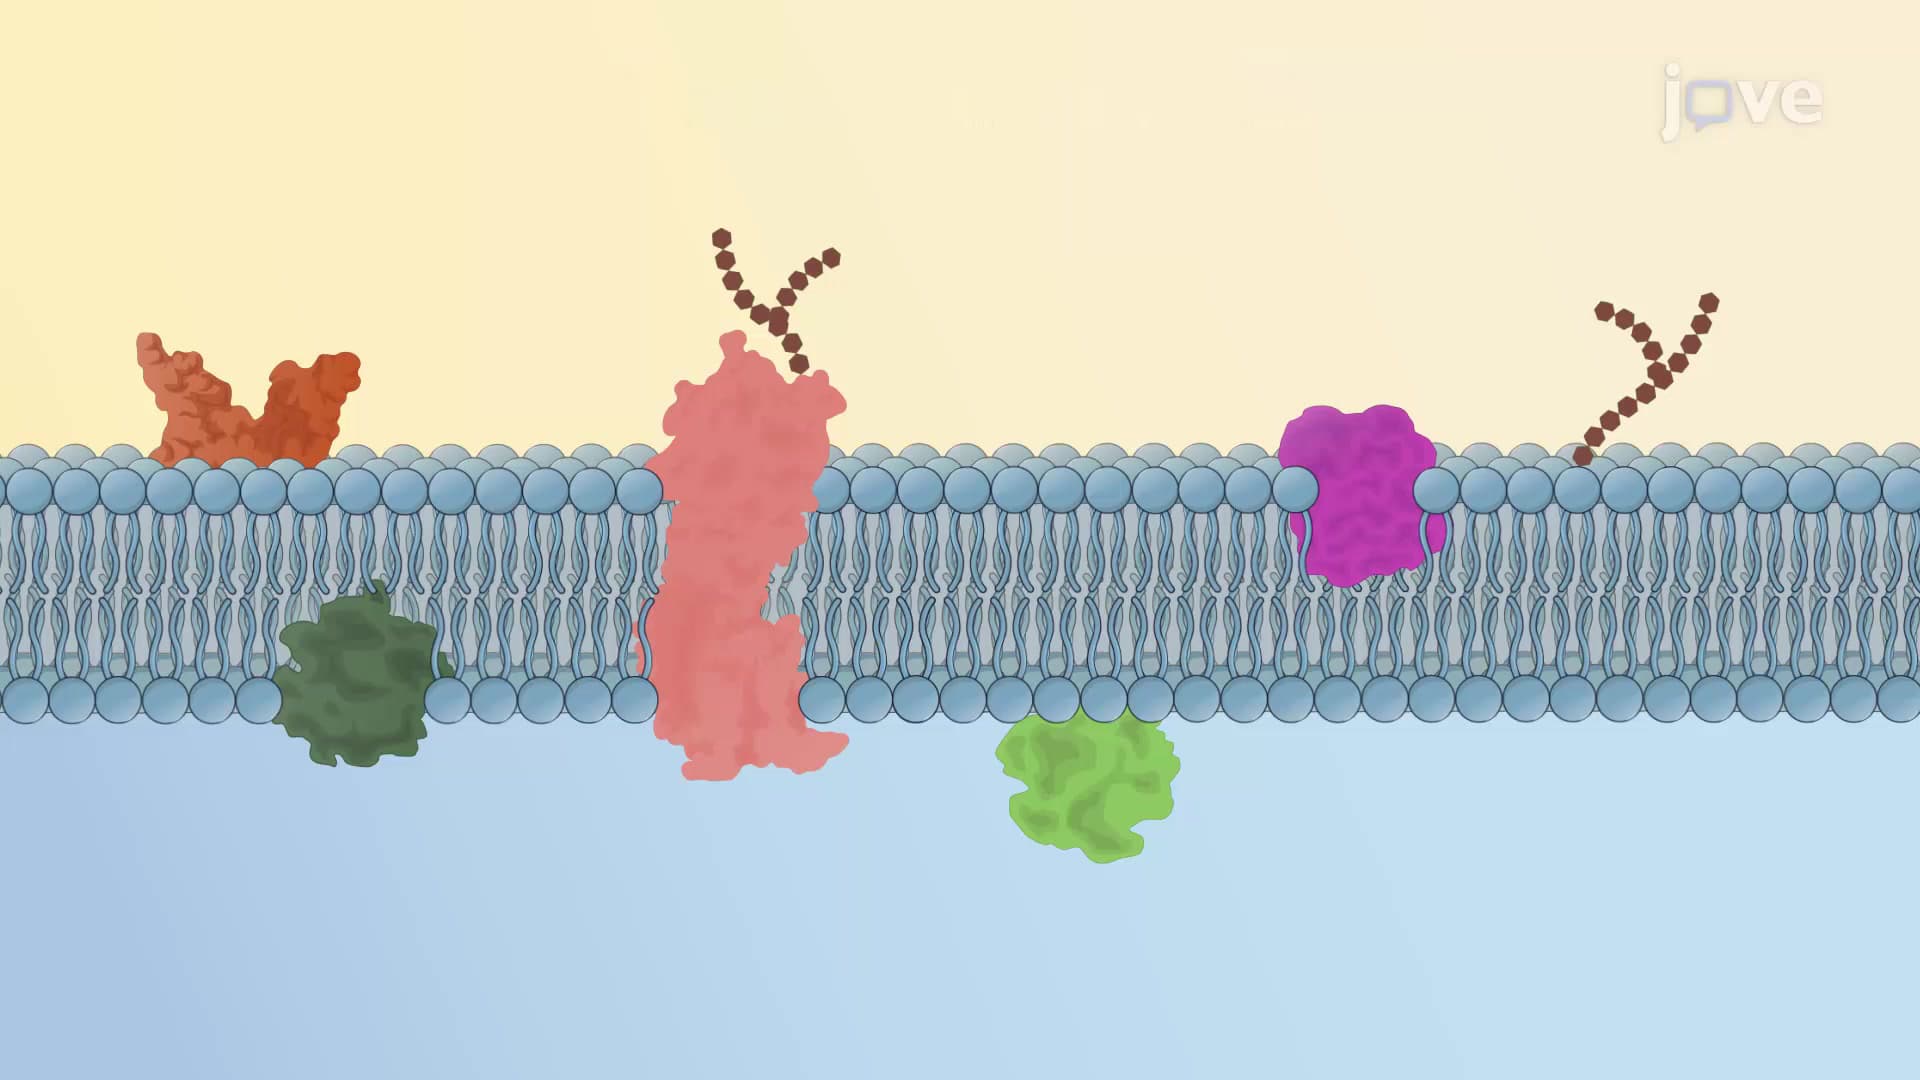
Fluid Mosaic Model
 01:49
Protein Folding
 01:35
Asymmetric Lipid Bilayer
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...
 01:32
Pinching-off of Coated Vesicles