Related Experiment Video
Updated: Aug 29, 2026

Peptide-based Identification of Functional Motifs and their Binding Partners
Published on: June 30, 2013
Small peptides patterned after the N-terminus domain of SNAP25 inhibit SNARE complex assembly and regulated
Clara Blanes-Mira1, Jaime M Merino, Elvira Valera
1Instituto de Biología Molecular y Celular, Universidad Miguel Hernández, Alicante, Spain.

Abstract:
Synthetic peptides patterned after the C-terminus of synaptosomal associated protein of 25 kDa (SNAP25) efficiently abrogate regulated exocytosis. In contrast, the use of SNAP25 N-terminal-derived peptides to modulate SNAP receptors (SNARE) complex assembly and neurosecretion has not been explored. Here, we show that the N-terminus of SNAP25, specially the segment that encompasses 22Ala-44Ile, is essential for the formation of the SNARE complex. Peptides patterned after this protein domain are potent inhibitors of SNARE complex formation. The inhibitory activity correlated with their propensity to adopt an alpha-helical secondary structure. These peptides abrogated SNARE complex formation only when added previous to the onset of aggregate assembly. Analysis of the mechanism of action revealed that these peptides disrupted the binary complex formed by SNAP25 and syntaxin. The identified peptides inhibited Ca2+-dependent exocytosis from detergent-permeabilized excitable cells. Noteworthy, these amino acid sequences markedly protected intact hippocampal neurones against hypoglycaemia-induced, glutamate-mediated excitotoxicity with a potency that rivalled that displayed by botulinum neurotoxins. Our findings indicate that peptides patterned after the N-terminus of SNAP25 are potent inhibitors of SNARE complex formation and neuronal exocytosis. Because of their activity in intact neurones, these cell permeable peptides may be hits for antispasmodic and analgesic drug development.
More Related Videos
Related Concept Videos
 01:43
SNAREs and Membrane Fusion
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
 01:19
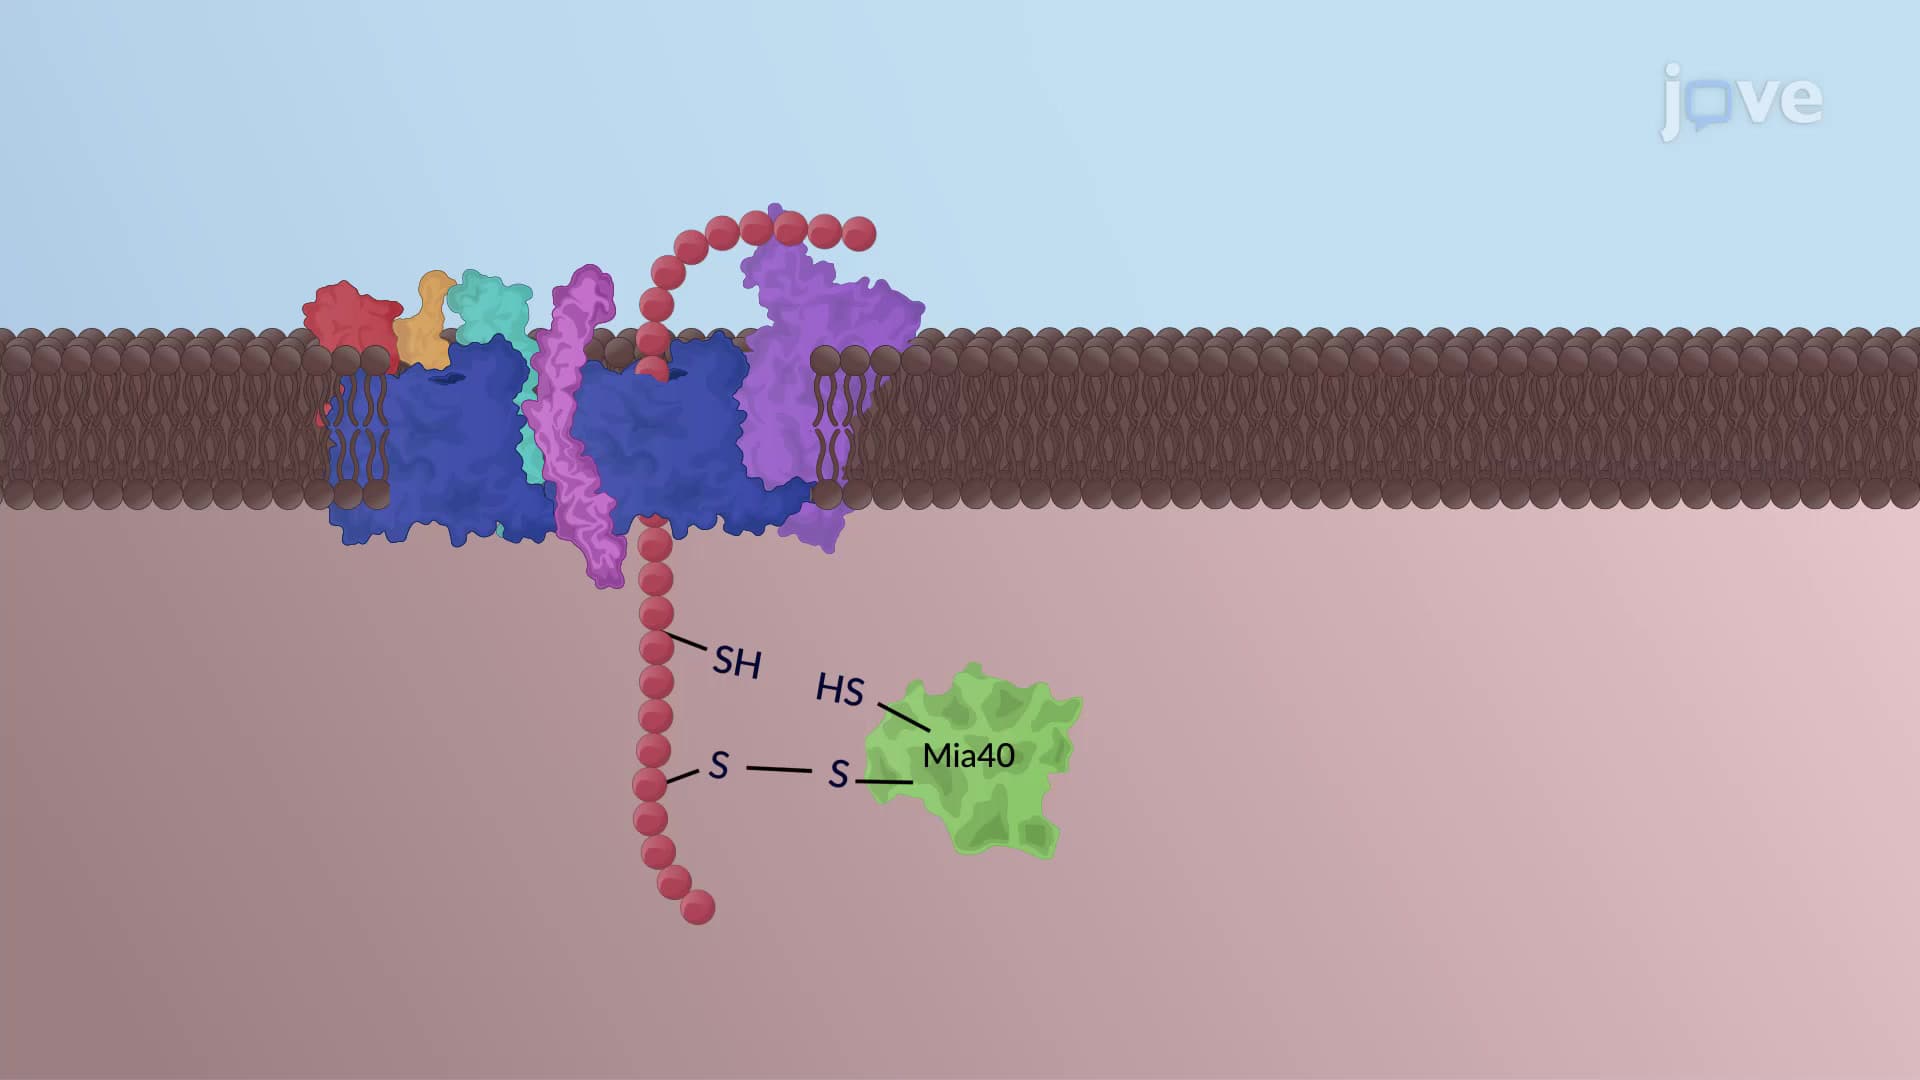
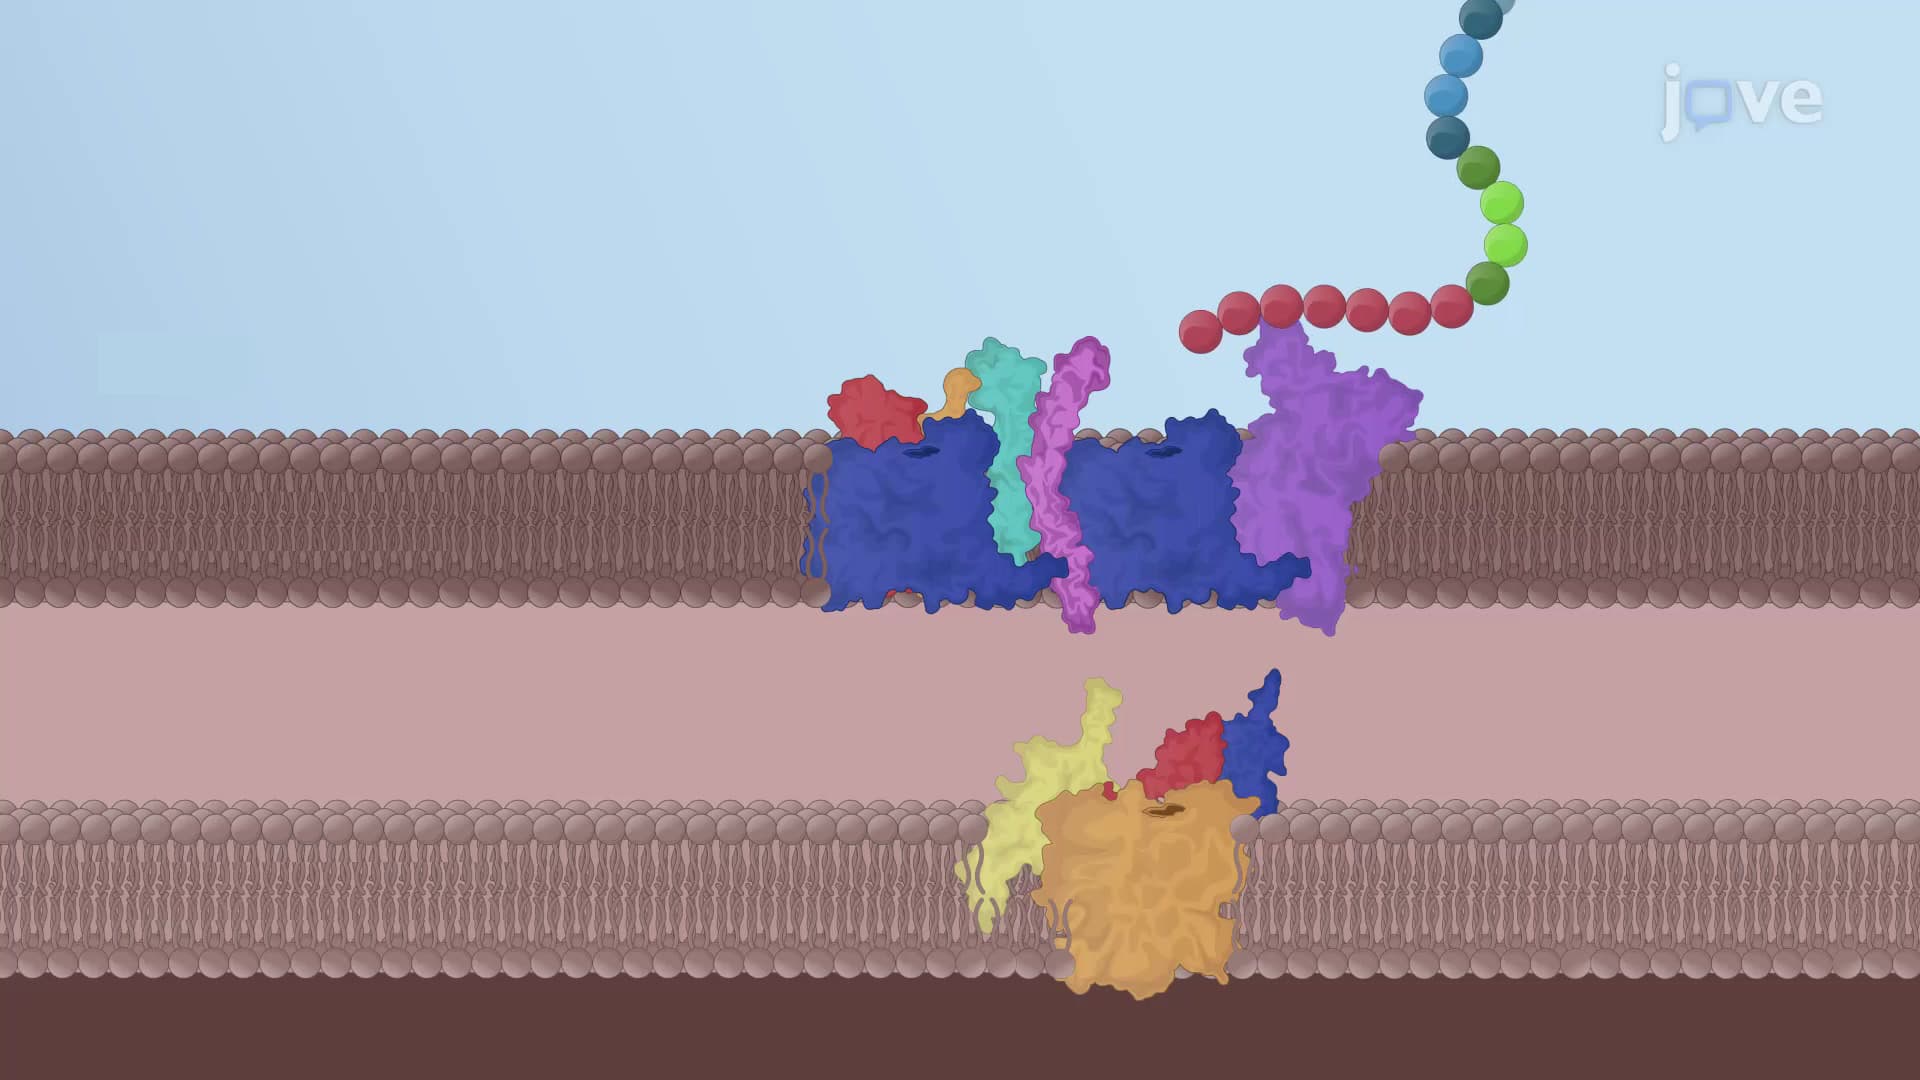
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:32
Pinching-off of Coated Vesicles
 01:39
Mitochondrial Precursor Proteins
Most of the mitochondrial precursors...
 01:45
Regulation of Nuclear Protein Sorting