Related Experiment Video
Updated: Aug 24, 2026

In-vitro Reconstitution of Bacterial Ubiquitination and VCP/p97-mediated Elimination
Published on: January 2, 2026
Ent5p is required with Ent3p and Vps27p for ubiquitin-dependent protein sorting into the multivesicular body
Anne Eugster1, Eve-Isabelle Pécheur, Fabrice Michel
1Laboratoire de Transport et Compartimentation Intracellulaire, Institut de Biologie et Chimie des Protéines, UMR5086 Centre National de la Recherche Scientifique, Institut Fédératif de Recherche 128 BioSciences Lyon-Gerland, 69367 Lyon, France.

Abstract:
At the late endosomes, cargoes destined for the interior of the vacuole are sorted into invaginating vesicles of the multivesicular body. Both PtdIns(3,5)P(2) and ubiquitin are necessary for proper sorting of some of these cargoes. We show that Ent5p, a yeast protein of the epsin family homologous to Ent3p, localizes to endosomes and specifically binds to PtdIns(3,5)P(2) via its ENTH domain. In cells lacking Ent3p and Ent5p, ubiquitin-dependent sorting of biosynthetic and endocytic cargo into the multivesicular body is disrupted, whereas other trafficking routes to the vacuole are not affected. Ent3p and Ent5p are associated with Vps27p, a FYVE domain containing protein that interacts with ubiquitinated cargoes and is required for protein sorting into the multivesicular body. Therefore, Ent3p and Ent5p are the first proteins shown to be connectors between PtdIns(3,5)P(2)- and the Vps27p-ubiquitin-driven sorting machinery at the multivesicular body.
Related Concept Videos
 01:38
Intralumenal Vesicles and Multivesicular Bodies
 01:45
Tail-anchoring of Proteins in the ER Membrane
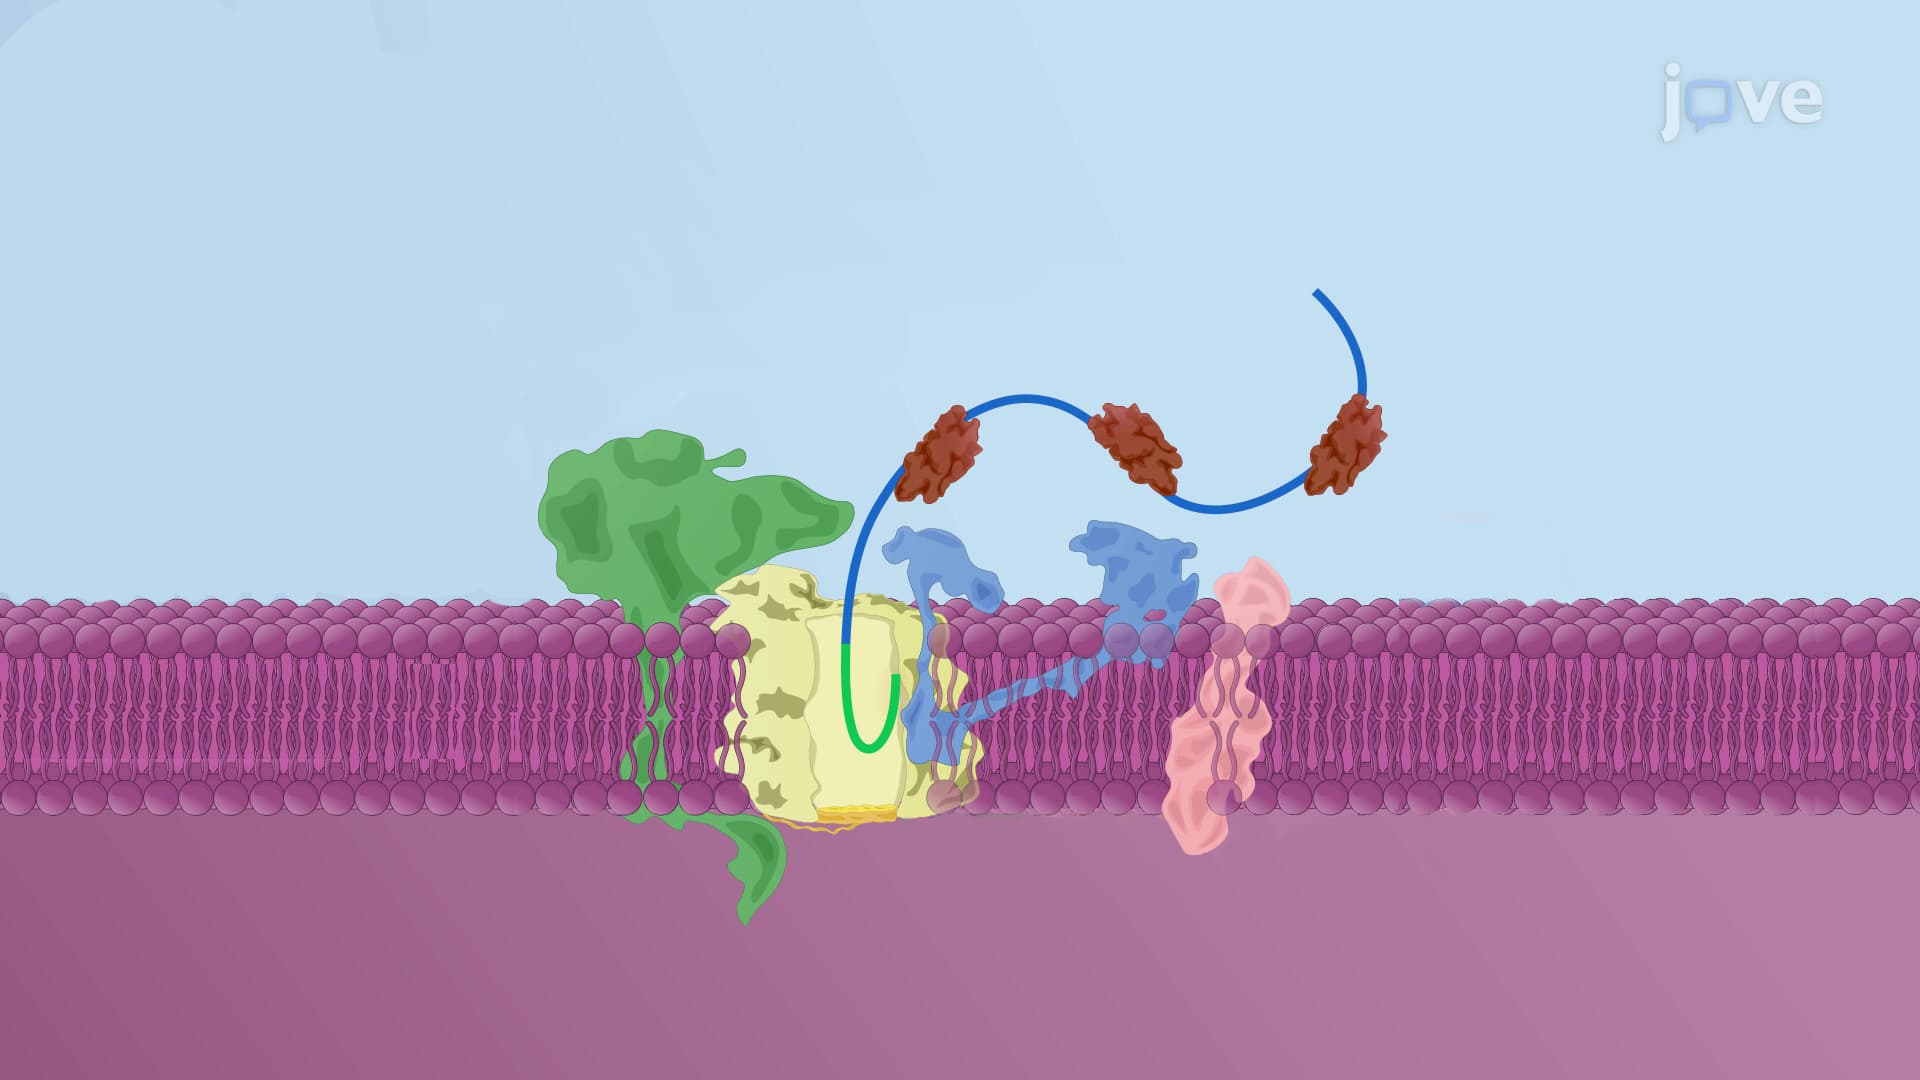 01:27
Post-translational Translocation of Proteins to the RER
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
 01:45
Vesicular Tubular Clusters
With the help of motor proteins such...
 01:37
The Unfolded Protein Response
 01:33
Coat Assembly and GTPases
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...