Related Experiment Video
Updated: Aug 24, 2026
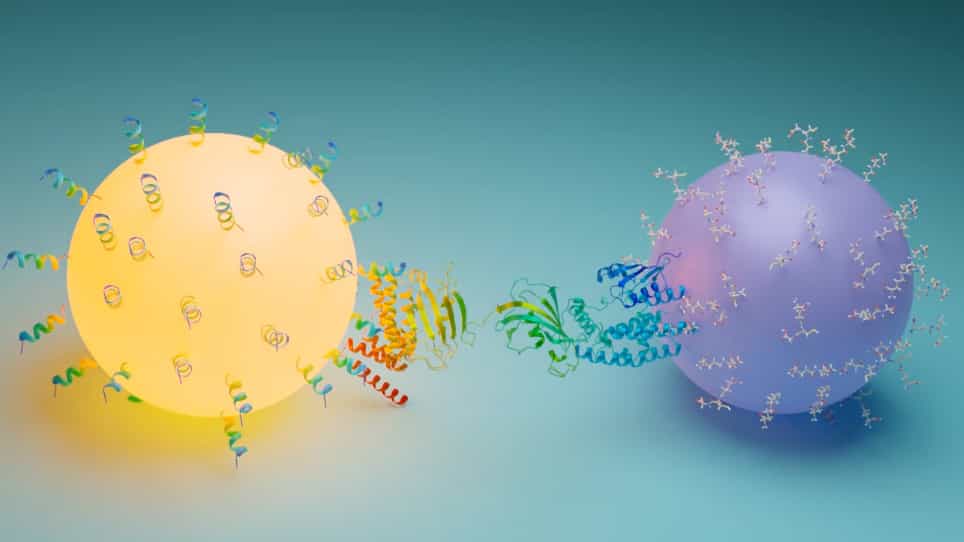
Studies of Chaperone-Cochaperone Interactions using Homogenous Bead-Based Assay
Published on: July 21, 2021
Role of hsp90 and the hsp90-binding immunophilins in signalling protein movement
William B Pratt1, Mario D Galigniana, Jennifer M Harrell
1Department of Pharmacology, University of Michigan Medical School, 1301 Med. Sci. Res. Building III, Ann Arbor, MI 48109-0632, USA. mgali@umich.edu

Abstract:
The ubiquitous protein chaperone hsp90 has been shown to regulate more than 100 proteins involved in cellular signalling. These proteins are called 'client proteins' for hsp90, and a multiprotein hsp90/hsp70-based chaperone machinery forms client protein.hsp90 heterocomplexes in the cytoplasm and the nucleus. In the case of signalling proteins that act as transcription factors, the client protein.hsp90 complexes also contain one of several TPR domain immunophilins or immunophilin homologs that bind to a TPR domain binding site on hsp90. Using several intracellular receptors and the tumor suppressor p53 as examples, we review evidence that dynamic assembly of heterocomplexes with hsp90 is required for rapid movement through the cytoplasm to the nucleus along microtubular tracks. The role of the immunophilin in this system is to connect the client protein.hsp90 complex to cytoplasmic dynein, the motor protein for retrograde movement toward the nucleus. Upon arrival at the nuclear pores, the receptor.hsp90.immunophilin complexes are transferred to the nuclear interior by importin-dependent facilitated diffusion. The unliganded receptors then distribute within the nucleus to diffuse patches from which they proceed in a ligand-dependent manner to discrete nuclear foci where chromatin binding occurs. We review evidence that dynamic assembly of heterocomplexes with hsp90 is required for movement to these foci and for the dynamic exchange of transcription factors between chromatin and the nucleoplasm.
More Related Videos
Related Concept Videos
 03:00
Molecular Chaperones and Protein Folding
The...
 01:30
Assembly of Signaling Complexes
Interaction domains in cell signaling
Interaction domains recognize exposed features of their binding partners containing post-translationally modified sequences,...
 01:27
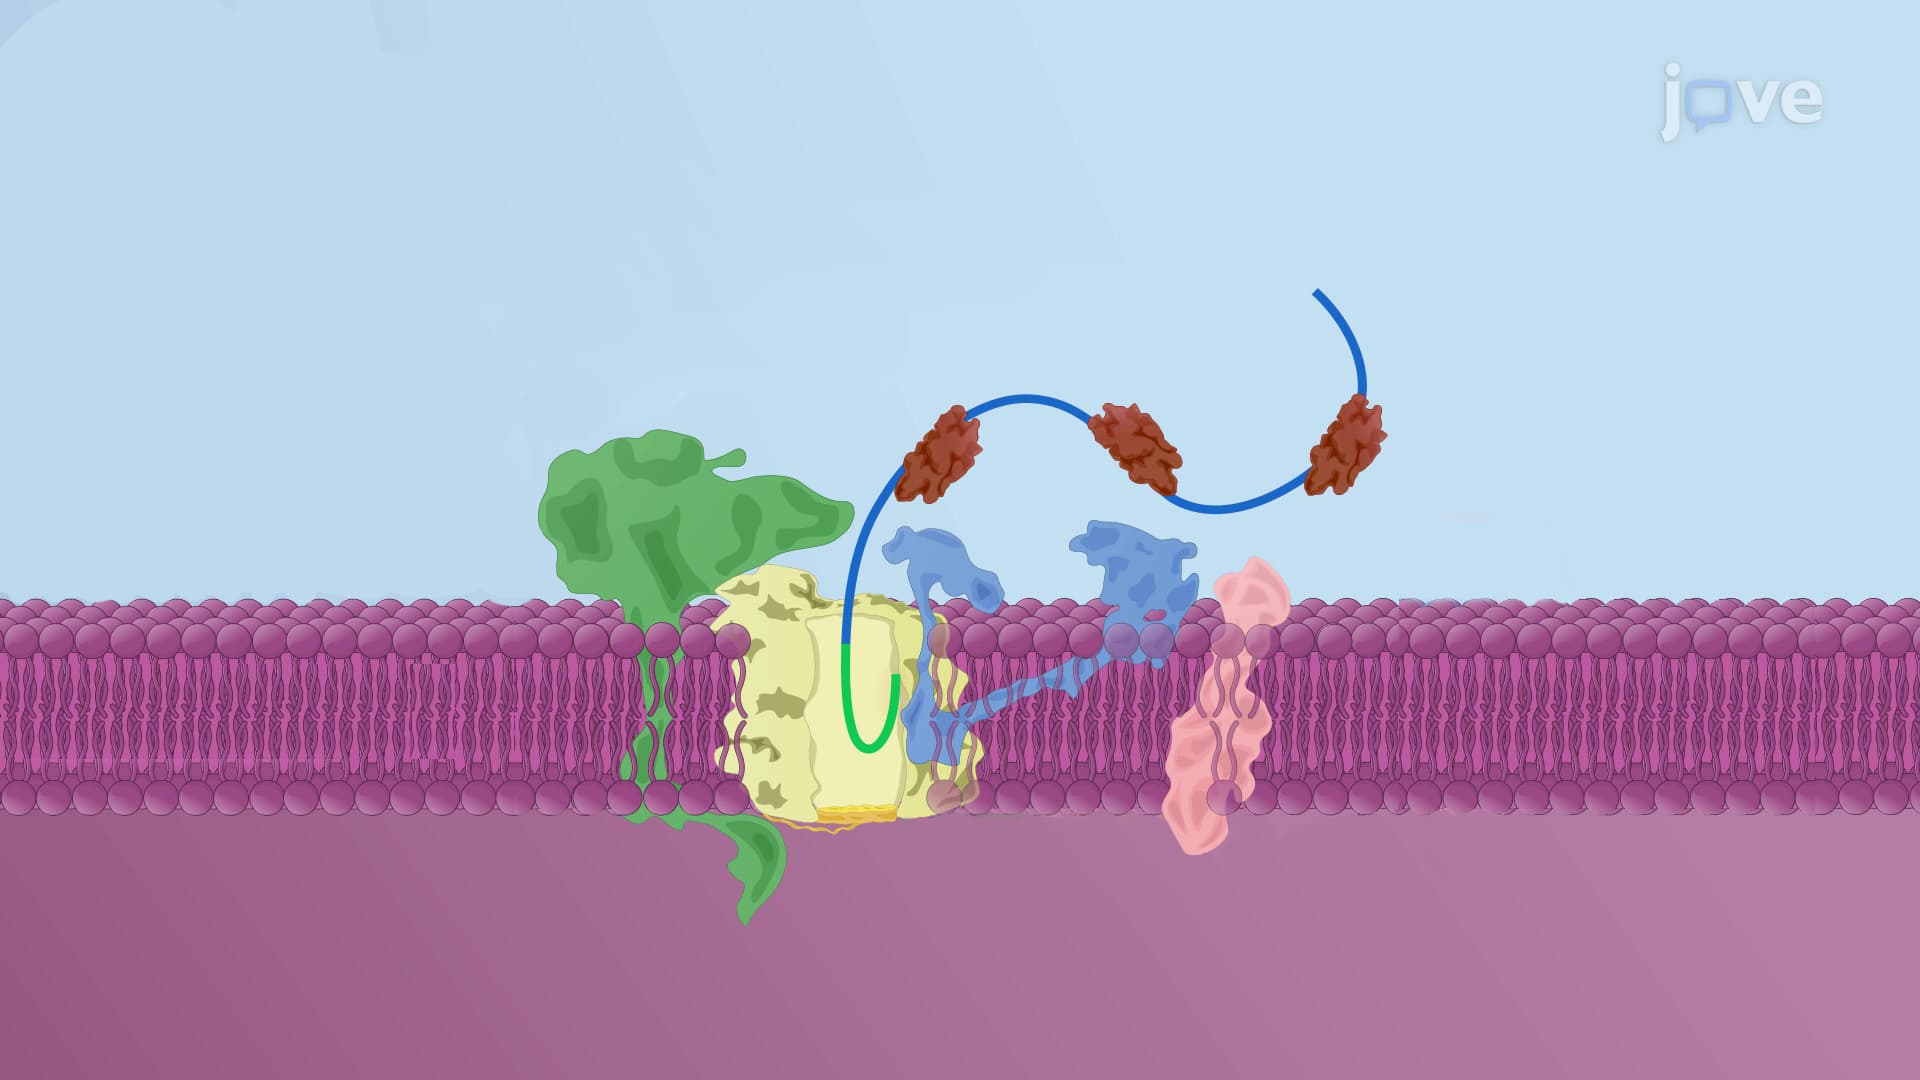
Post-translational Translocation of Proteins to the RER
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
 01:37
Energy to Drive Translocation
Generally, polypeptides are unfolded by two distinct...
 01:19
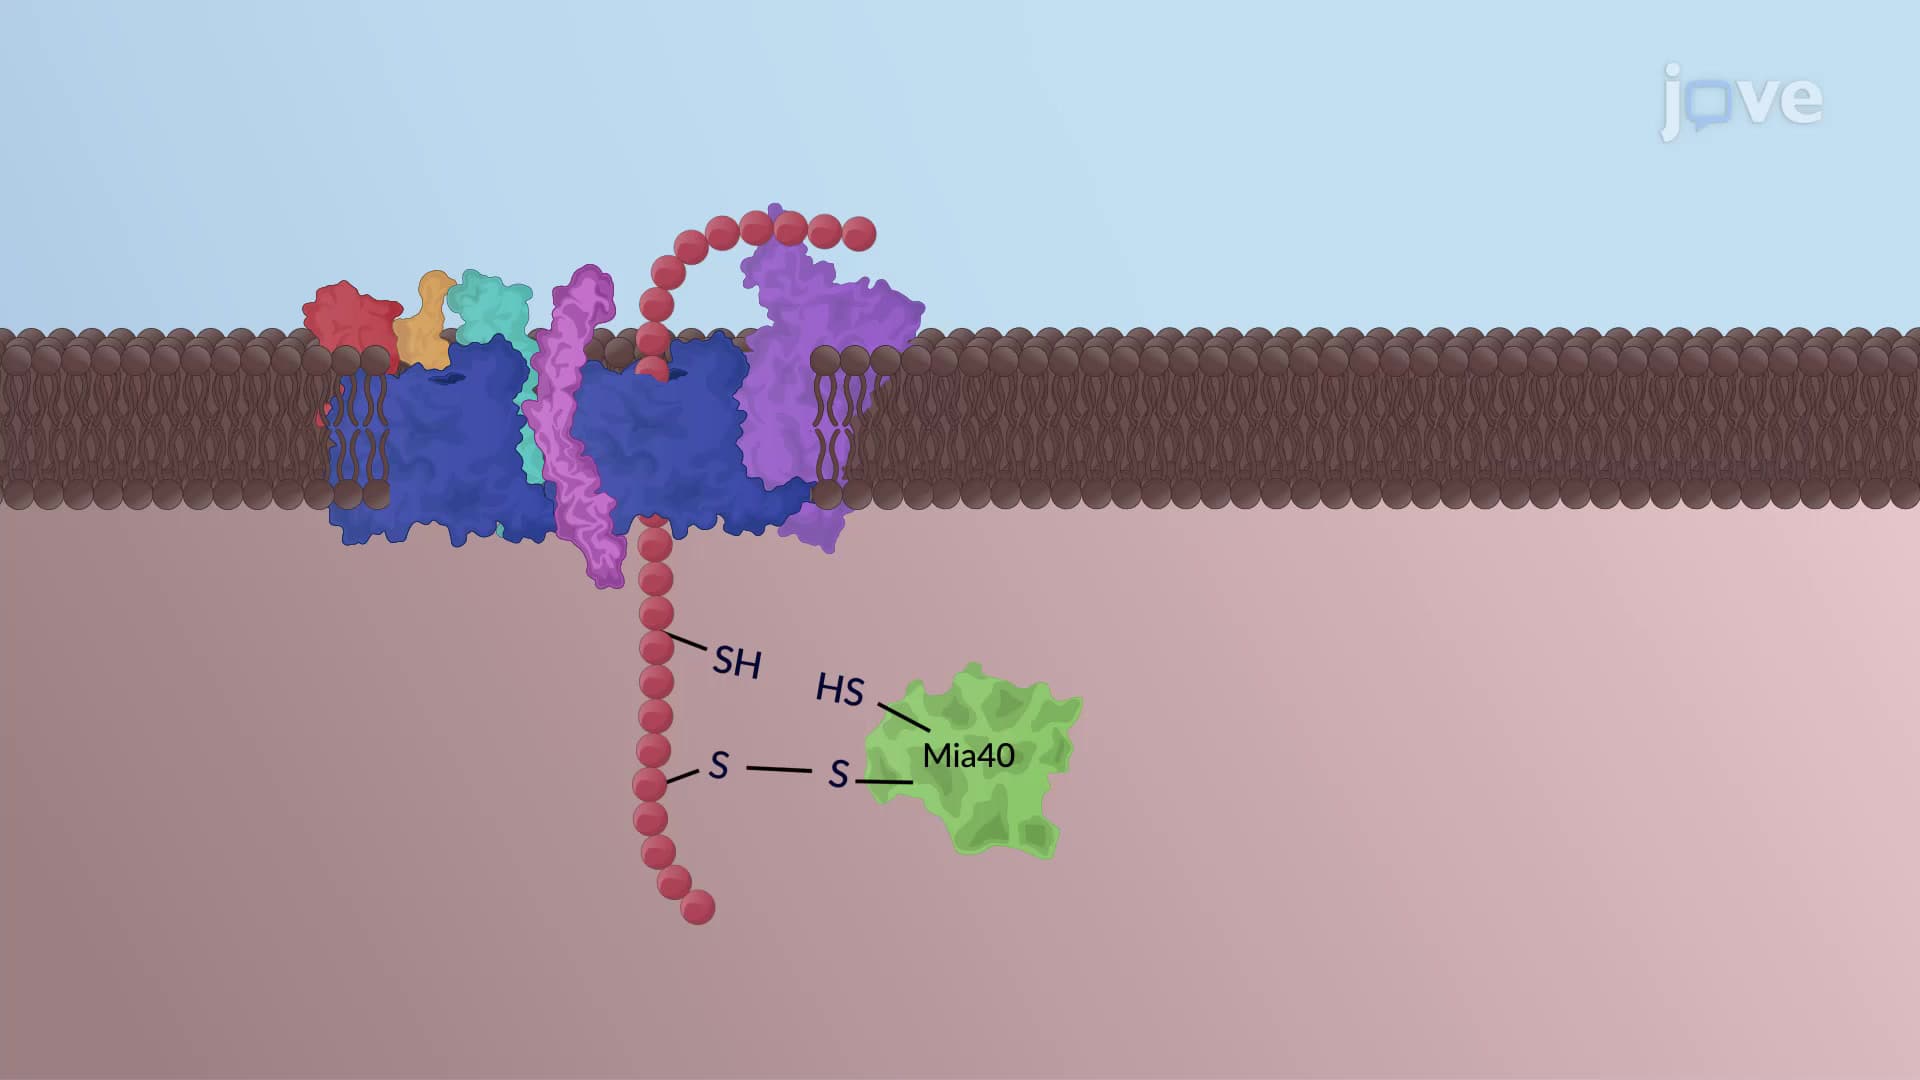
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum