Related Experiment Video
Updated: Aug 20, 2026

Method to Visualize and Analyze Membrane Interacting Proteins by Transmission Electron Microscopy
Published on: March 5, 2017
Lipid-mediated, reversible misfolding of a sterol-sensing domain protein
Alexander G Shearer1, Randolph Y Hampton
1Department of Biology, UCSD Division of Biological Sciences, Section of Cell and Molecular Biology, La Jolla, CA 92093, USA.

Abstract:
Cellular quality control requires recognition of common features of misfolding, and so is not typically associated with the specific targeting of individual proteins. However, physiologically regulated degradation of yeast HMG-CoA reductase (Hmg2p) occurs by the HRD endoplasmic reticulum quality control pathway, implying that Hmg2p undergoes a regulated transition to a quality control substrate in response to a sterol pathway molecule. Using in vitro structural assays, we now show that the pathway derivative farnesol causes Hmg2p to undergo a change to a less folded structure. The effect is reversible, biologically relevant by numerous criteria, highly specific for farnesol structure, and requires an intact Hmg2p sterol-sensing domain. This represents a distinct lipid-sensing function for this highly conserved motif that suggests novel approaches to cholesterol management. More generally, our observation of reversible small-molecule-mediated misfolding may herald numerous examples of regulated quality control to be discovered in biology or applied in the clinic.
Insights
Farnesol, a sterol pathway molecule, reversibly alters yeast HMG-CoA reductase (Hmg2p) structure, marking it for cellular quality control. This discovery suggests new strategies for cholesterol management and reveals a novel mechanism of regulated protein misfolding.
Area of Science:
- Biochemistry
- Cellular Biology
- Molecular Medicine
Background:
- Cellular quality control typically identifies common misfolding patterns, not individual proteins.
- Regulated degradation of yeast HMG-CoA reductase (Hmg2p) involves the HRD endoplasmic reticulum quality control pathway.
- This suggests Hmg2p transitions to a quality control substrate due to a sterol pathway molecule.
Purpose of the Study:
- To investigate the mechanism by which Hmg2p becomes a substrate for regulated degradation.
- To determine if specific sterol pathway molecules can induce structural changes in Hmg2p.
- To explore the implications for cellular quality control and potential therapeutic applications.
Main Methods:
- In vitro structural assays were employed to assess changes in Hmg2p structure.
- The effect of farnesol on Hmg2p folding was analyzed.
- The role of the Hmg2p sterol-sensing domain in this process was investigated.
Main Results:
- Farnesol was shown to induce a reversible change in Hmg2p structure, leading to a less folded state.
- This effect was specific to the farnesol structure and dependent on an intact Hmg2p sterol-sensing domain.
- The observed misfolding was biologically relevant and occurred under physiological conditions.
Conclusions:
- Hmg2p exhibits a novel lipid-sensing function mediated by its sterol-sensing domain.
- Reversible small-molecule-induced misfolding represents a newly identified mechanism of regulated cellular quality control.
- This finding opens new avenues for cholesterol management and therapeutic interventions.
Related Concept Videos
 01:32
Export of Misfolded Proteins out of the ER
 01:31
Regulation of the Unfolded Protein Response
 01:37
The Unfolded Protein Response
 01:45
Regulation of Nuclear Protein Sorting
 03:00
Molecular Chaperones and Protein Folding
The...
 01:26
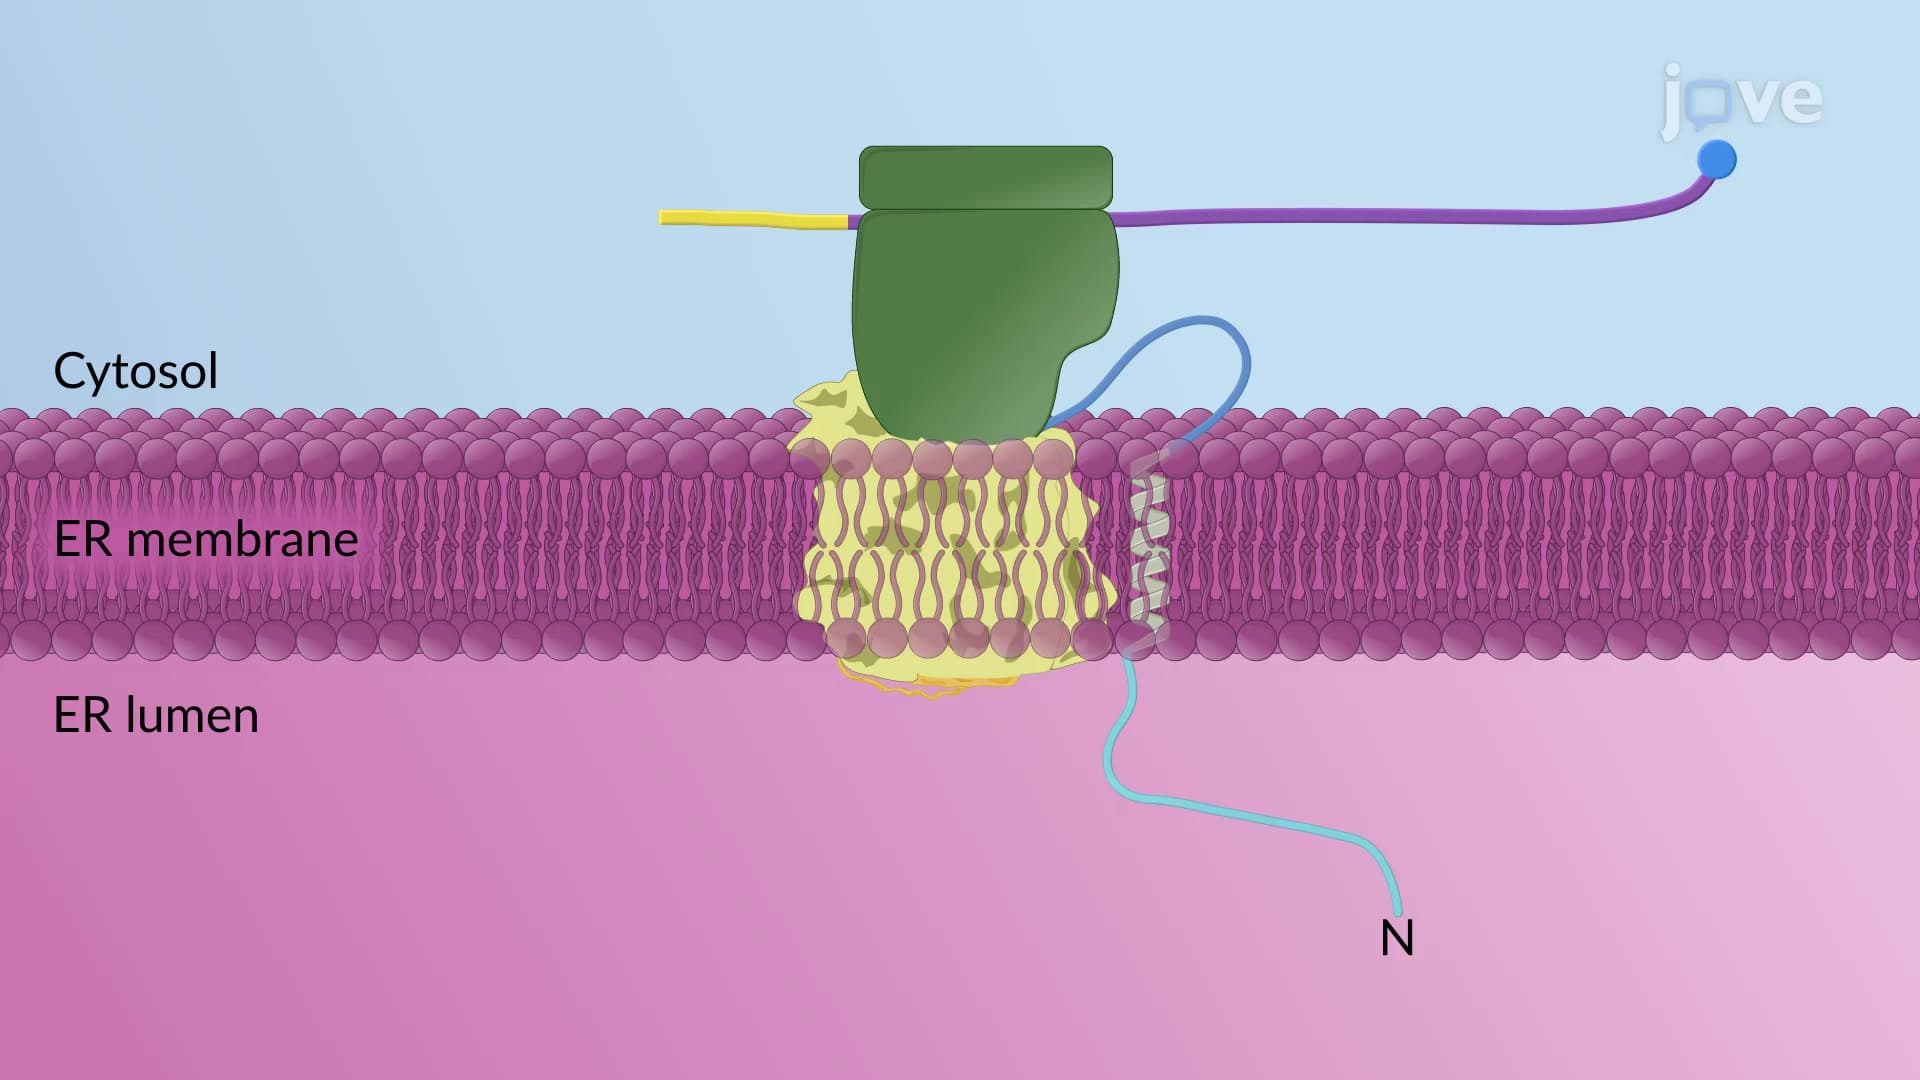
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...