Related Experiment Video
Updated: Aug 19, 2026
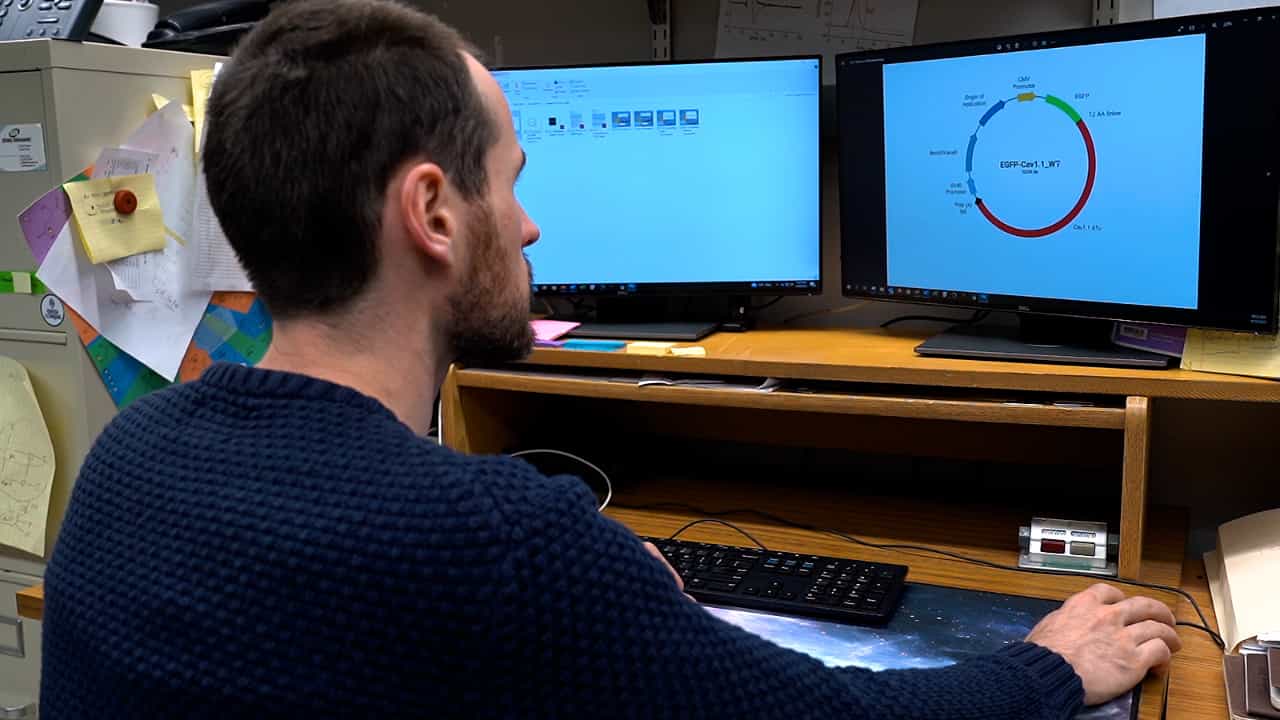
Functional Site-Directed Fluorometry in Native Cells to Study Skeletal Muscle Excitability
Published on: June 2, 2023
Molecular compatibility of the channel gate and the N terminus of S5 segment for voltage-gated channel activity
Marco Caprini1, Marianna Fava, Pierluigi Valente
1Department of Human and General Physiology, University of Bologna, Via San Donato 19/2, 40127 Bologna, Italy.

Abstract:
Voltage-gated ion channels are modular proteins designed by the structural linkage of a voltage sensor and a pore domain. The functional coupling of these two protein modules is a subject of intense research. A major focus has been directed to decipher the role of the S4-S5 linker and the C-end of the inner pore helix in channel gating. However, the contribution of the cytosolic N terminus of S5 remains elusive. To address this issue, we used a chimeric subunit that linked the voltage sensor of the Shaker channel to the prokaryotic KcsA pore domain (denoted as Shaker-KcsA). This chimera preserved the Shaker sequences at both the N terminus of S5 and the C-end of S6. Chimeric Shaker-KcsA subunits did not form functional homomeric channels but were synthesized, folded, and trafficked to the cell surface, as evidenced by their co-assembly with Shaker wild type subunits. Sequential substitution of Shaker amino acids at the C-end of S6 and the N terminus of S5 by the corresponding KcsA created voltage-sensitive channels with voltage-dependent properties that asymptotically approached those of the wild type Shaker channel. Noteworthy, substitution of the region encompassing Phe(401)-Phe(404) at the N-end of Shaker S5 by KcsA residues resulted in a significant gain in voltage sensitivity of the chimeras. Furthermore, analysis of channel function at high [K(+)](o) revealed that the Phe(401)-Phe(404) region is an important molecular determinant for competent coupling of voltage sensing and pore opening. Taken together, these findings indicate that complete replacement of Shaker S5 and S6 by KcsA M1 and M2 is required for voltage-dependent gating of the prokaryotic channel. In addition, our results imply that the region encompassing Phe(401)-Phe(404) in Shaker is involved in protein-protein interactions with the voltage sensor, and signal to the Phe(401) in the S5 segment as a key molecular determinant to pair the voltage sensor and the pore domain.
More Related Videos
Related Concept Videos
 01:26
Voltage-gated Ion Channels
Generally, all voltage-gated ion channels have a 'voltage-sensing domain' that spans the lipid bilayer. The charged residues in the sensor move in response to the membrane potential changes that open the channel allowing ions movement. There are several types of...
01:26Voltage-gated Ion Channels
Generally, all voltage-gated ion channels have a 'voltage-sensing domain' that spans the lipid bilayer. The charged residues in the sensor move in response to the membrane potential changes that open the channel allowing ions movement. There are several types of...
 01:24
Non-gated Ion Channels
Compared to the gated ion channels, the non-gated channels, also known as leakage or passive channels, have no gating mechanism.
01:24Non-gated Ion Channels
Compared to the gated ion channels, the non-gated channels, also known as leakage or passive channels, have no gating mechanism.
 01:30
Ligand-Gated Ion Channel Receptor: Gating Mechanism
 01:19
Ligand-gated Ion Channels
Three Subfamilies of Ligand-gated Ion Channels
Ligand-gated ion channels fall into three subfamilies. The 'Cys-loop' includes the nicotinic acetylcholine receptors, γ-aminobutyric acid (GABA), glycine, and 5-hydroxytryptamine receptors. The second one is the 'Pore-loop' channels that include the...