Identification of a novel, intraperoxisomal pex14-binding site in pex13: association of pex13 with the docking complex is essential for peroxisomal matrix protein import
Related Experiment Video
Updated: Aug 18, 2026
Peroxisome Staining in Mammalian Cells Using Peroxisome-Specific Probes
Published on: December 19, 2025
Annette Schell-Steven1, Katharina Stein, Mara Amoros
1Institut für Physiologische Chemie, Ruhr-Universität Bochum, D-44780 Bochum, Germany.

Insights
The peroxisomal docking complex
Area of Science:
- Cell Biology
- Molecular Biology
Background:
- The peroxisomal docking complex is crucial for importing matrix proteins.
- Pex14 is the core protein, serving as the docking site for Pex5 and Pex7 import receptors.
- Pex13 is another essential component associated with this complex.
Purpose of the Study:
- To investigate the interaction between Pex13 and Pex14.
- To elucidate the role of Pex5 in the Pex13-Pex14 association.
- To understand the functional significance of these interactions in peroxisomal protein import.
Main Methods:
- Investigated direct binding sites between Pex13 and Pex14 using biochemical assays.
- Utilized mutant strains to assess the impact of altered interactions on peroxisome function.
- Analyzed peroxisomal protein import pathways (PTS1 and PTS2) and growth phenotypes.
Main Results:
- Pex13 binds Pex14 directly via its SH3 domain and a novel intraperoxisomal site.
- Pex5 also contributes to Pex13's association with Pex14.
- Combined mutations severely impaired PTS1 import and oleic acid growth, while blocking SH3 interaction abolished PTS2 import.
Conclusions:
- The Pex13-Pex14 association is essential for peroxisomal protein import, involving multiple interaction modes.
- Pex5 plays a role in this association, suggesting a novel receptor-independent function.
- Understanding these interactions provides insights into peroxisome biogenesis and function.
Abstract:
The peroxisomal docking complex is a key component of the import machinery for matrix proteins. The core protein of this complex, Pex14, is thought to represent the initial docking site for the import receptors Pex5 and Pex7. Associated with this complex is a fraction of Pex13, another essential component of the import machinery. Here we demonstrate that Pex13 directly binds Pex14 not only via its SH3 domain but also via a novel intraperoxisomal site. Furthermore, we demonstrate that Pex5 also contributes to the association of Pex13 with Pex14. Peroxisome function was affected only mildly by mutations within the novel Pex14 interaction site of Pex13 or by the non-Pex13-interacting mutant Pex5(W204A). However, when these constructs were tested in combination, PTS1-dependent import and growth on oleic acid were severely compromised. When the SH3 domain-mediated interaction of Pex13 with Pex14 was blocked on top of that, PTS2-dependent matrix protein import was completely compromised and Pex13 was no longer copurified with the docking complex. We conclude that the association of Pex13 with Pex14 is an essential step in peroxisomal protein import that is enabled by two direct interactions and by one that is mediated by Pex5, a result which indicates a novel, receptor-independent function of Pex5.
Related Concept Videos
 01:27
Protein Import into the Peroxisomes
Peroxisomal Protein Import:
Peroxisomes lack the genetic machinery required to code for their own proteins. Hence, most peroxisomal membrane, lumenal and transmembrane proteins are synthesized in the cytoplasm or ER and transported to the peroxisome...
 01:21
Structure of Porins
 01:19
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
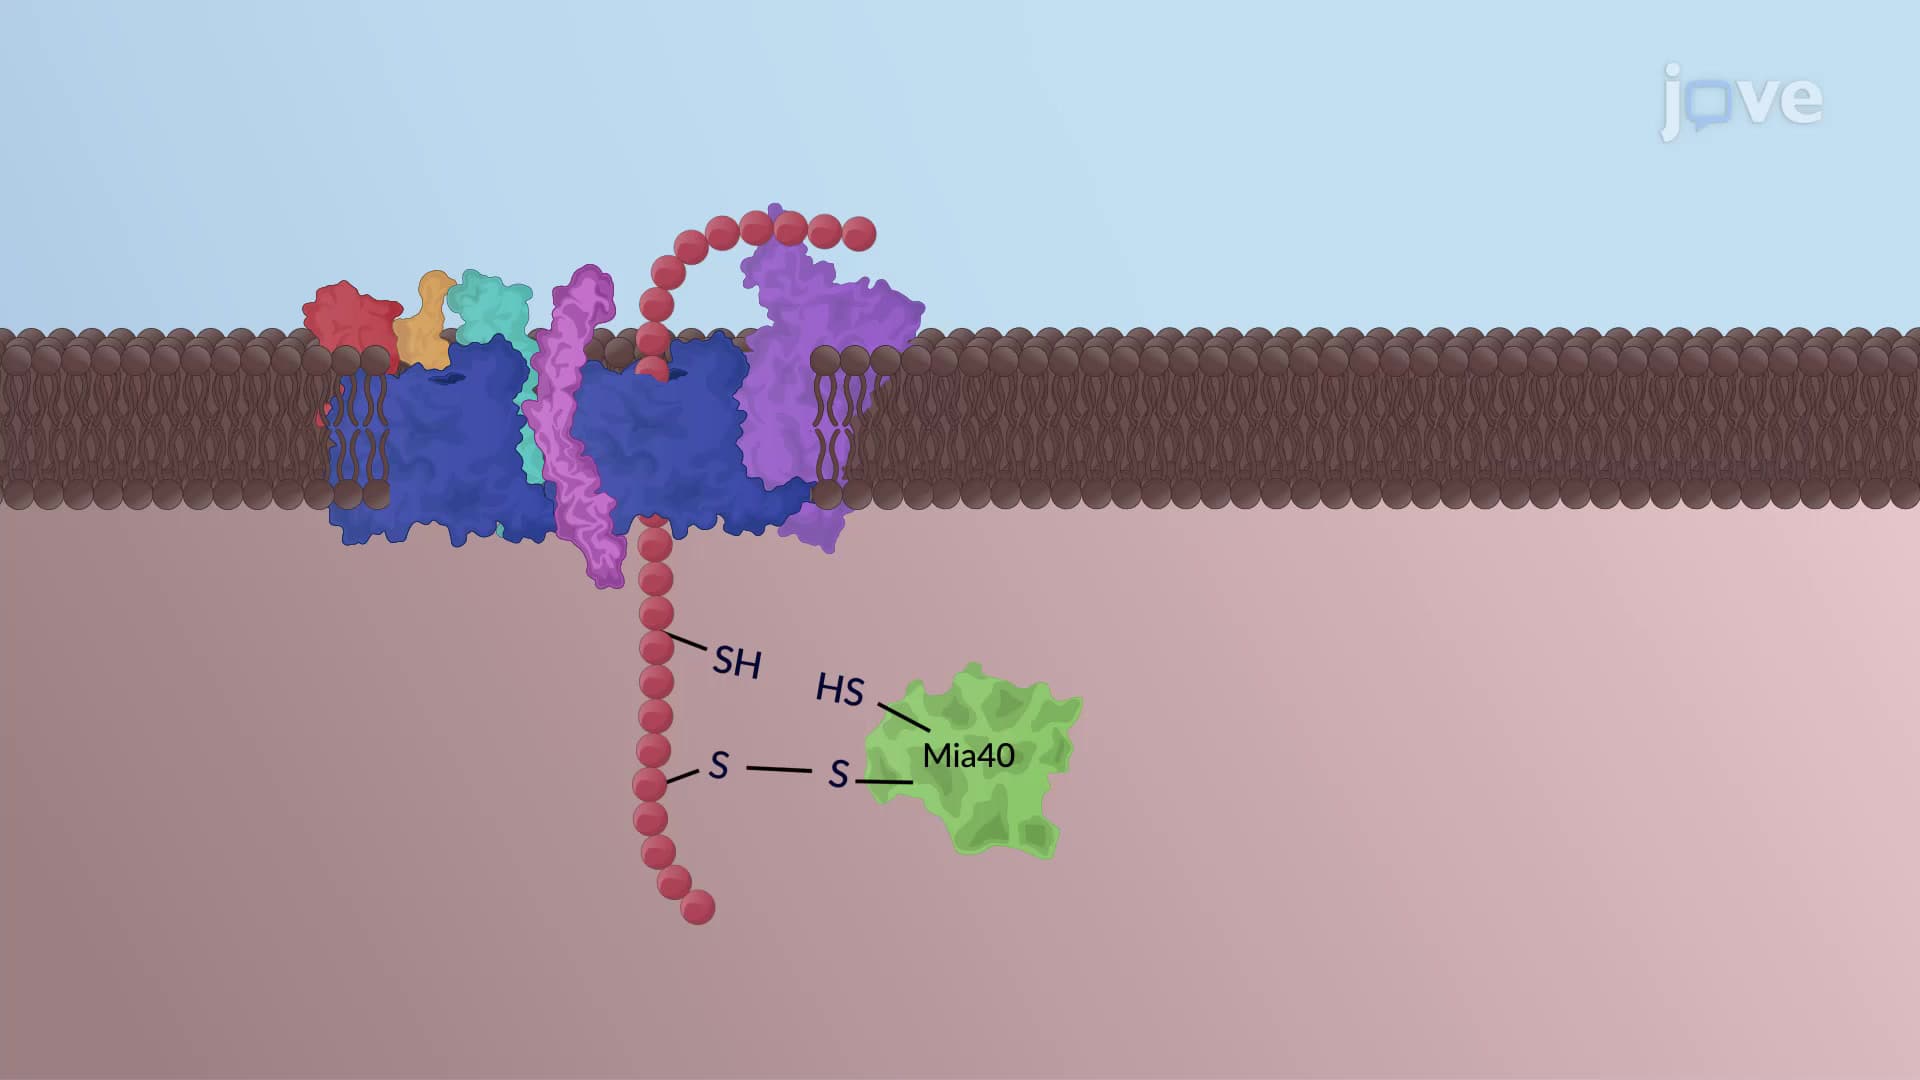
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:46
Nuclear Localization Signals and Import
 01:34
Protein Transport into the Inner Mitochondrial Membrane
Transport of mitochondrial precursors across the TIM23 channel is driven by...
 01:12
Porin Insertion in the Outer Mitochondrial Membrane
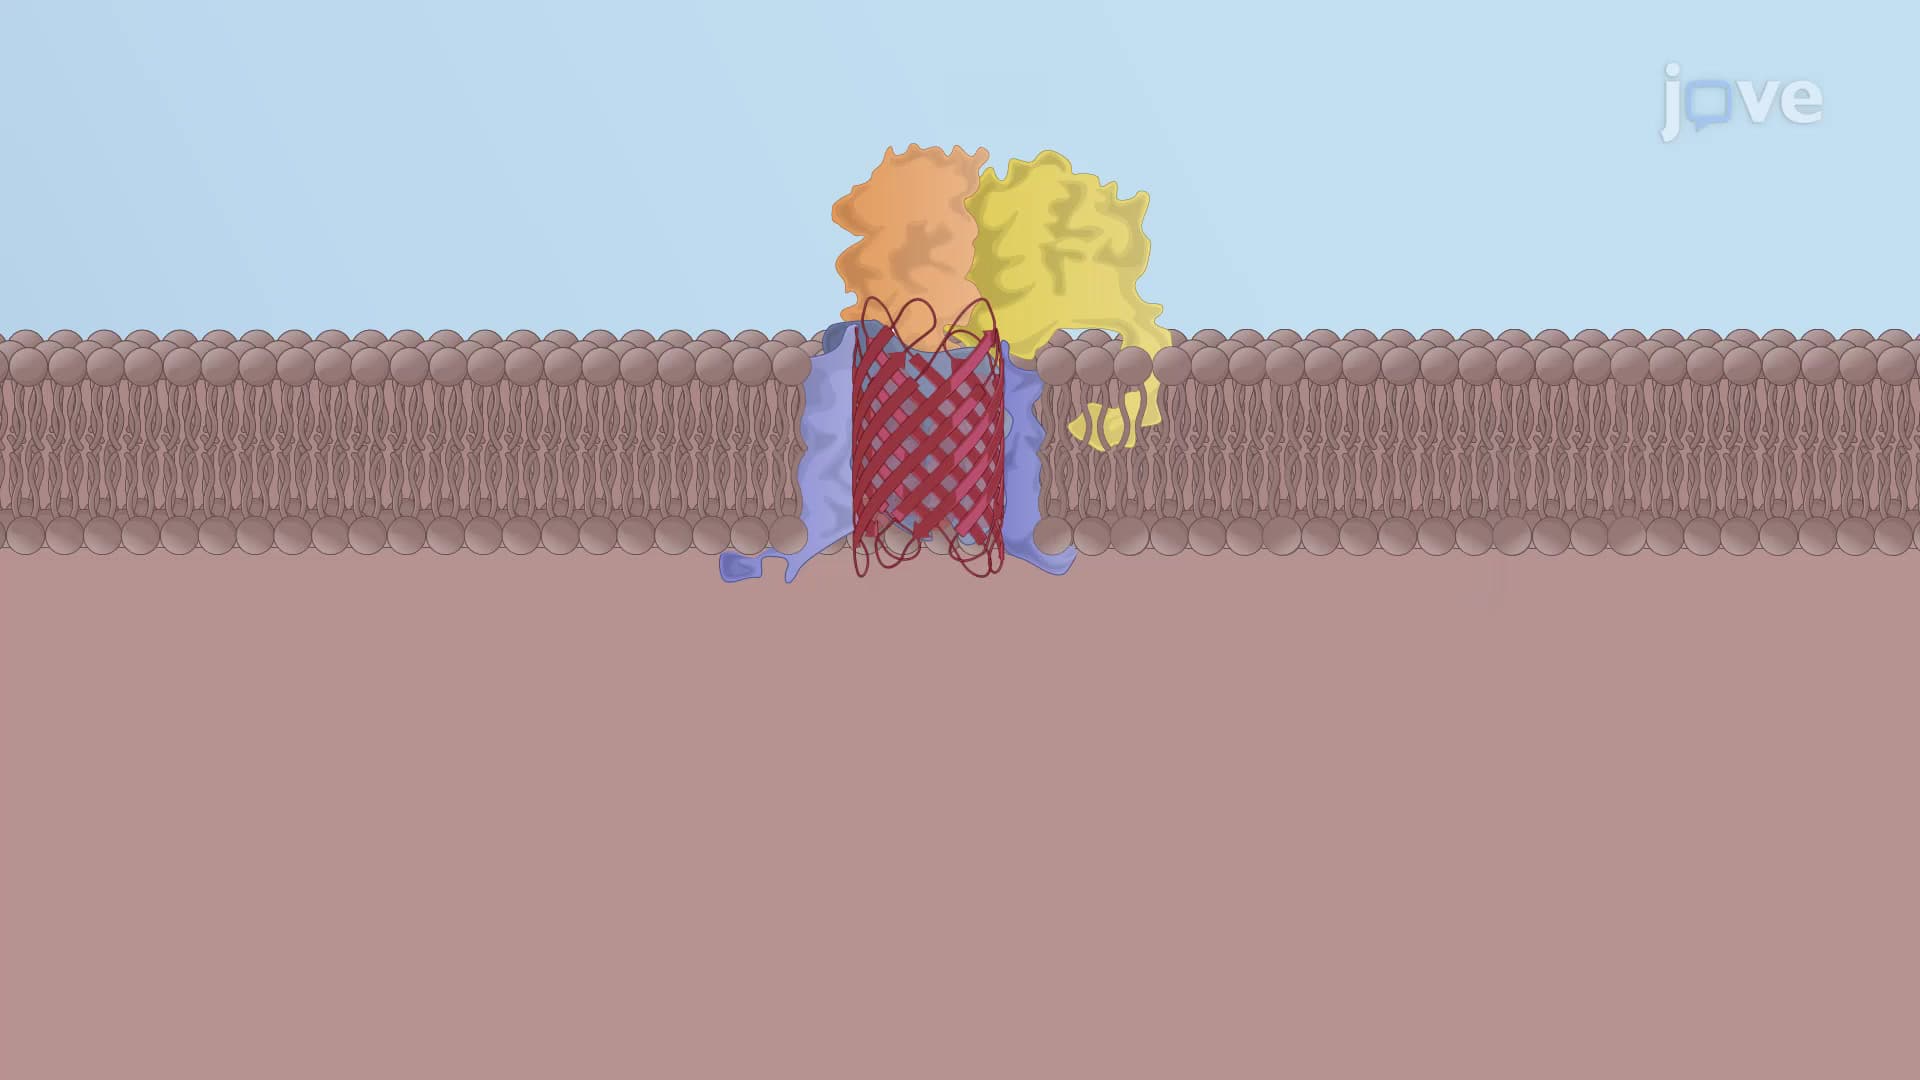
Three models describe the assembly of porins by the SAM complex and their insertion into the outer membrane. Model 1 suggests that porins are assembled outside the SAM channel as the...