Related Experiment Video
Updated: Aug 17, 2026

Defining Hsp33's Redox-regulated Chaperone Activity and Mapping Conformational Changes on Hsp33 Using Hydrogen-deuterium Exchange Mass Spectrometry
Published on: June 7, 2018
Structure of unliganded GRP94, the endoplasmic reticulum Hsp90. Basis for nucleotide-induced conformational change
D Eric Dollins1, Robert M Immormino, Daniel T Gewirth
1Department of Biochemistry, Duke University Medical Center, Durham, North Carolina 27710, USA.

Abstract:
GRP94, the endoplasmic reticulum paralog of Hsp90, is regulated by adenosine nucleotides that bind to its N-terminal regulatory domain. Because of its weak affinity for nucleotides, the functionally relevant transition in GRP94 is likely to be between the unliganded and nucleotide-bound states. We have determined the structure of the unliganded GRP94 N-domain. The helix 1-4-5 subdomain of the unliganded protein adopts the closed conformation seen in the structure of the protein in complex with inhibitors. This conformation is distinct from the open conformation of the subdomain seen when the protein is bound to ATP or ADP. ADP soaked into crystals of the unliganded protein reveals an intermediate conformation midway between the open and closed states and demonstrates that in GRP94 the conversion between the open and closed states is driven by ligand binding. The direction of the observed movement in GRP94 shows that nucleotides act to open the subdomain elements rather than close them, which is contrary to the motion proposed for Hsp90. These observations support a model where ATP binding dictates the conformation of the N-domain and regulates its ability to form quaternary structural interactions.
Related Concept Videos
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum
 03:00
Molecular Chaperones and Protein Folding
The...
 01:31
Regulation of the Unfolded Protein Response
 01:27
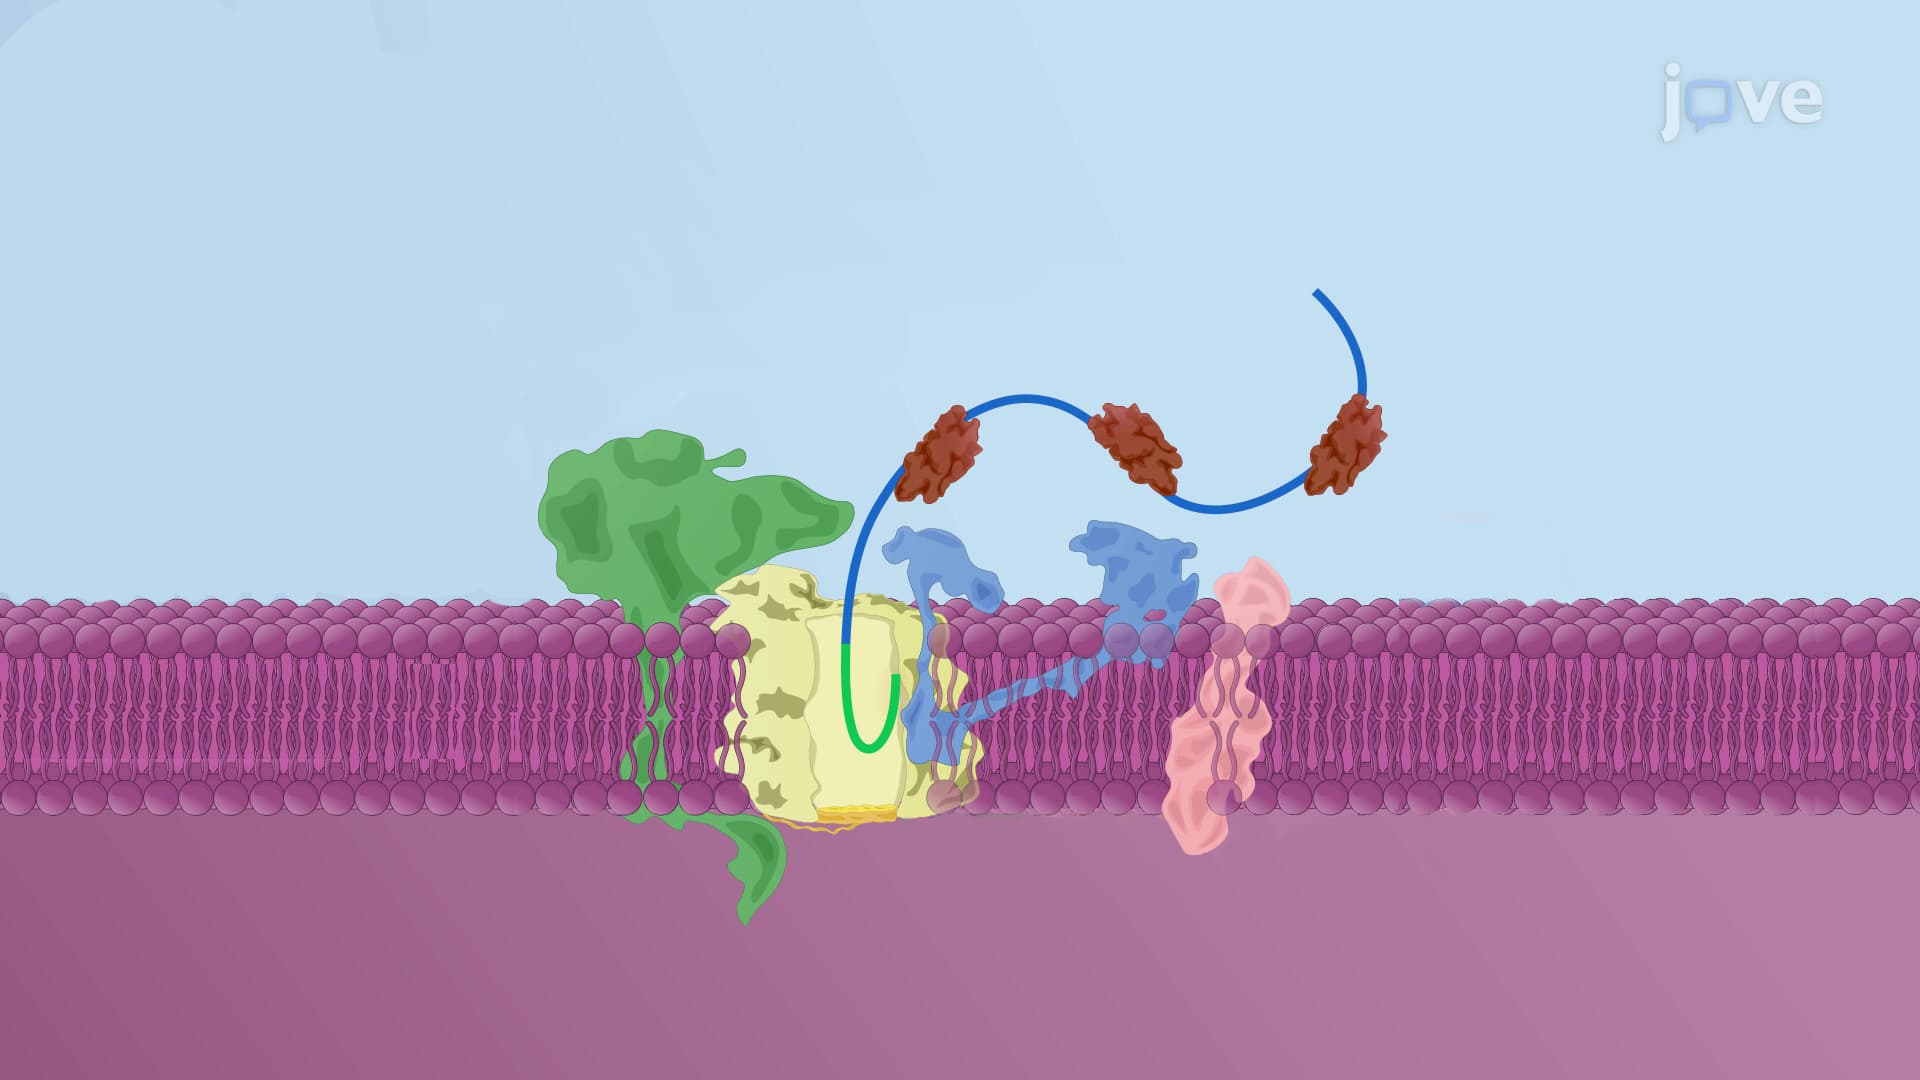
Post-translational Translocation of Proteins to the RER
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
 01:20
Cotranslational Protein Translocation
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
 01:32
Export of Misfolded Proteins out of the ER