Related Experiment Video
Updated: Aug 17, 2026

Functional Site-Directed Fluorometry in Native Cells to Study Skeletal Muscle Excitability
Published on: June 2, 2023
Carboxy-terminal truncations modify the outer pore vestibule of muscle chloride channels
Simon Hebeisen1, Christoph Fahlke
1Department of Physiology, RWTH Aachen, Aachen, Germany.

Abstract:
Mammalian ClC-type chloride channels have large cytoplasmic carboxy-terminal domains whose function is still insufficiently understood. We investigated the role of the distal part of the carboxy-terminus of the muscle isoform ClC-1 by constructing and functionally evaluating two truncation mutants, R894X and K875X. Truncated channels exhibit normal unitary conductances and anion selectivities but altered apparent anion binding affinities in the open and in the closed state. Since voltage-dependent gating is strictly coupled to ion permeation in ClC-1 channels, the changed pore properties result in different fast and slow gating. Full length and truncated channels also differed in methanethiosulphonate (MTS) modification rate constants of an engineered cysteine at position 231 near the selectivity filter. Our data demonstrate that the carboxy-terminus of ClC channels modifies the conformation of the outer pore vestibule.
Insights
The carboxy-terminus of muscle chloride channel ClC-1 influences ion binding and gating by altering the outer pore vestibule conformation. This study reveals key insights into ClC channel function.
Area of Science:
- Molecular biology
- Biophysics
- Ion channel research
Background:
- Mammalian ClC-type chloride channels possess large, functionally uncharacterized cytoplasmic carboxy-terminal domains.
- The muscle isoform, ClC-1, is crucial for muscle membrane potential and function.
Purpose of the Study:
- To investigate the role of the distal carboxy-terminus of the muscle ClC-1 chloride channel.
- To determine how truncations in this domain affect channel function, including ion permeation and gating.
Main Methods:
- Construction and functional evaluation of two ClC-1 truncation mutants (R894X and K875X).
- Assessment of unitary conductances, anion selectivities, and apparent anion binding affinities.
- Analysis of voltage-dependent gating kinetics and methanethiosulphonate (MTS) modification rates.
Main Results:
- Truncated ClC-1 channels retained normal unitary conductances and anion selectivities.
- Altered apparent anion binding affinities were observed in both open and closed states of truncated channels.
- Changes in pore properties led to modified fast and slow gating kinetics.
- Differences in MTS modification rates at cysteine 231 were noted between full-length and truncated channels.
Conclusions:
- The carboxy-terminus of ClC-1 channels significantly impacts the outer pore vestibule conformation.
- This conformational modification influences ion binding and voltage-dependent gating.
- The distal carboxy-terminus plays a critical role in regulating ClC-1 channel function.
More Related Videos
 12:48
Measuring Cation Transport by Na,K- and H,K-ATPase in Xenopus Oocytes by Atomic Absorption Spectrophotometry: An Alternative to Radioisotope Assays
Published on: February 19, 2013
 10:45
Levator Auris Longus Preparation for Examination of Mammalian Neuromuscular Transmission Under Voltage Clamp Conditions
Published on: May 5, 2018
Related Concept Videos
 01:09
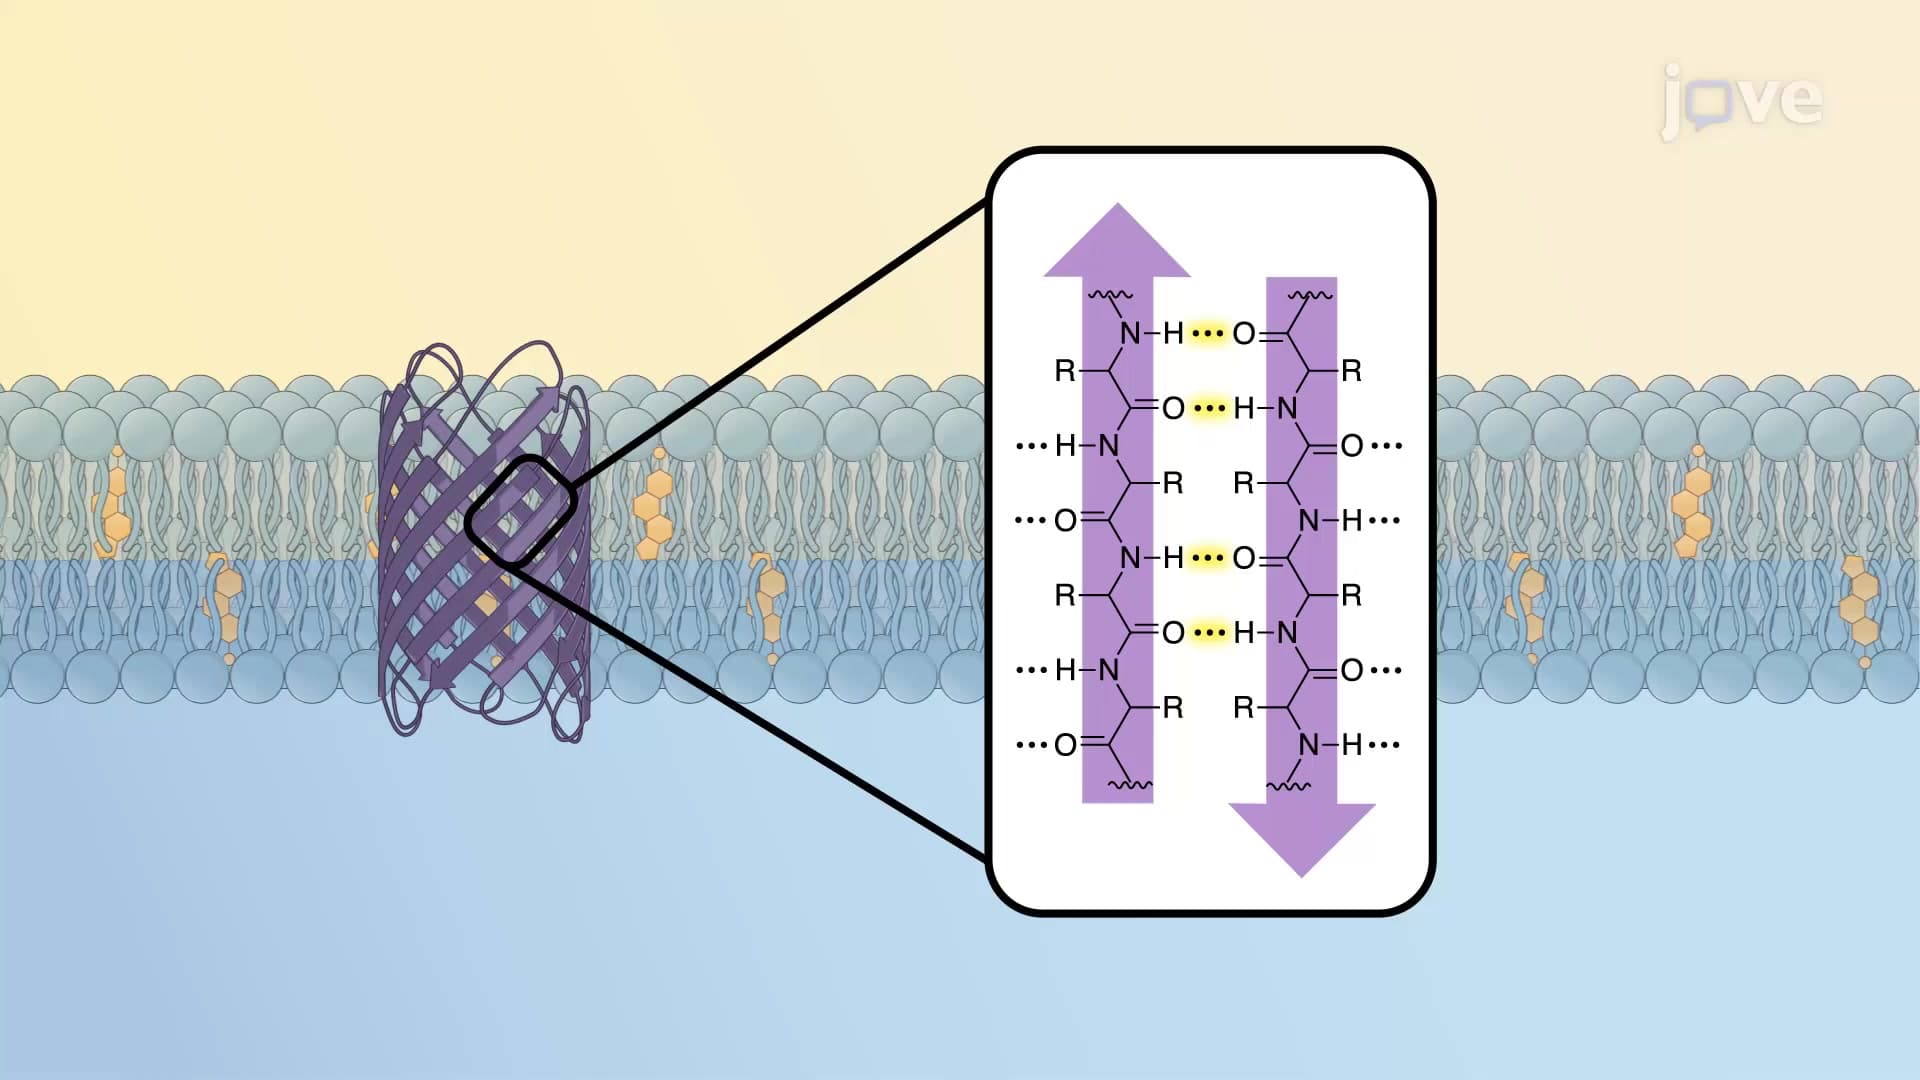
Multi-pass Transmembrane Proteins and β-barrels
α-Helix containing multi-pass transmembrane proteins
Multi-pass transmembrane proteins such as G-protein-linked receptors (GPCRs) and...
 01:26
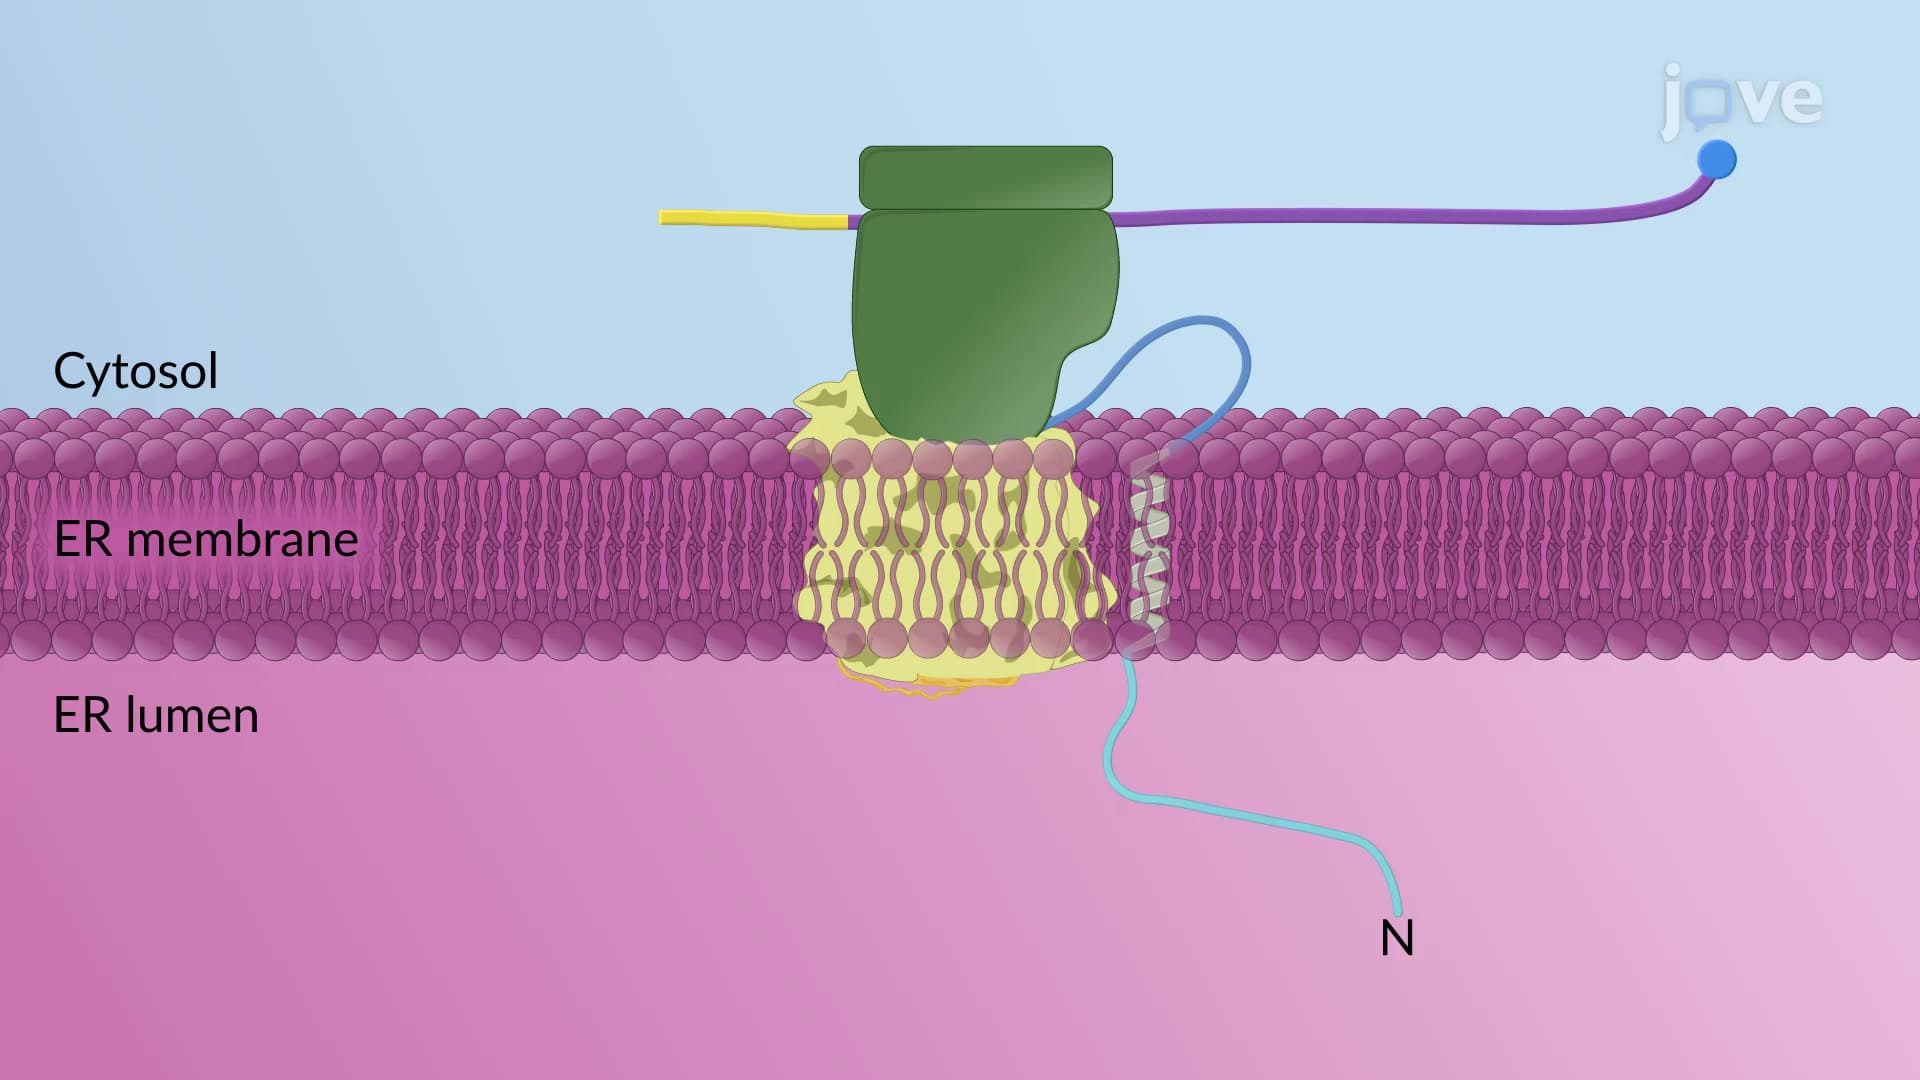
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:12
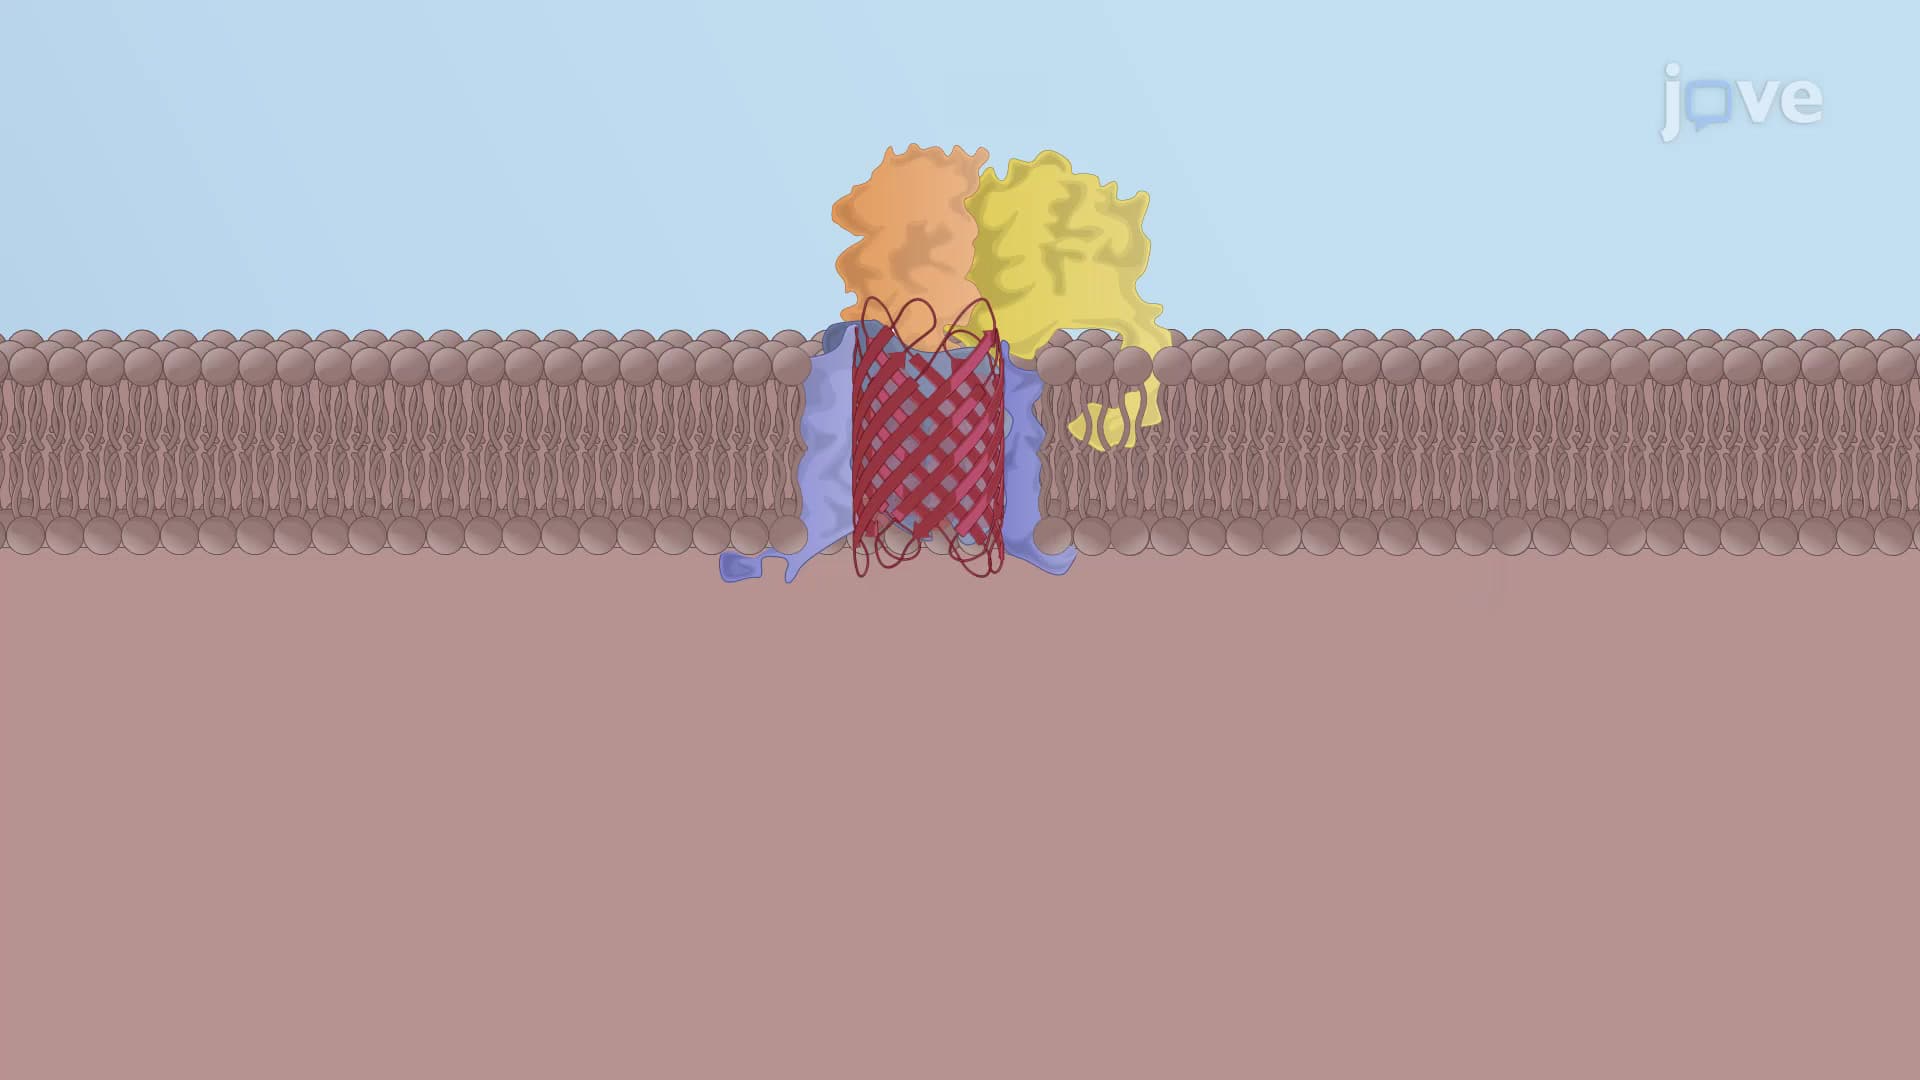
Porin Insertion in the Outer Mitochondrial Membrane
Three models describe the assembly of porins by the SAM complex and their insertion into the outer membrane. Model 1 suggests that porins are assembled outside the SAM channel as the...
 01:39
Mitochondrial Precursor Proteins
Most of the mitochondrial precursors...
 01:12
Clathrin Coated Vesicles
 01:19
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...