Related Experiment Video
Updated: Aug 16, 2026
Monitoring GPCR-β-arrestin1/2 Interactions in Real Time Living Systems to Accelerate Drug Discovery
Published on: June 28, 2019
ARF directly binds DP1: interaction with DP1 coincides with the G1 arrest function of ARF
Abhishek Datta1, Jayita Sen, Jussara Hagen
1Department of Biochemistry and Molecular Genetics, University of Illinois at Chicago, 900 S. Ashland Ave., Chicago, IL 60607, USA.

Abstract:
The tumor suppressor ARF inhibits cell growth in response to oncogenic stress in a p53-dependent manner. Also, there is an increasing appreciation of ARF's ability to inhibit cell growth via multiple p53-independent mechanisms, including its ability to regulate the E2F pathway. We have investigated the interaction between the tumor suppressor ARF and DP1, the DNA binding partner of the E2F family of factors (E2Fs). We show that ARF directly binds to DP1. Interestingly, binding of ARF to DP1 results in an inhibition of the interaction between DP1 and E2F1. Moreover, ARF regulates the association of DP1 with its target gene, as evidenced by a chromatin immunoprecipitation assay with the dhfr promoter. By analyzing a series of ARF mutants, we demonstrate a strong correlation between ARF's ability to regulate DP1 and its ability to cause cell cycle arrest. S-phase inhibition by ARF is preceded by an inhibition of the E2F-activated genes. Moreover, we provide evidence that ARF inhibits the E2F-activated genes independently of p53 and Mdm2. Also, the interaction between ARF and DP1 is enhanced during oncogenic stress and "culture shock." Taken together, our results show that DP1 is a critical direct target of ARF.
Insights
The tumor suppressor ARF directly binds to DP1, inhibiting E2F1 interaction and regulating gene association. This ARF-DP1 interaction is crucial for ARF-mediated cell cycle arrest, independent of p53.
Area of Science:
- Molecular Biology
- Cell Biology
- Oncology
Background:
- The tumor suppressor ARF inhibits cell growth, often via p53-dependent pathways.
- ARF also exhibits p53-independent mechanisms for cell growth inhibition, including regulation of the E2F pathway.
Purpose of the Study:
- To investigate the interaction between the tumor suppressor ARF and DP1, a key component of the E2F transcription factor complex.
- To elucidate the role of the ARF-DP1 interaction in ARF-mediated cell cycle regulation.
Main Methods:
- Direct binding assays to confirm ARF-DP1 interaction.
- Co-immunoprecipitation to assess the effect of ARF on DP1-E2F1 interaction.
- Chromatin immunoprecipitation (ChIP) assays to evaluate DP1 association with target gene promoters.
- Analysis of ARF mutants to correlate DP1 regulation with cell cycle arrest.
- Assays to determine p53 and Mdm2 independence.
Main Results:
- ARF directly binds to DP1.
- ARF binding to DP1 inhibits the interaction between DP1 and E2F1.
- ARF regulates DP1's association with target gene promoters, such as the dhfr promoter.
- ARF-induced cell cycle arrest, specifically S-phase inhibition, correlates with ARF's ability to regulate DP1.
- ARF inhibits E2F-activated genes independently of p53 and Mdm2.
- ARF-DP1 interaction is enhanced under oncogenic stress and culture shock conditions.
Conclusions:
- DP1 is a critical direct target of the tumor suppressor ARF.
- The ARF-DP1 interaction is a key p53-independent mechanism by which ARF inhibits cell growth and induces cell cycle arrest.
More Related Videos
Related Concept Videos
 02:36
DNA Damage can Stall the Cell Cycle
02:36DNA Damage Can Stall the Cell Cycle
 01:14
Generation of Straight or Branched Actin Filaments
Arp2/3 Complex
Arp2/3 complex is a seven-subunit complex consisting of two proteins similar to actin- Arp2 and Arp3, and five other subunits that help keep Arp2 and Arp3 inactive. When required, the complex is...
 01:14
Rab Proteins
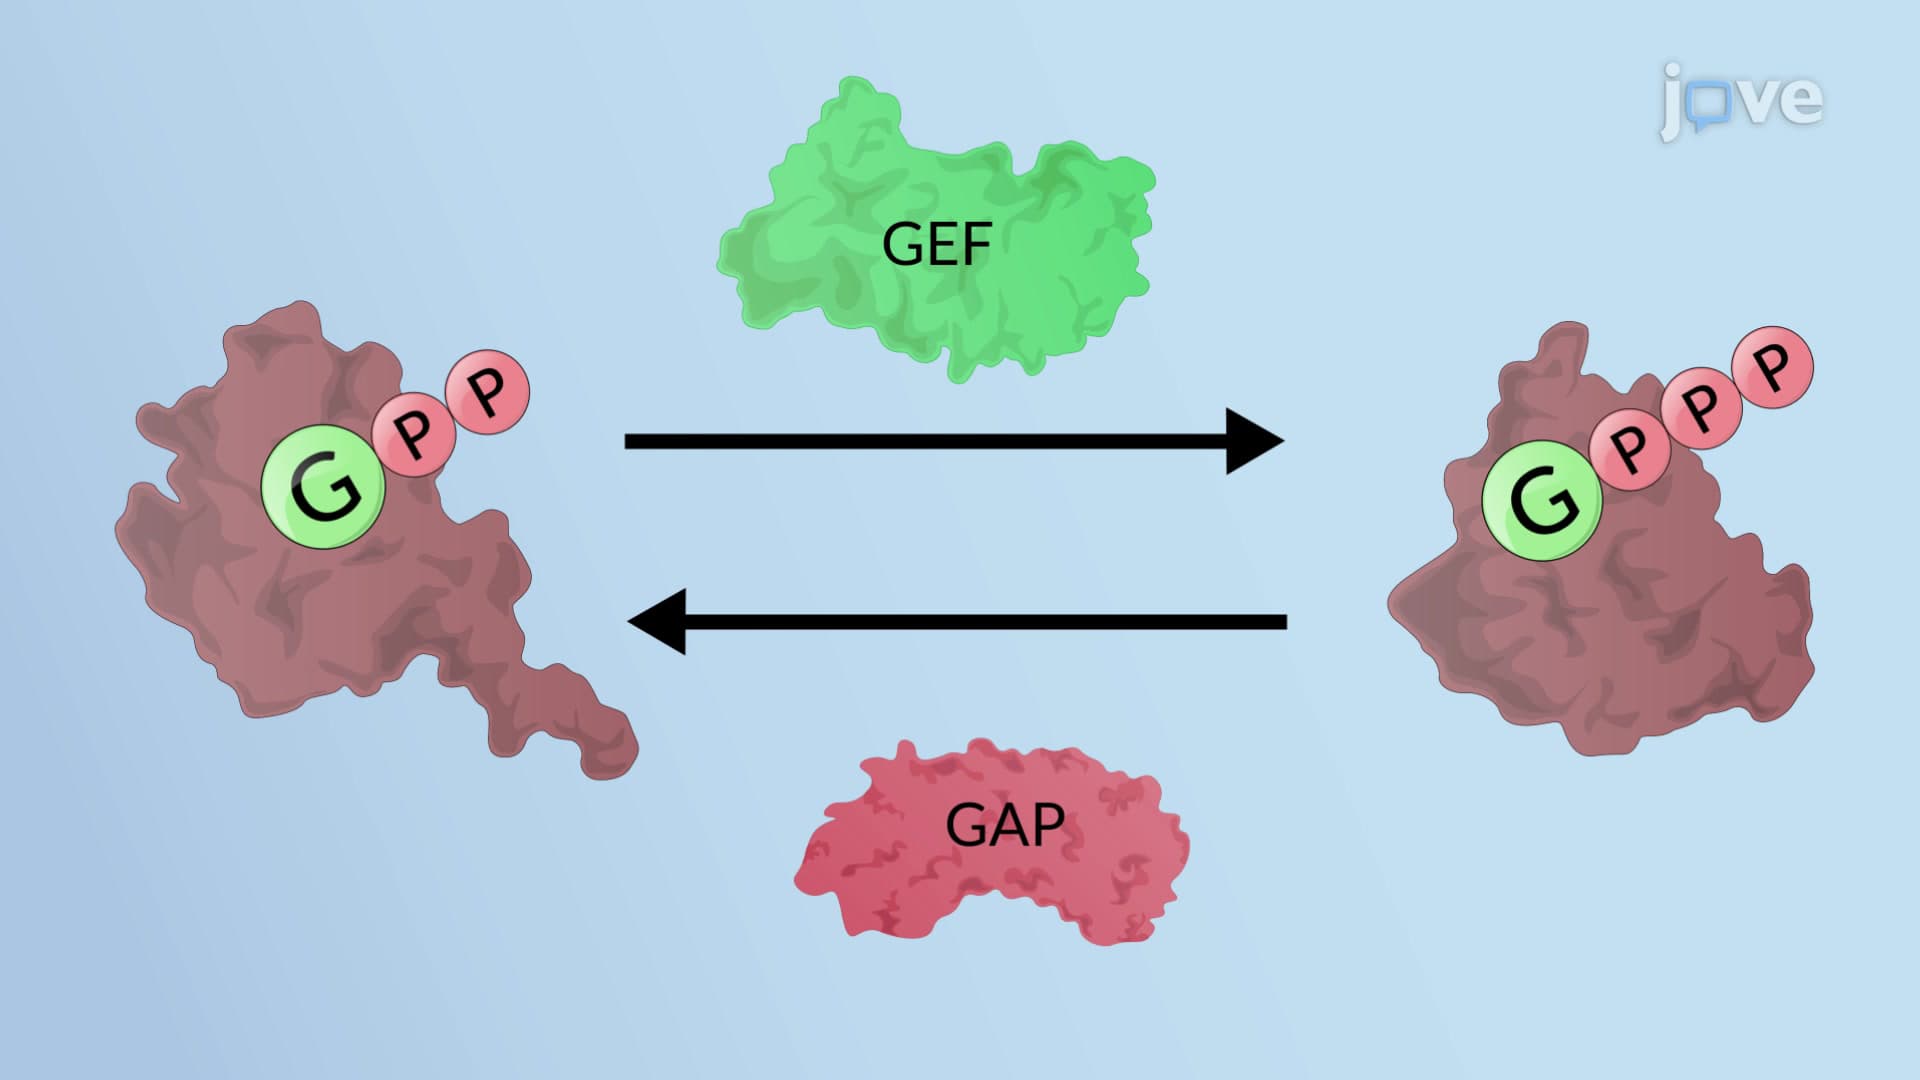
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum
 01:09
GPCRs Regulate Adenylyl Cylase Activity
Two...