Related Experiment Video
Updated: Aug 15, 2026
08:04

Assembling Molecular Shuttles Powered by Reversibly Attached Kinesins
Published on: January 26, 2019
Structural evidence of mechanical shuttling in condensed monolayers of bistable rotaxane molecules
Kasper Nørgaard1, Bo W Laursen, Sune Nygaard
1Nano-Science Center, University of Copenhagen, Universitetsparken 5, 2100 København, Denmark.
Angewandte Chemie (International Ed. in English)
|October 12, 2005

Abstract
No abstract available in PubMed .
Related Concept Videos
 00:52
¹H NMR of Conformationally Flexible Molecules: Temporal Resolution
At room temperature, the chair conformer of cyclohexane undergoes rapid ring flipping between two equivalent chair conformers at a rate of approximately 105 times per second. These two chair conformers are in equilibrium. The rapid ring flipping results in the interconversion of the axial proton to an equatorial proton and an equatorial to the axial proton. Such interconversions are too rapid and cannot be detected on the NMR timescale. Hence, the NMR spectrometer cannot distinguish between the...
 01:32
Pinching-off of Coated Vesicles
Vesicle budding is orchestrated by distinct cytosolic proteins such as adaptor proteins, coat proteins, and GTPases. To initiate vesicle budding, membrane-bending proteins containing crescent-shaped BAR domains bind to the lipid heads in the bilayer and distort the membrane to form a protein-coated vesicle bud. Adaptors proteins such as AP2 for clathrin-coated vesicles can nucleate on the deformed membrane. Finally, coat proteins such as clathrin or COPI and COPII assemble into a coat forming...
 02:02
Chair Conformation of Cyclohexane
The chair conformation is the most stable form of cyclohexane due to the absence of angle and torsional strain. The absence of angle strain is a result of cyclohexane’s bond angle being very close to the ideal tetrahedral bond angle of 109.5° in its chair conformer. Similarly, the torsional strain is also absent owing to the perfectly staggered arrangement of bonds.
The hydrogen atoms linked to carbons are arranged in two different axial and equatorial orientations to achieve this staggered...
The hydrogen atoms linked to carbons are arranged in two different axial and equatorial orientations to achieve this staggered...
 01:43
The Movement of Organelles and Vesicles
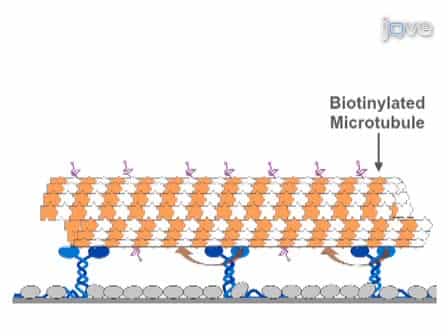
In eukaryotic cells, cytoskeletal filaments such as actin, microtubules, and intermediate filaments form a mesh-like cytoskeletal network. These filaments serve as tracks for transporting cellular cargo. Specialized motor proteins use the chemical energy stored in adenosine triphosphate (ATP) for this transport. During interphase, microtubules are polarized, with the plus-end towards the cell periphery and the minus-end towards the cell center. Two microtubule-associated motor proteins,...
 02:30
Stability of Substituted Cyclohexanes
This lesson discusses the stability of substituted cyclohexanes with a focus on energies of various conformers and the effect of 1,3-diaxial interactions.
The two chair conformations of cyclohexanes undergo rapid interconversion at room temperature. Both forms have identical energies and stabilities, each comprising equal amounts of the equilibrium mixture. Replacing a hydrogen atom with a functional group makes the two conformations energetically non-equivalent.
For example, in...
The two chair conformations of cyclohexanes undergo rapid interconversion at room temperature. Both forms have identical energies and stabilities, each comprising equal amounts of the equilibrium mixture. Replacing a hydrogen atom with a functional group makes the two conformations energetically non-equivalent.
For example, in...
 01:05
Mechanism of Ciliary Motion
The ciliary structures were first seen in 1647 by Antonie Leeuwenhoek while observing the protozoans. In lower organisms, these appendages are responsible for cell movement, while in higher organisms, these appendages help in the movement of the extracellular fluids within the body cavities.
The cilia are made up of microtubules in a 9+2 arrangement, with nine microtubule doublet ring bundles, surrounding a pair of central singlet microtubule bundles. The doublet microtubule bundles are...
The cilia are made up of microtubules in a 9+2 arrangement, with nine microtubule doublet ring bundles, surrounding a pair of central singlet microtubule bundles. The doublet microtubule bundles are...