Related Experiment Video
Updated: Aug 10, 2026

Patch Clamp and Perfusion Techniques for Studying Ion Channels Expressed in Xenopus oocytes
Published on: January 10, 2011
Quantitative analysis of the voltage-dependent gating of mouse parotid ClC-2 chloride channel
Jose Antonio de Santiago1, Keith Nehrke, Jorge Arreola
1Instituto de Física, Universidad Autonóma de San Luis Potosí, San Luis Potosí, SLP 78290, México.

Abstract:
Various ClC-type voltage-gated chloride channel isoforms display a double barrel topology, and their gating mechanisms are thought to be similar. However, we demonstrate in this work that the nearly ubiquitous ClC-2 shows significant differences in gating when compared with ClC-0 and ClC-1. To delineate the gating of ClC-2 in quantitative terms, we have determined the voltage (V(m)) and time dependence of the protopore (P(f)) and common (P(s)) gates that control the opening and closing of the double barrel. mClC-2 was cloned from mouse salivary glands, expressed in HEK 293 cells, and the resulting chloride currents (I(Cl)) were measured using whole cell patch clamp. WT channels had I(Cl) that showed inward rectification and biexponential time course. Time constants of fast and slow components were approximately 10-fold different at negative V(m) and corresponded to P(f) and P(s), respectively. P(f) and P(s) were approximately 1 at -200 mV, while at V(m) > or = 0 mV, P(f) approximately 0 and P(s) approximately 0.6. Hence, P(f) dominated open kinetics at moderately negative V(m), while at very negative V(m) both gates contributed to gating. At V(m) > or = 0 mV, mClC-2 closes by shutting off P(f). Three- and two-state models described the open-to-closed transitions of P(f) and P(s), respectively. To test these models, we mutated conserved residues that had been previously shown to eliminate or alter P(f) or P(s) in other ClC channels. Based on the time and V(m) dependence of the two gates in WT and mutant channels, we constructed a model to explain the gating of mClC-2. In this model the E213 residue contributes to P(f), the dominant regulator of gating, while the C258 residue alters the V(m) dependence of P(f), probably by interacting with residue E213. These data provide a new perspective on ClC-2 gating, suggesting that the protopore gate contributes to both fast and slow gating and that gating relies strongly on the E213 residue.
Related Concept Videos
 01:18
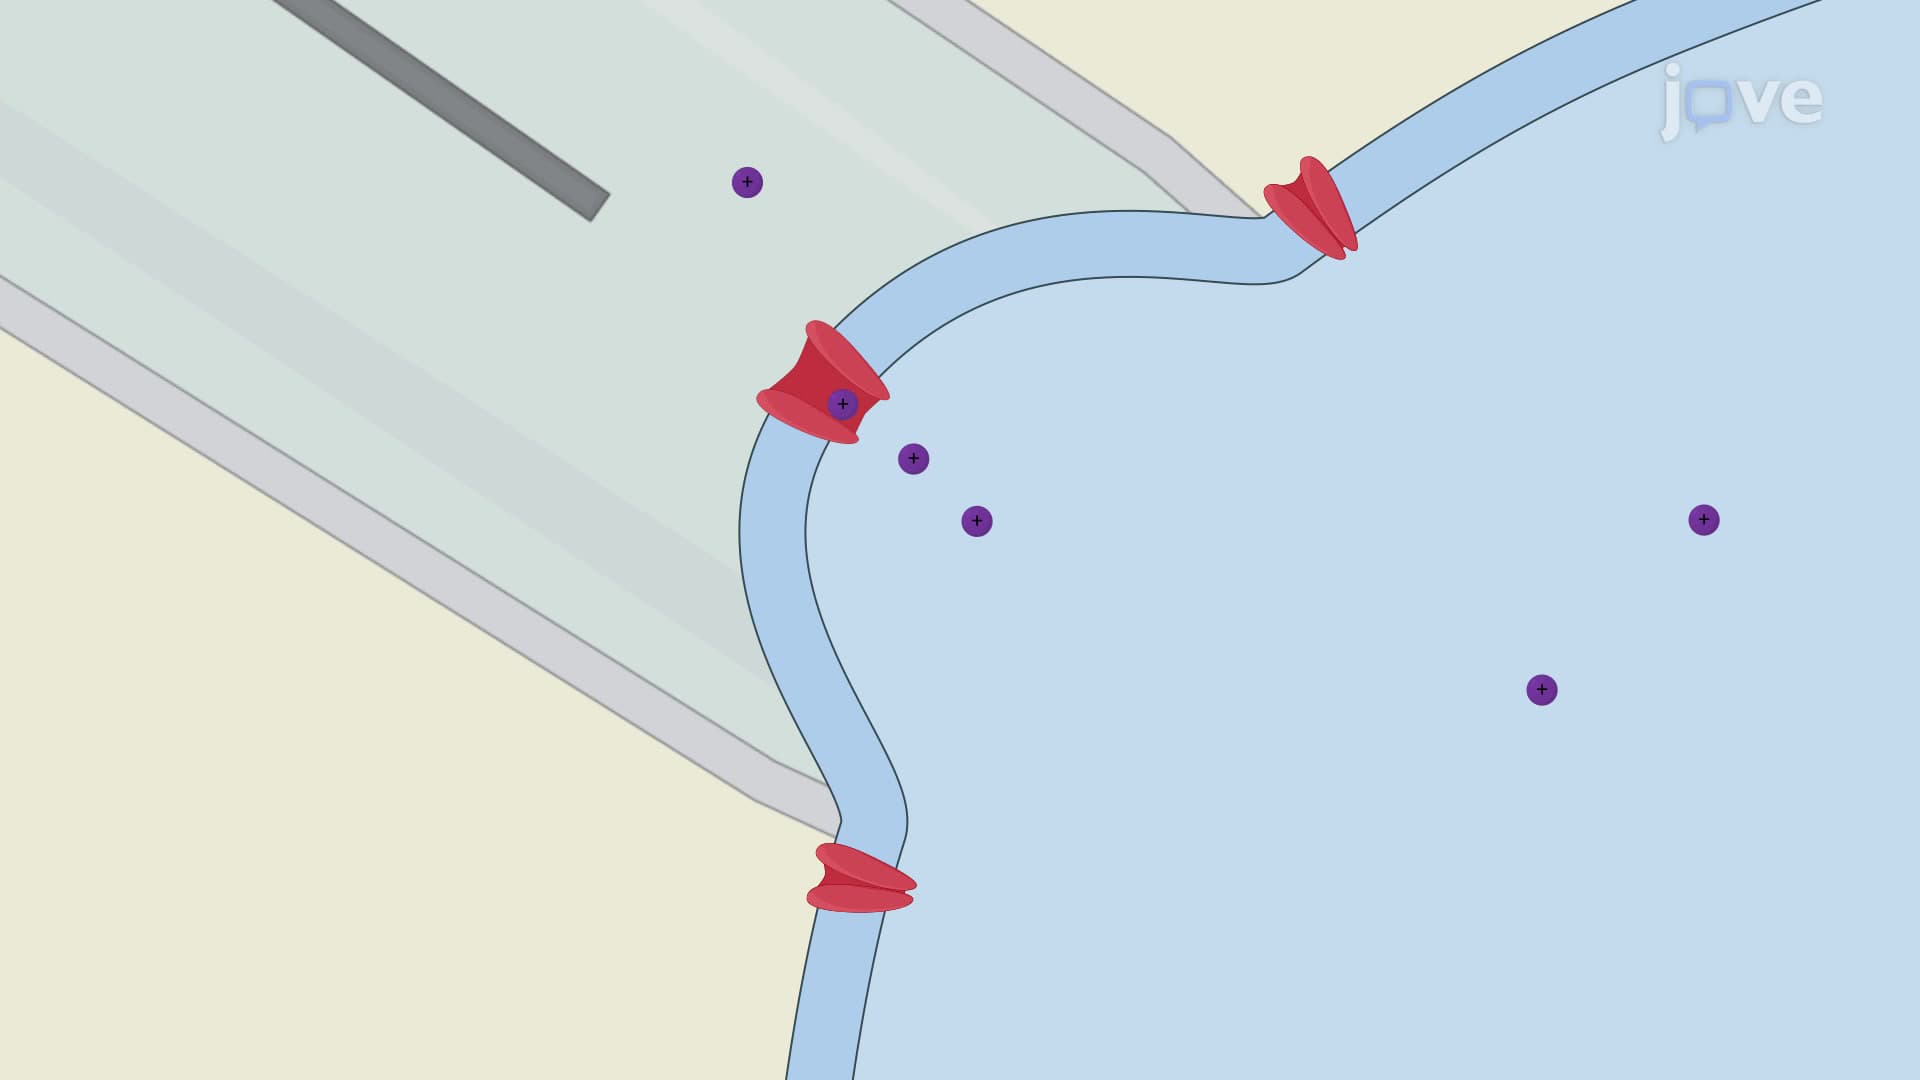
Patch Clamp
In this method, a glass micropipette containing electrolyte solution is tightly sealed against a small portion of the cell membrane. As a result, a patch of the cell...
 01:19
Ligand-gated Ion Channels
Three Subfamilies of Ligand-gated Ion Channels
Ligand-gated ion channels fall into three subfamilies. The 'Cys-loop' includes the nicotinic acetylcholine receptors, γ-aminobutyric acid (GABA), glycine, and 5-hydroxytryptamine receptors. The second one is the 'Pore-loop' channels that include the...
 01:26
Voltage-gated Ion Channels
Generally, all voltage-gated ion channels have a 'voltage-sensing domain' that spans the lipid bilayer. The charged residues in the sensor move in response to the membrane potential changes that open the channel allowing ions movement. There are several types of...
01:26Voltage-gated Ion Channels
Generally, all voltage-gated ion channels have a 'voltage-sensing domain' that spans the lipid bilayer. The charged residues in the sensor move in response to the membrane potential changes that open the channel allowing ions movement. There are several types of...