Source of endoproteolytic activity associated with purified ribulose bisphosphate carboxylase

J L Rosichan1, R C Huffaker

  • 1Plant Growth Laboratory and the Department of Agronomy and Range Science, University of California, Davis, California 95616.

Plant Physiology
|May 1, 1984
PubMed

Related Concept Videos

The Calvin Benson Cycle01:46

The Calvin Benson Cycle

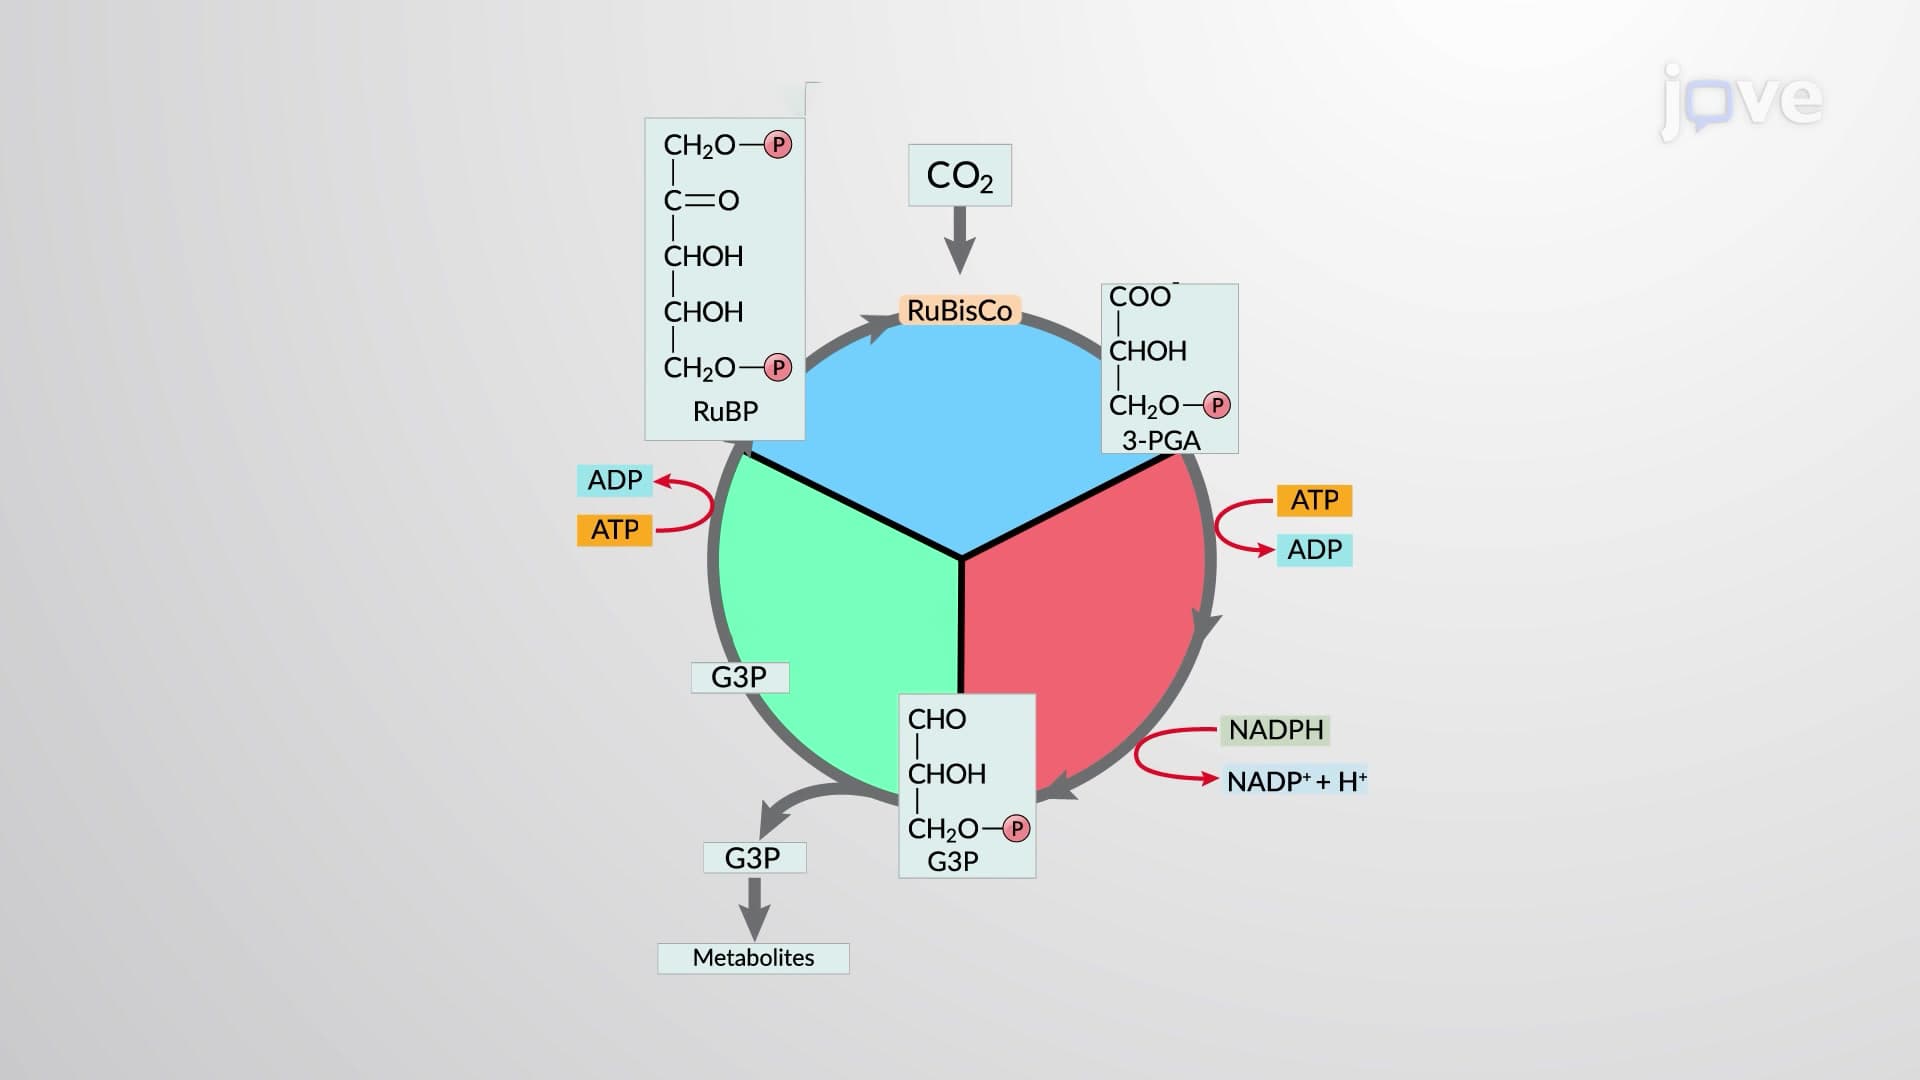
Ribulose 1,5- bisphosphate carboxylase/oxygenase (RuBisCo) is a critical enzyme that catalyzes carbon dioxide assimilation during photosynthesis. However, it is an inefficient enzyme, having an extremely slow catalytic rate. A typical enzyme can process about a thousand molecules per second; however, RuBisCo fixes only around three-carbon dioxides per second. Photosynthetic cells compensate for this slow rate by synthesizing very high amounts of RuBisCo, making it the most abundant single...
Allosteric Proteins-ATCase01:19

Allosteric Proteins-ATCase

Binding sites linkages can regulate a protein's function.  For example, enzyme activity is often regulated through a feedback mechanism where the end product of the biochemical process serves as an inhibitor.
Aspartate transcarbamoylase (ATCase) is a cytosolic enzyme that catalyzes the condensation of L-aspartate and carbamoyl phosphate to  N-carbamoyl-L-aspartate. This reaction is the first step in pyrimidine biosynthesis. UTP and CTP, the end products of the pyrimidine synthesis pathway,...
The Photochemical Reaction Center01:29

The Photochemical Reaction Center
Reaction centers are pigment-protein complexes that initiate energy conversion from photons to chemical entities. Therefore, photochemical reaction center is a more appropriate term that describes these complexes. The Nobel laureates Robert Emerson and William Arnold provided the first experimental evidence of photochemical reaction centers by demonstrating the participation of nearly 2,500 chlorophyll molecules for the release of just one molecule of oxygen. Despite thousands of photosynthetic...
Post-translational Translocation of Proteins to the RER01:27

Post-translational Translocation of Proteins to the RER

A sizable fraction of proteins destined for ER are first synthesized in the cell cytosol and then transported across the ER membrane–a process called post-translational translocation. Similar to cotranslationally translocated proteins, these proteins also use the Sec translocon complex to enter the ER lumen.
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
Export of Misfolded Proteins out of the ER01:32

Export of Misfolded Proteins out of the ER
After folding, the ER assesses the quality of secretory and membrane proteins. The correctly folded proteins are cleared by the calnexin cycle for transport to their final destination, while misfolded proteins are held back in the ER lumen. The ER chaperones attempt to unfold and refold the misfolded proteins but sometimes fail to achieve the correct native conformation. Such terminally misfolded proteins are then exported to the cytosol by ER-associated degradation or ERAD pathway for...
Protein Transport to the Outer Chloroplast Membrane01:11

Protein Transport to the Outer Chloroplast Membrane

Chloroplast outer membrane proteins encoded by the nucleus are synthesized in the cytosol. Soon after synthesis, they bind cytosolic factors such as 14-3-3 protein and the Hsp70 chaperones that keep these precursors in an unfolded state until their translocation.
Two models describe the mechanism of precursor recognition and entry across the outer membrane through the TOC complex. Model 1 suggests the newly synthesized precursor binds to the TOC receptor 159 and forms a complex.