Related Experiment Video
Updated: Aug 6, 2026

Microbiota of Attine Ants' Gardens: Visualizing a Microbial Landscape by Scanning Electron Microscopy
Published on: October 4, 2024
The growth and form of tunnelling networks in ants
Camille Buhl1, Jacques Gautrais, Jean Louis Deneubourg
1Centre de Recherches sur la Cognition Animale, CNRS UMR 5169, Université Paul Sabatier, 118 route de Narbonne, 31062 Toulouse Cedex 4, France. jerome.buhl@bio.usyd.edu.au <jerome.buhl@bio.usyd.edu.au>

Abstract:
Many biological networks grow under strong spatial constraints, where the large-scale structure emerges from the extension, the branching and intersection of growing parts of the network. One example is provided by ant tunnelling networks, which represent the most common nest architecture in ants. Our goal was to understand how these network structures emerge from the tunnel growth dynamics. We used a standardized two-dimensional set-up shaped as a disk and studied the characteristics of tunnel growth in terms of initiation, propagation and termination of new digging sites and found that they can be described with simple probabilistic laws. We show that a model based on these simple laws and for which parameters were measured from the sand disks experiments can account for the emergence of several topological properties that were observed in experimental networks. In particular, the model accurately reproduced an allometric relation between the number of edges and the number of nodes, as well as an invariance of the node degree distribution. The model was then used to make predictions about the resulting networks' topology when the geometry of the sand substrate was shaped as a square. Experiments aimed at testing the model's predictions showed that the predictions were indeed validated. Both in the model and in the experiments, there was a similar trend for the node degree distribution tail to be steeper in the square sand patch than in the disk sand patch, while other characteristics such as the meshedness (i.e. how densely the network is internally connected) remained constant. Because network growth based on branching/fusion events is widespread in biological systems, this general model might provide useful insights for the study of other systems and, more generally, the evolution of spatial networks in biological systems.
Related Concept Videos
 01:18
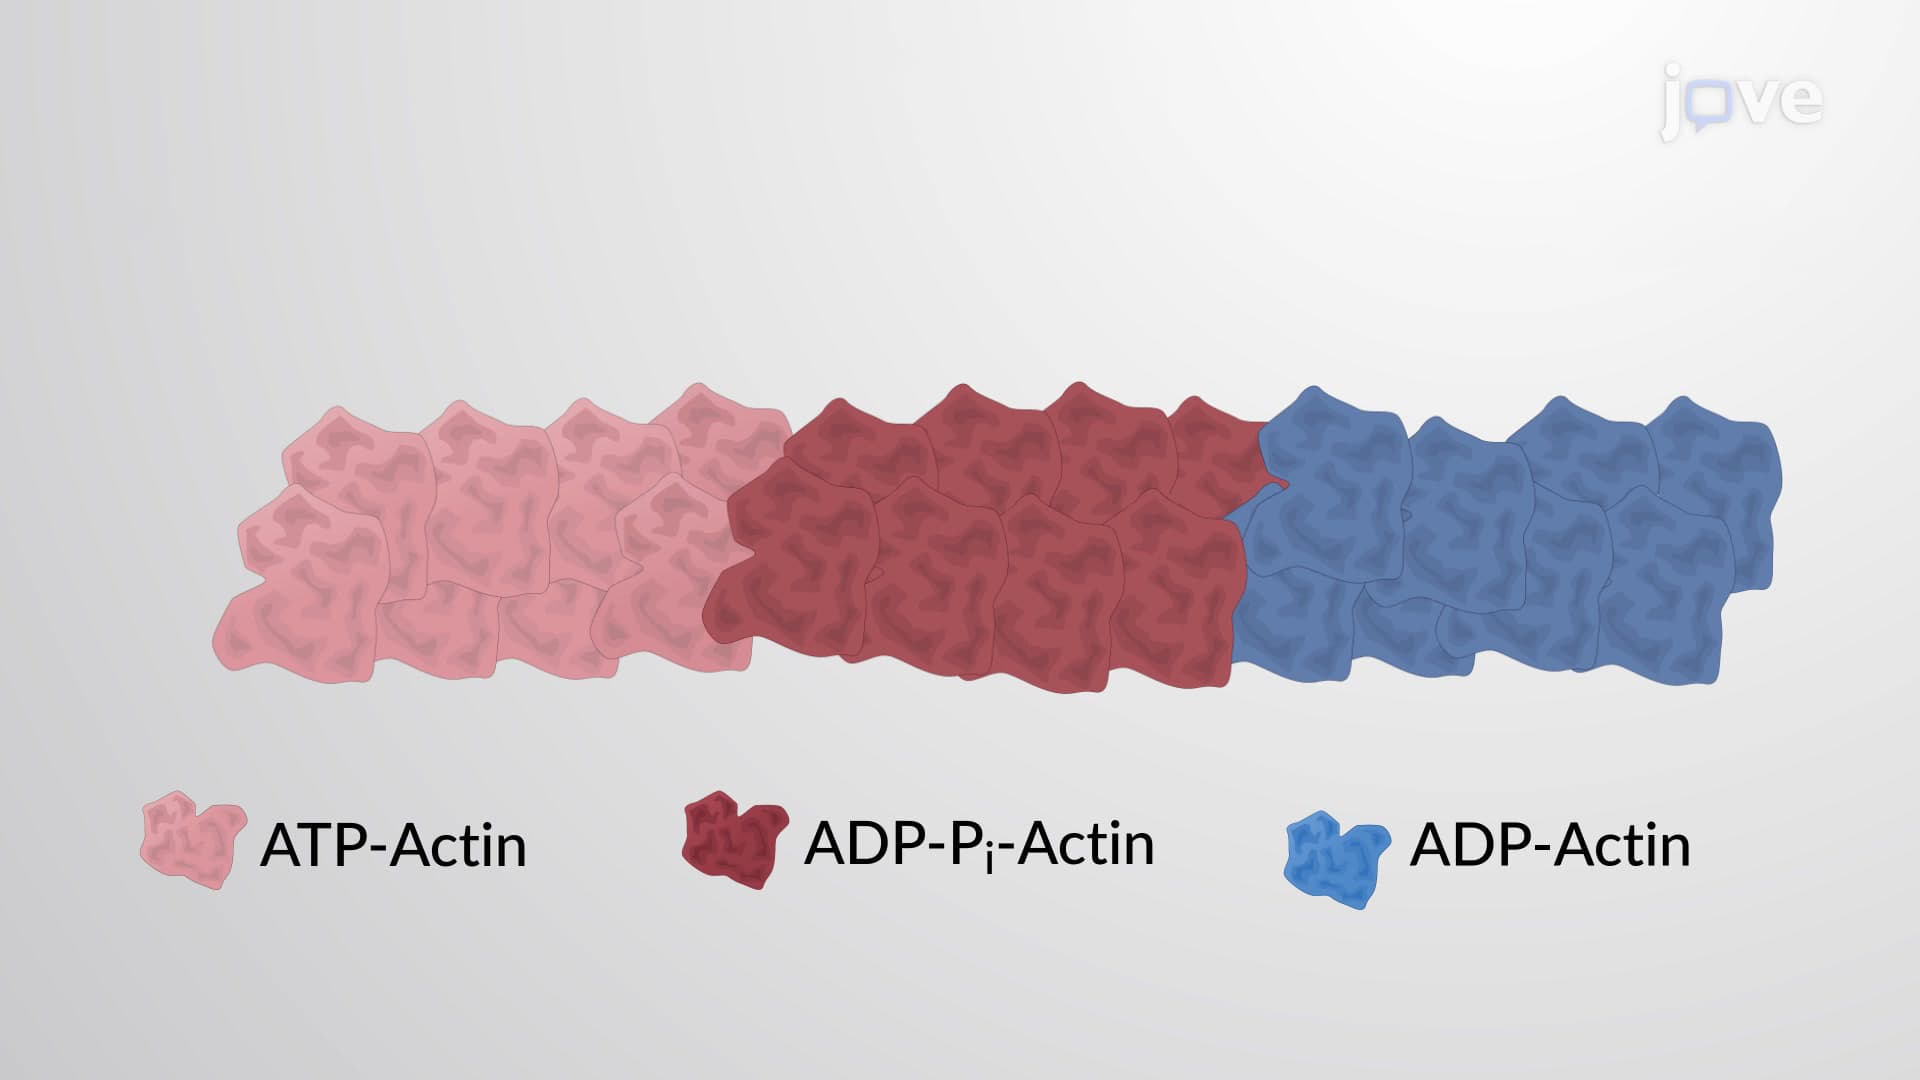
Actin Treadmilling
 01:32
Assembly of Complex Microtubule Structures
 01:11
Formation of Higher-order Actin Filaments
The high-order actin networks...
 01:14
Generation of Straight or Branched Actin Filaments
Arp2/3 Complex
Arp2/3 complex is a seven-subunit complex consisting of two proteins similar to actin- Arp2 and Arp3, and five other subunits that help keep Arp2 and Arp3 inactive. When required, the complex is...
 01:26
Tension Response at Adherens Junctions
α-Catenin as a Mechanosensory Protein
The α-catenin of adherens junctions is an allosteric protein with three VH (vinculin homology) domains...
 01:23
Microtubule Formation