Related Experiment Video
Updated: Jul 16, 2026
Isolation of Translating Ribosomes Containing Peptidyl-tRNAs for Functional and Structural Analyses
Published on: February 25, 2011
Transient arrest in proteasomal degradation during inhibition of translation in the unfolded protein response
Marina Shenkman1, Sandra Tolchinsky, Maria Kondratyev
1Department of Cell Research and Immunology, George Wise Faculty of Life Sciences, Tel Aviv University, Tel Aviv 69978, Israel.

Abstract:
The UPR (unfolded protein response) activates transcription of genes involved in proteasomal degradation. However, we found that in its early stages the UPR leads to a transient inhibition of proteasomal disposal of cytosolic substrates (p53 and p27kip1) and of those targeted to ER (endoplasmic reticulum)-associated degradation (uncleaved precursor of asialoglycoprotein receptor H2a). Degradation resumed soon after the protein synthesis arrest that occurs in early UPR subsided. Consistent with this, protein synthesis inhibitors blocked ubiquitin/proteasomal degradation. Ubiquitination was inhibited during the translation block, suggesting short-lived E3 ubiquitin ligases as candidate depleted proteins. This was indeed the case for p53 whose E3 ligase, Mdm2 (murine double minute 2), when overexpressed, restored the degradation, whereas a mutant Mdm2 in its acidic domain restored the ubiquitination but did not completely restore the degradation. Inhibition of proteasomal degradation early in UPR may prevent depletion of essential short-lived factors during the translation arrest. Stabilization of p27 through this mechanism may explain the cell cycle arrest in G1 when translation is blocked by inhibitors or by the UPR.
Insights
The unfolded protein response (UPR) initially halts proteasomal degradation of key proteins like p53 and p27kip1. This temporary inhibition, linked to protein synthesis arrest, ensures vital factors are not depleted during cellular stress.
Area of Science:
- Cell Biology
- Molecular Biology
- Biochemistry
Background:
- The unfolded protein response (UPR) is a cellular stress response that typically upregulates protein degradation pathways.
- However, the precise impact of early UPR on proteasomal degradation remains incompletely understood.
Purpose of the Study:
- To investigate the early effects of the unfolded protein response (UPR) on the proteasomal degradation of specific cytosolic and ER-associated substrates.
- To elucidate the molecular mechanisms underlying any observed inhibition of proteasomal degradation during early UPR.
Main Methods:
- Utilized cell-based assays to monitor the degradation of p53, p27kip1, and an ER-associated substrate.
- Employed protein synthesis inhibitors and manipulated E3 ligase (Mdm2) expression and function.
- Assessed ubiquitination levels of target proteins.
Main Results:
- Early UPR stages transiently inhibit proteasomal degradation of cytosolic (p53, p27kip1) and ER-associated substrates.
- This inhibition correlates with a block in protein synthesis and is reversible upon recovery from translation arrest.
- Ubiquitination is impaired during the translation block, implicating short-lived E3 ligases like Mdm2.
- Overexpression of functional Mdm2 restored degradation, while a mutant Mdm2 variant partially restored ubiquitination but not full degradation.
Conclusions:
- Early UPR induces a temporary shutdown of proteasomal degradation, likely to conserve essential short-lived proteins during translation arrest.
- The stabilization of p27kip1 may contribute to cell cycle arrest observed under these conditions.
- This finding reveals a novel regulatory mechanism of proteasomal degradation linked to the UPR and protein synthesis.
Related Concept Videos
 01:37
The Unfolded Protein Response
 01:31
Regulation of the Unfolded Protein Response
 01:27
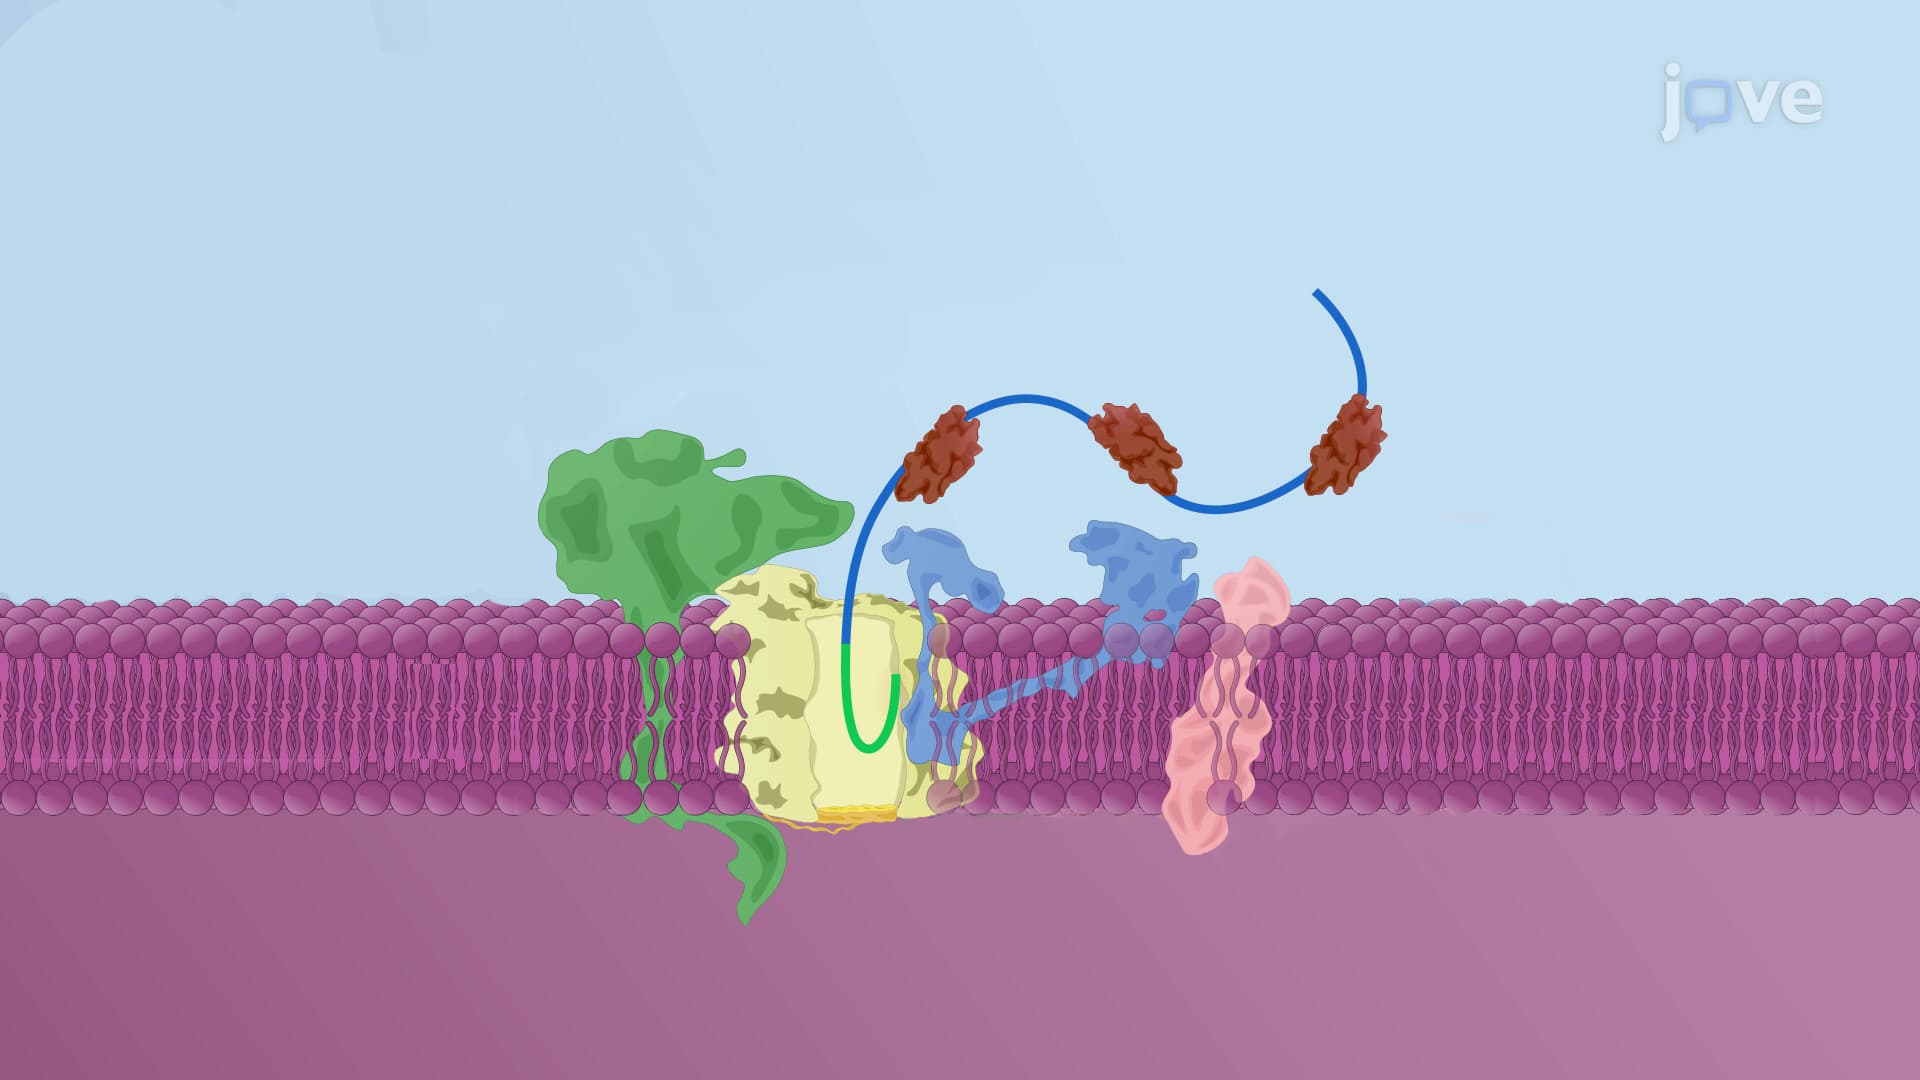
Post-translational Translocation of Proteins to the RER
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
 02:07
Improving Translational Accuracy
 01:20
Cotranslational Protein Translocation
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
 01:13
The Proteasome
In this pathway, the target proteins are first tagged with small proteins called ubiquitin. This involves participation of a series of enzymes including— E1 (ubiquitin-activating enzyme), E2 (ubiquitin-conjugating enzyme), and E3 (ubiquitin...