Related Experiment Video
Updated: Jul 15, 2026

From Constructs to Crystals – Towards Structure Determination of β-barrel Outer Membrane Proteins
Published on: July 4, 2016
Structure and function of transmembrane segment XII in osmosensor and osmoprotectant transporter ProP of Escherichia
Feng Liu1, Doreen E Culham, Yaroslava I Vernikovska
1Department of Structural Biology and Biochemistry, Hospital for Sick Children, Toronto M5G 1X8, ON Canada.

Abstract:
Escherichia coli transporter ProP acts as both an osmosensor and an osmoregulator. As medium osmolality rises, ProP is activated and mediates H+-coupled uptake of osmolytes like proline. A homology model of ProP with 12-transmembrane (TM) helices and cytoplasmic termini was created, and the protein's topology was substantiated experimentally. Residues 468-497, at the end of the C-terminal domain and linked to TM XII, form an intermolecular, homodimeric alpha-helical coiled-coil that tunes the transporter's response to osmolality. We aim to further define the structure and function of ProP residues Q415-E440, predicted to include TM XII. Each residue was replaced with cysteine (Cys) in a histidine-tagged, Cys-less ProP variant (ProP*). Cys at positions 415-418 and 438-440 were most reactive with Oregon Green Maleimide (OGM), suggesting that residues 419 through 437 are in the membrane. Except for V429-I433, reactivity of those Cys varied with helical periodicity. Cys predicted to face the interior of ProP were more reactive than Cys predicted to face the lipid. The former may be exposed to hydrated polar residues in the protein interior, particularly on the periplasmic side. Intermolecular cross-links formed when ProP* variants with Cys at positions 419, 420, 422, and 439 were treated with DTME. Thus TM XII can participate, along its entire length, in the dimer interface of ProP. Cys substitution E440C rendered ProP* inactive. All other variants retained more than 30% of the proline uptake activity of ProP* at high osmolality. Most variants with Cys substitutions in the periplasmic half of TM XII activated at lower osmolalities than ProP*. Variants with Cys substitutions on one face of the cytoplasmic half of TM XII required a higher osmolality to activate. They included elements of a GXXXG motif that are predicted to form the interface of TM XII with TM VII. These studies define the position of ProP TM XII within the membrane, further support the predicted structure of ProP, reveal the dimerization interface, and show that the structure of TM XII influences the osmolality at which ProP activates.
Related Concept Videos
 01:21
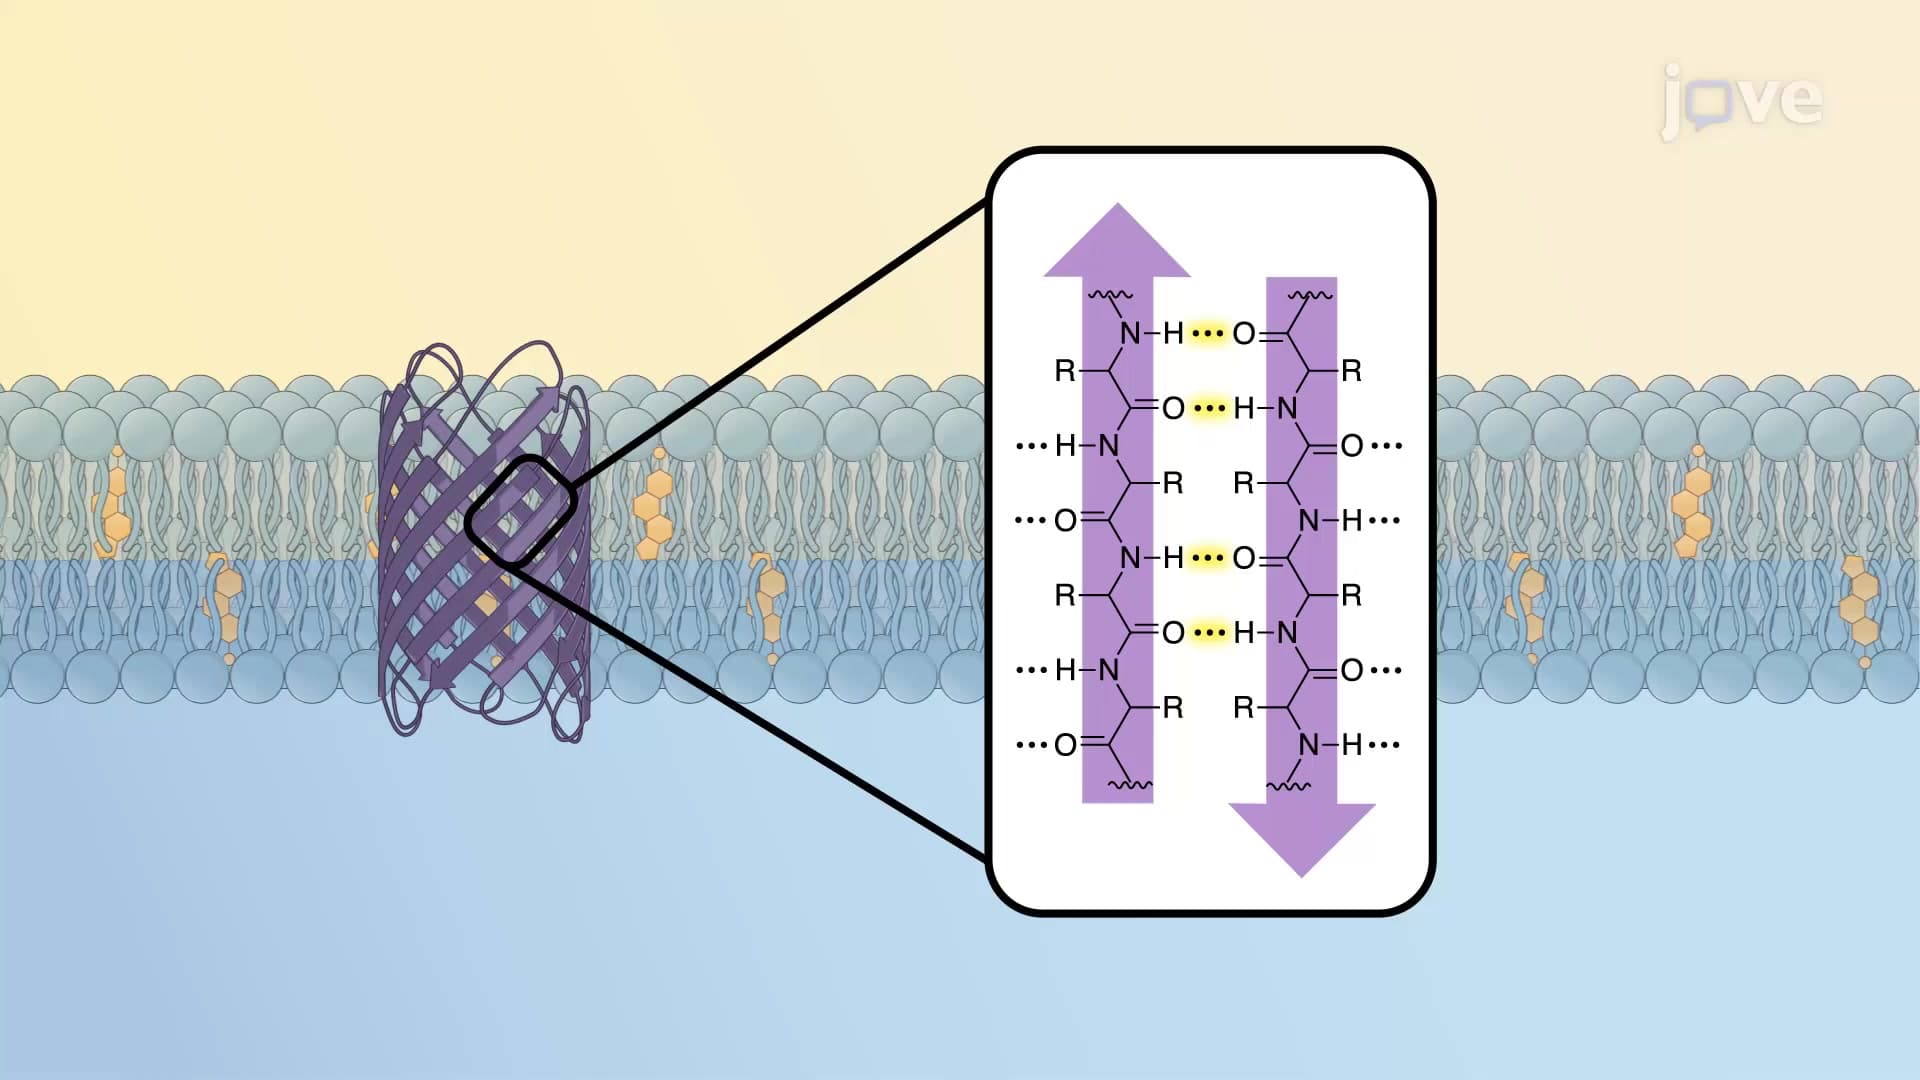
Structure of Porins
 01:09
Multi-pass Transmembrane Proteins and β-barrels
α-Helix containing multi-pass transmembrane proteins
Multi-pass transmembrane proteins such as G-protein-linked receptors (GPCRs) and...
 01:26
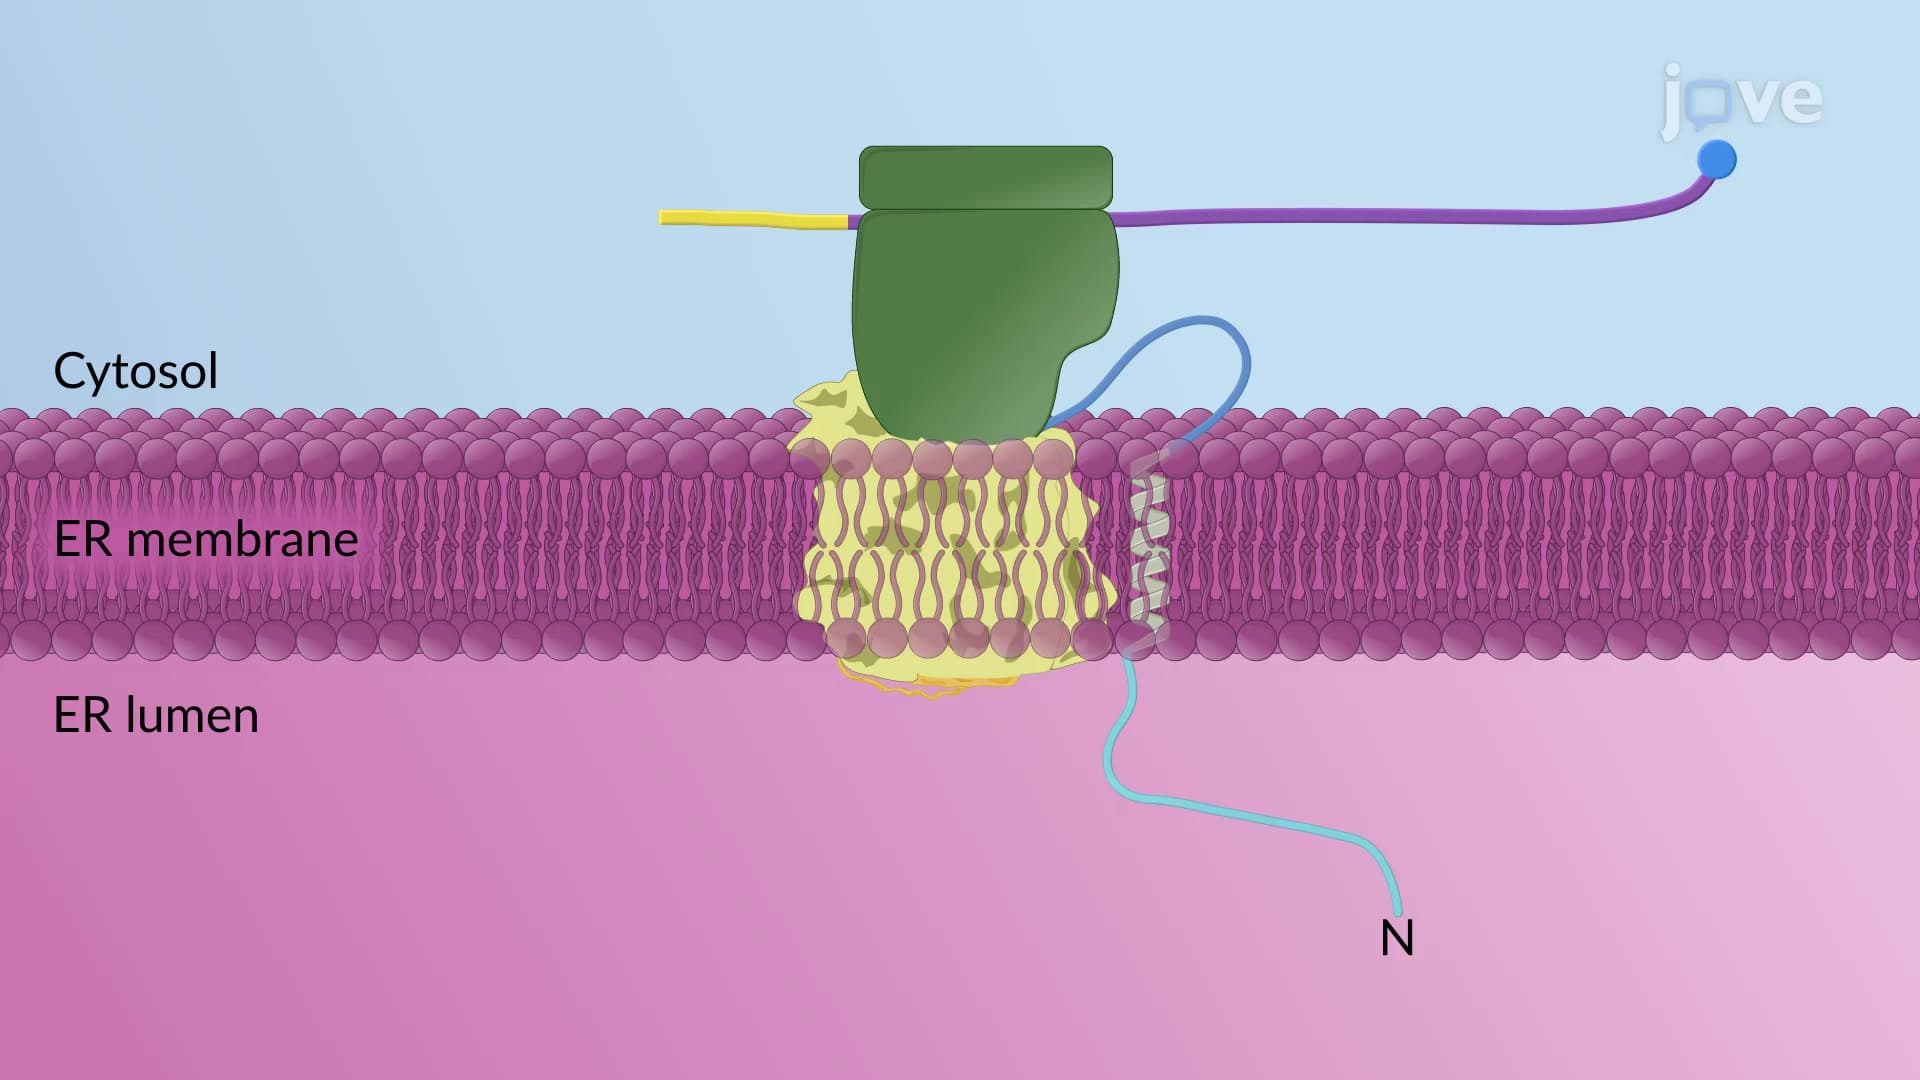
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:29
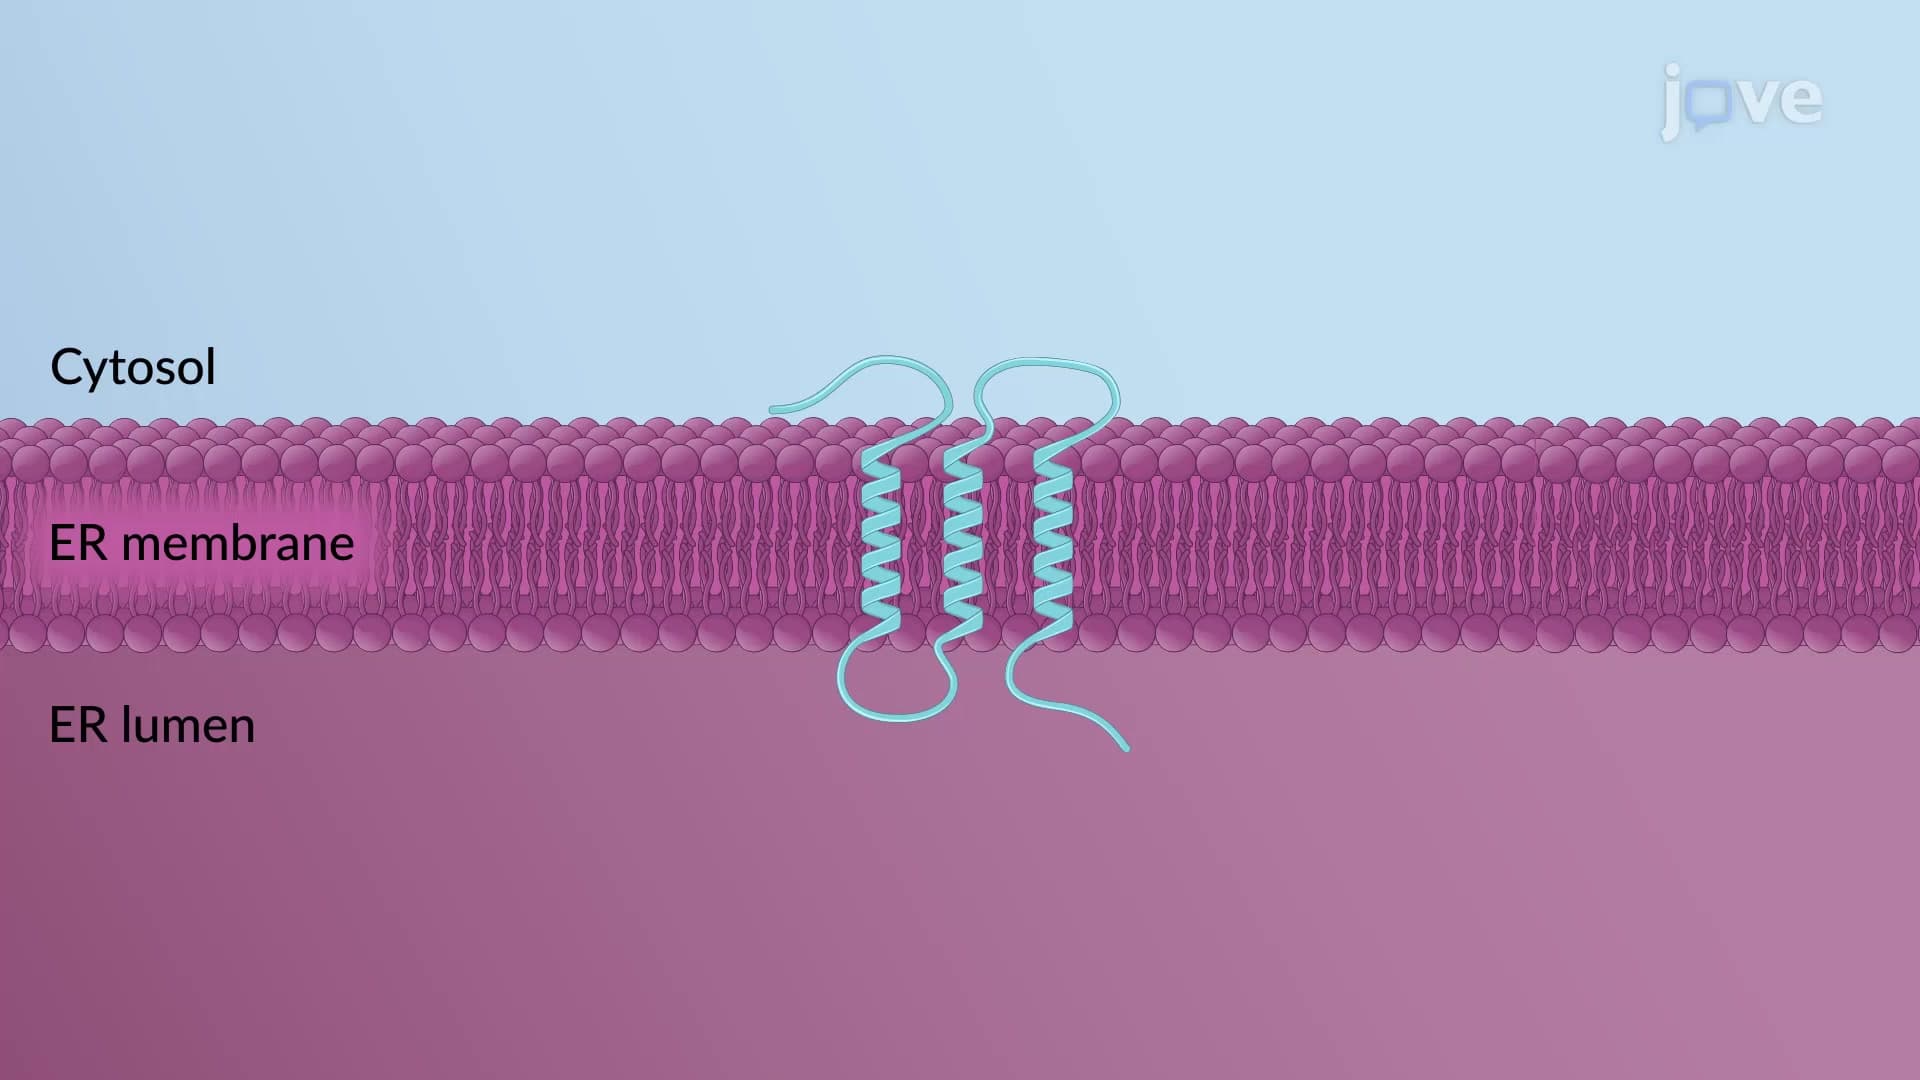
Insertion of Multi-pass Transmembrane Proteins in the RER
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
 01:28
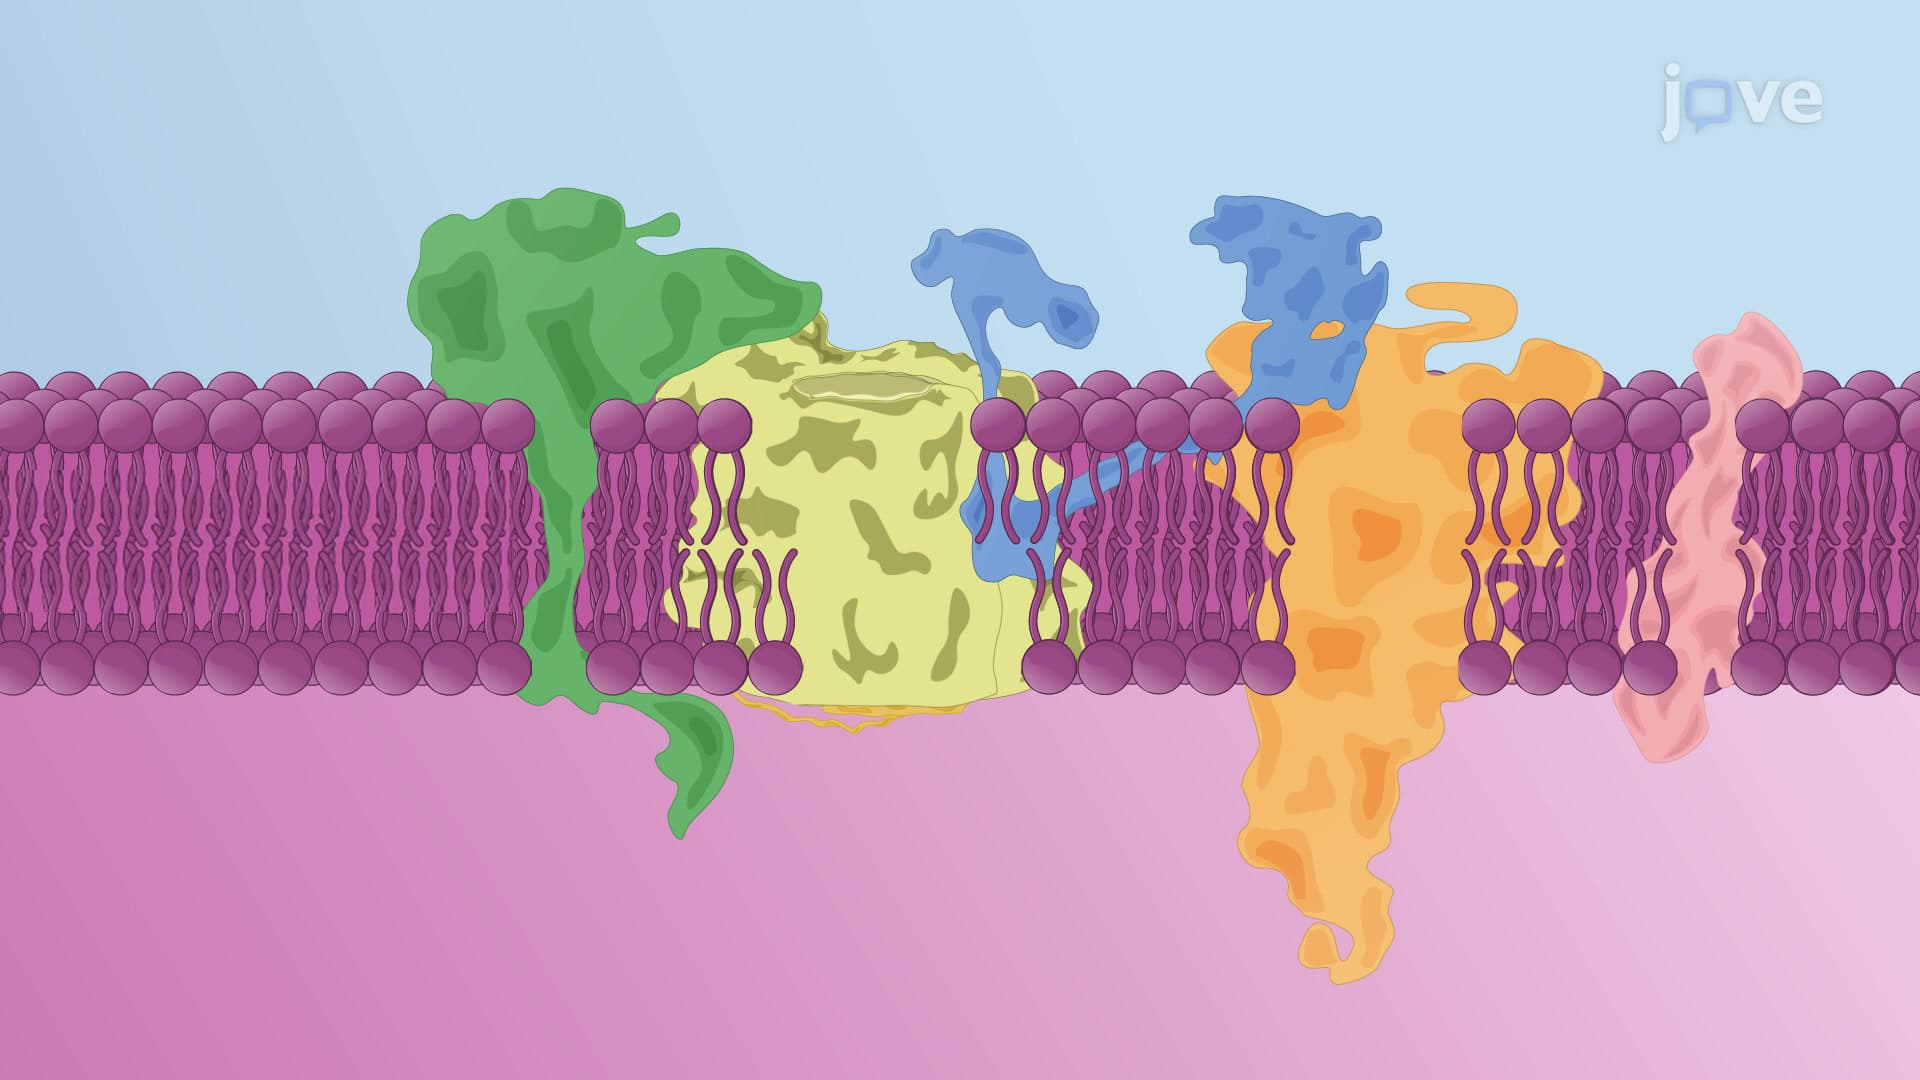
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.
 01:34
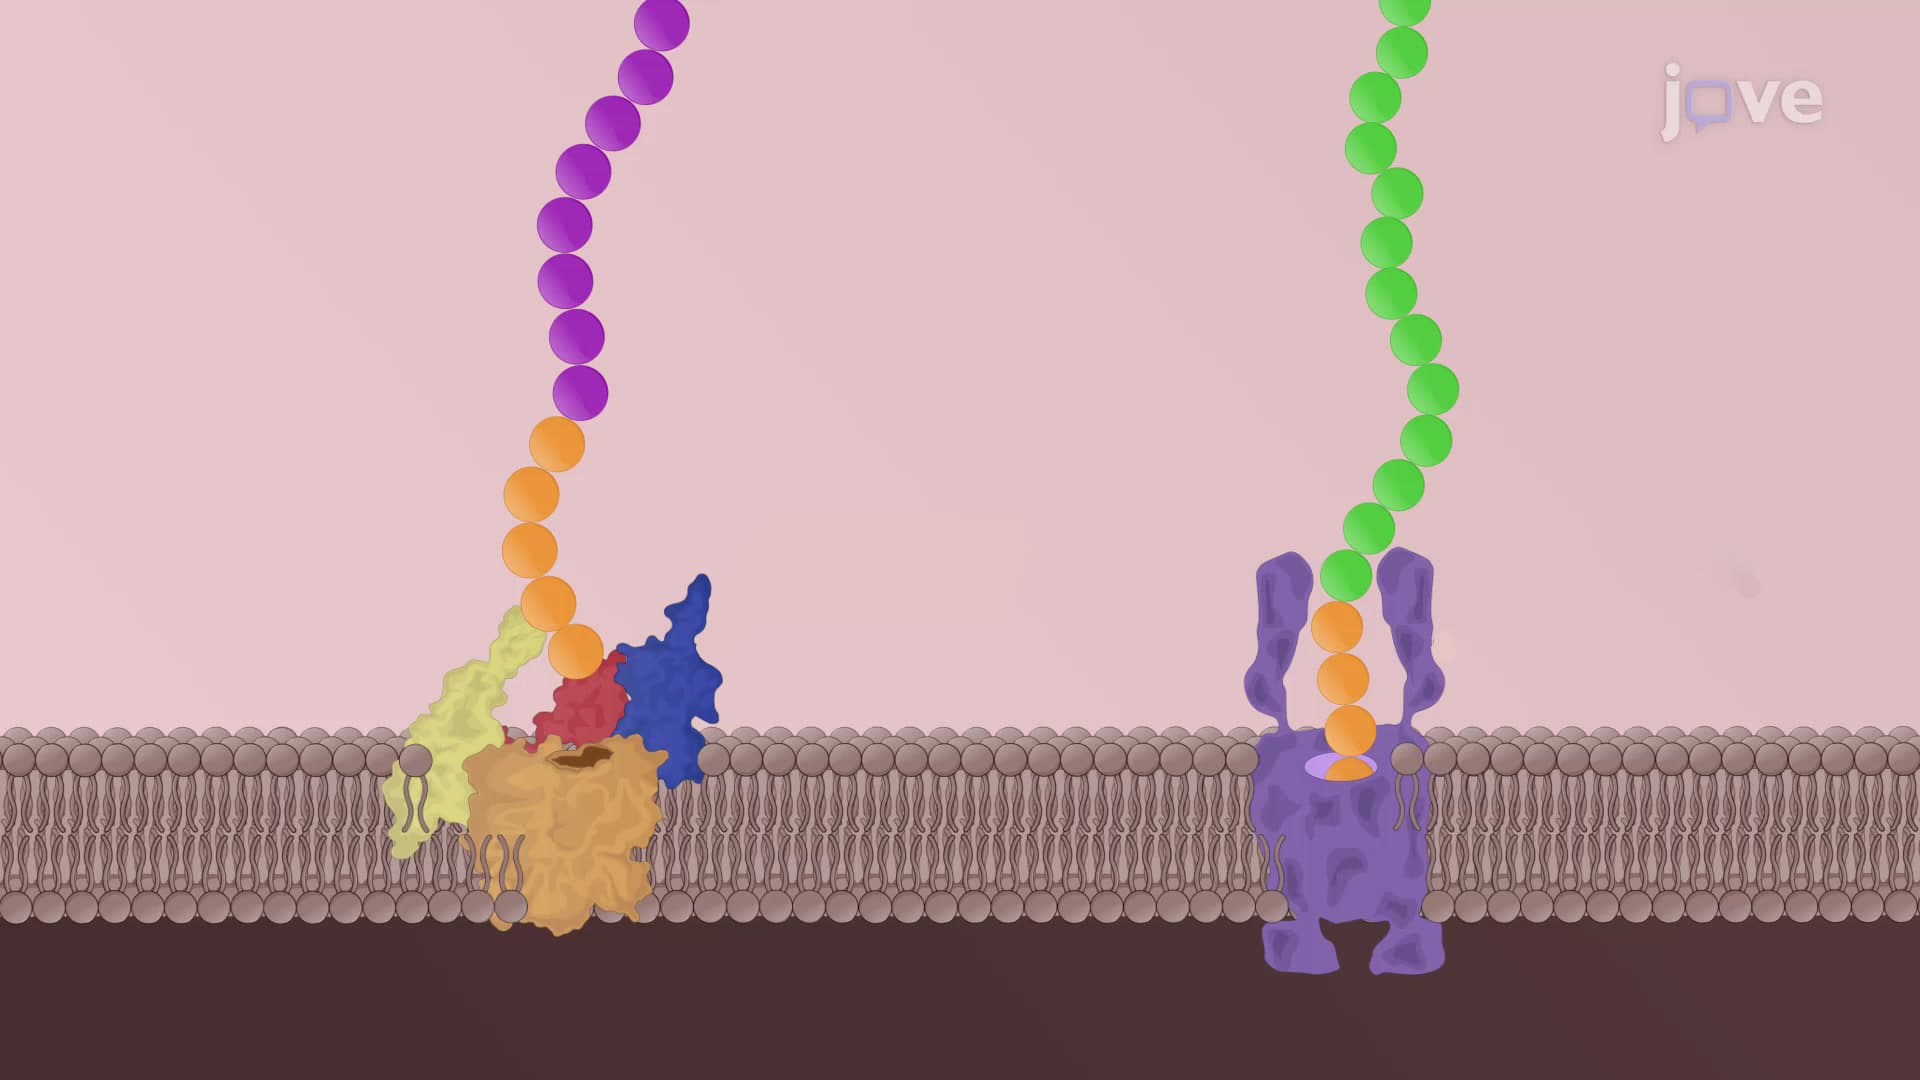
Protein Transport into the Inner Mitochondrial Membrane
Transport of mitochondrial precursors across the TIM23 channel is driven by...