A membrane leucine heptad contributes to trafficking, signaling, and transformation by latent membrane protein 1
Related Experiment Video
Updated: Jul 14, 2026
Image-Based Methods to Study Membrane Trafficking Events in Stomatal Lineage Cells
Published on: May 12, 2023
1McArdle Laboratory for Cancer Research, University of Wisconsin-Madison, Madison, WI 53706, USA.

Abstract:
Latent membrane protein 1 (LMP1) of Epstein Barr virus (EBV) is important for maintaining proliferation of EBV-infected B cells. LMP1, unlike its cellular counterpart, CD40, signals without a ligand and is largely internal to the plasma membrane. In order to understand how LMP1 initiates its ligand-independent signaling, we focused on a leucine heptad in LMP1's first membrane-spanning domain that was shown to be necessary for LMP1's signaling through NF-kappaB. LZ1EBV, a recombinant EBV genetically altered to express LZ1, a derivative of LMP1 in which a leucine heptad was replaced with alanines, transformed B cells with 56% of wild-type (wt) EBV's efficiency, demonstrating the importance of this heptad. To elucidate the mechanism by which this domain contributes to the functions of LMP1, the properties of the wt and LZ1 were compared in transfected cells. LZ1 failed to home to lipid rafts as efficiently as did wt LMP1. The distribution of tagged derivatives of LZ1 also differed from that of wt LMP1 in transfected cells. LZ1's defect in homing to lipid rafts and altered trafficking likely underlie the defect in transformation of LZ1EBV. While the third and fourth membrane-spanning domains of LMP1 foster its trafficking to the Golgi, the leucine heptad within the first membrane-spanning domain contributes to its trafficking, particularly to internal rafts. B cells that are successfully transformed by LZ1EBV have the same average number of viral genomes and the same fraction of cells with capped LZ1 at the cell surface but express 50% more of the LZ1 allele than wt infected cells.
Related Concept Videos
 01:17
Intracellular Signaling Affects Focal Adhesions
Some...
 01:26
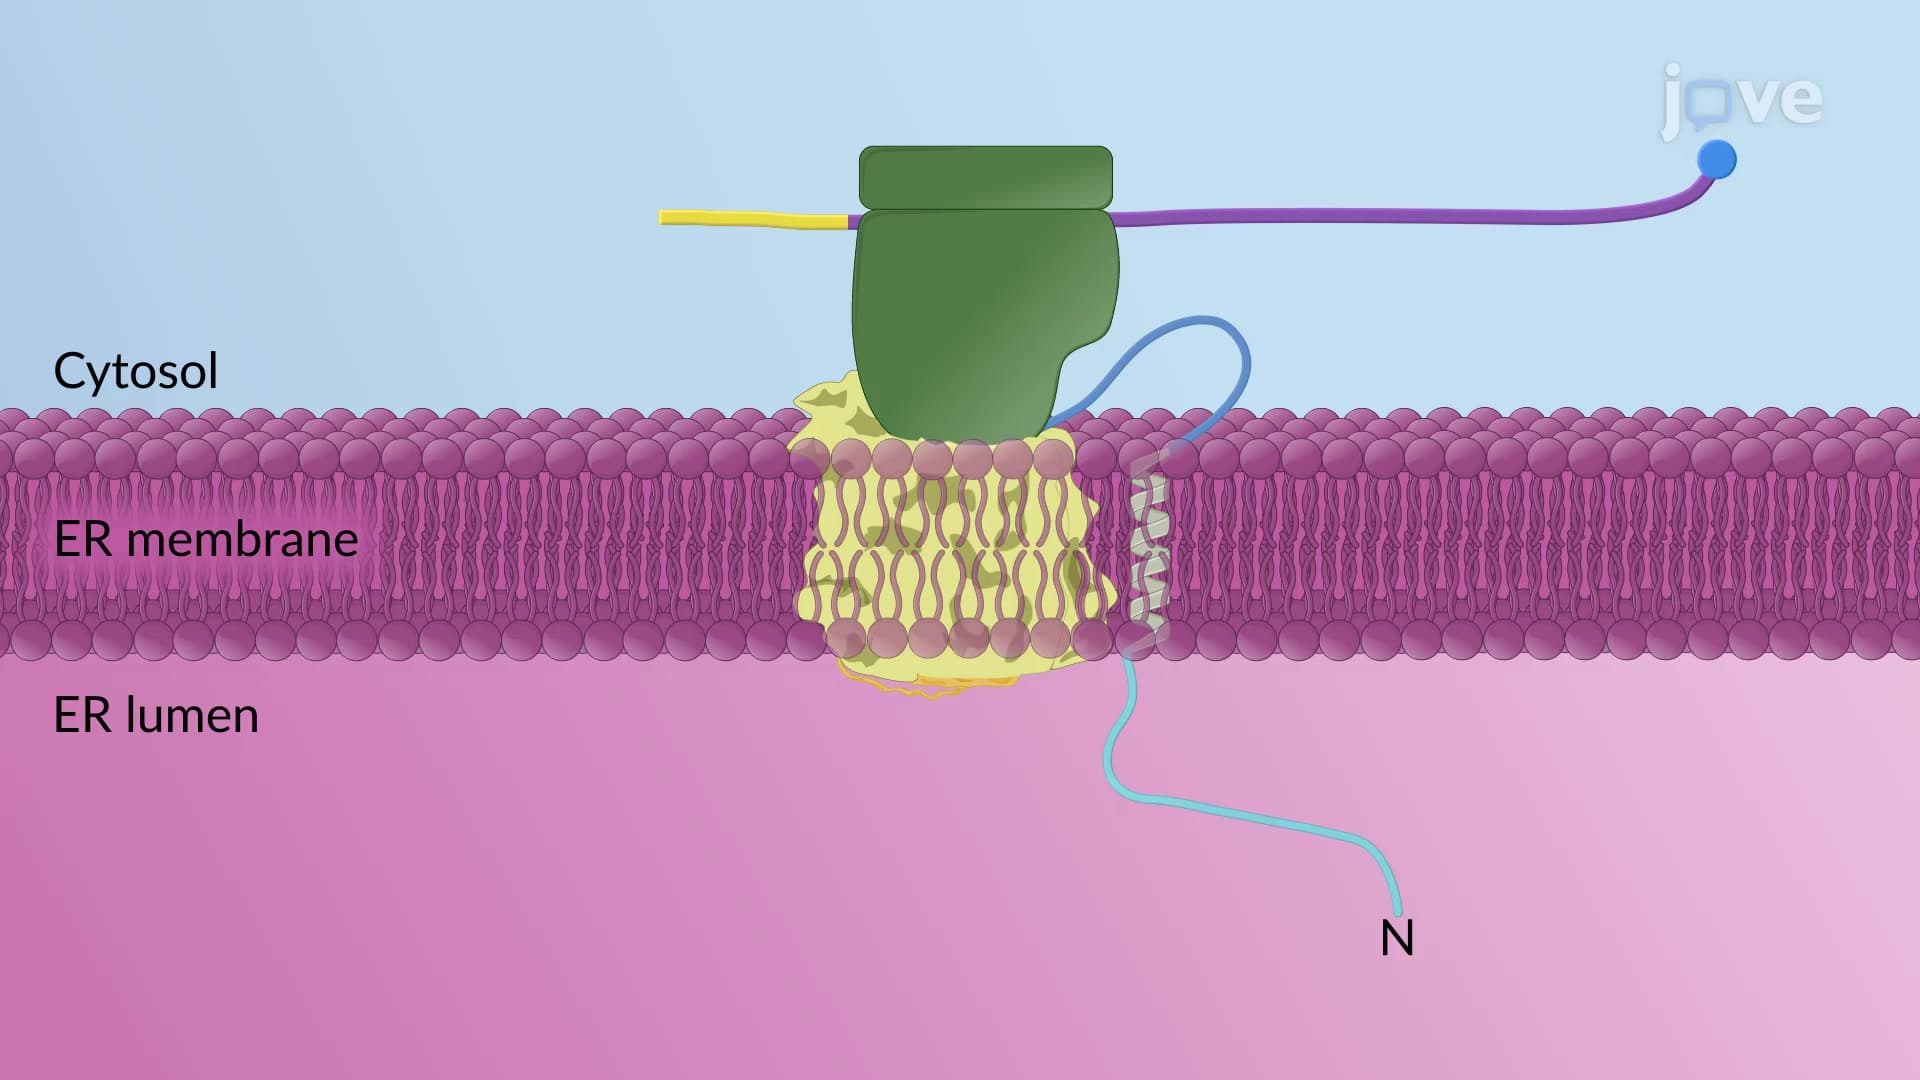
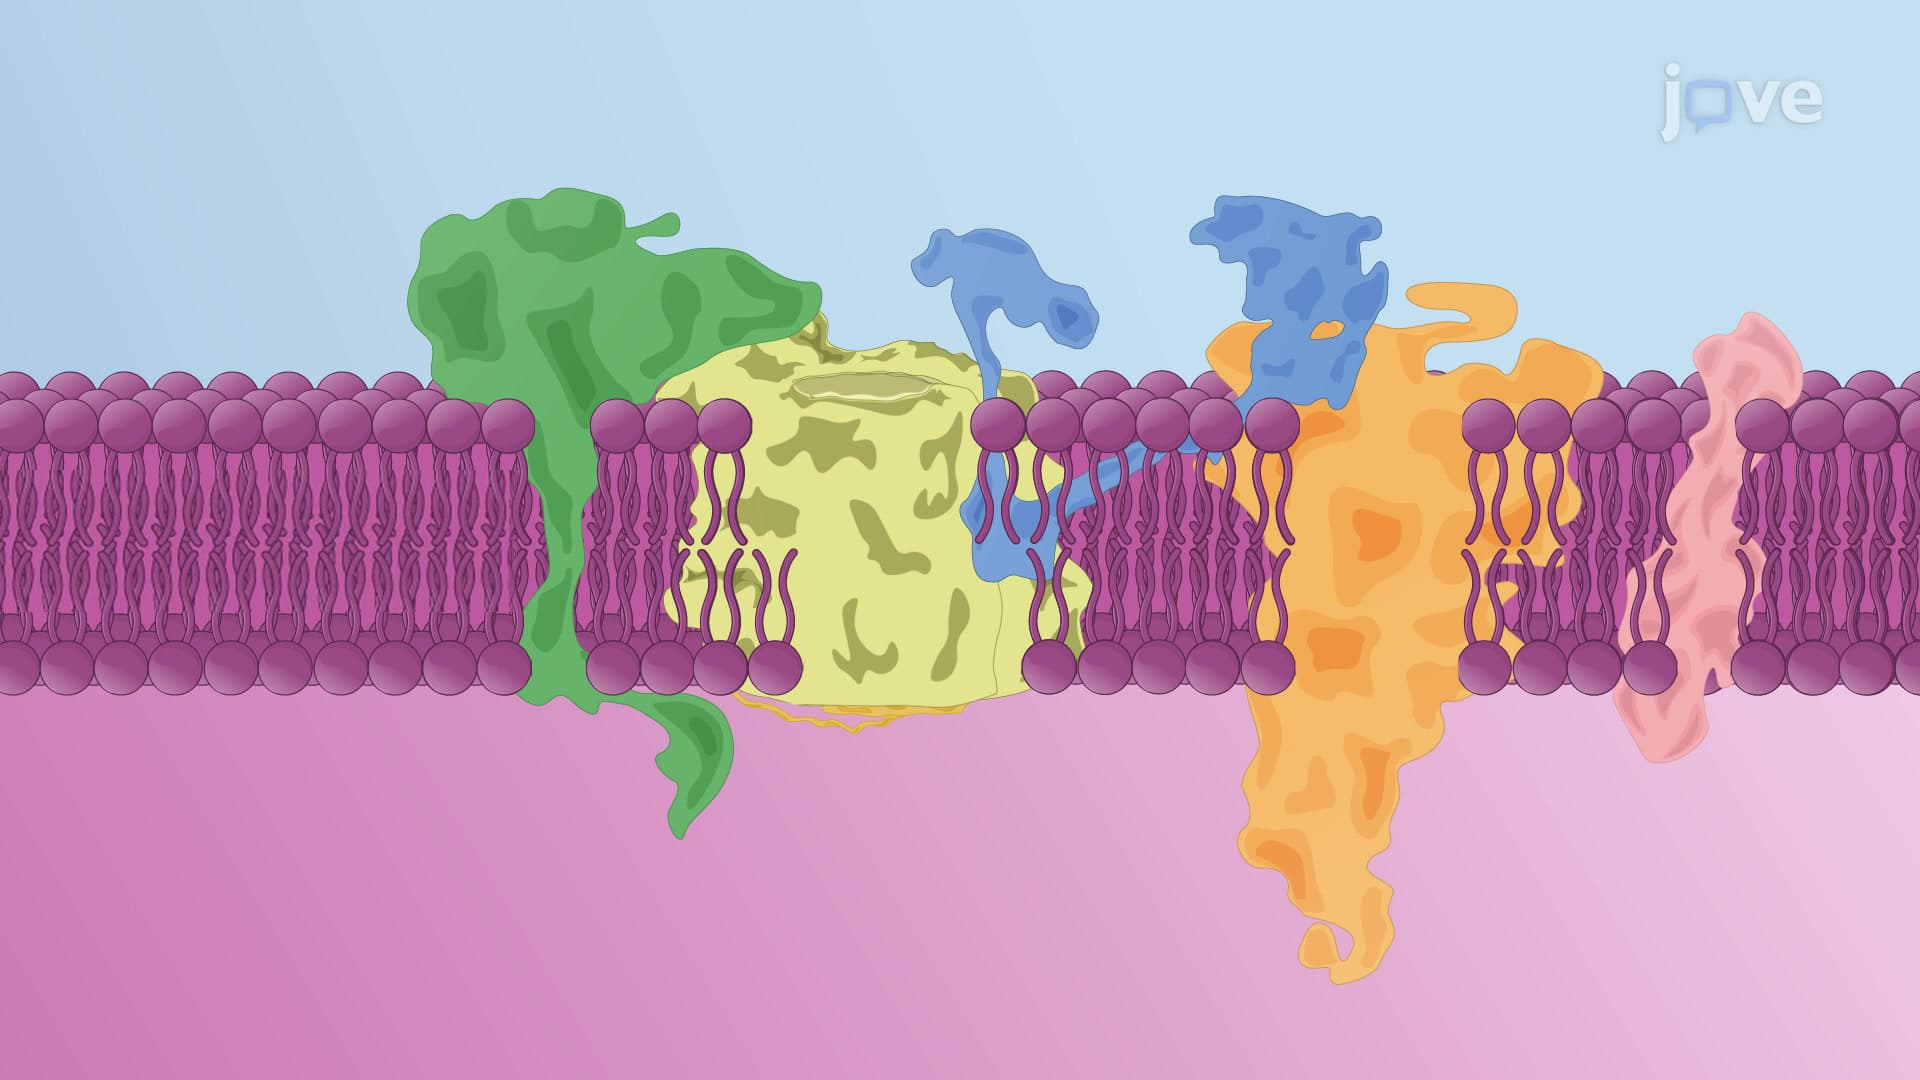
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:28
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.
 01:20
Cotranslational Protein Translocation
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
 01:19
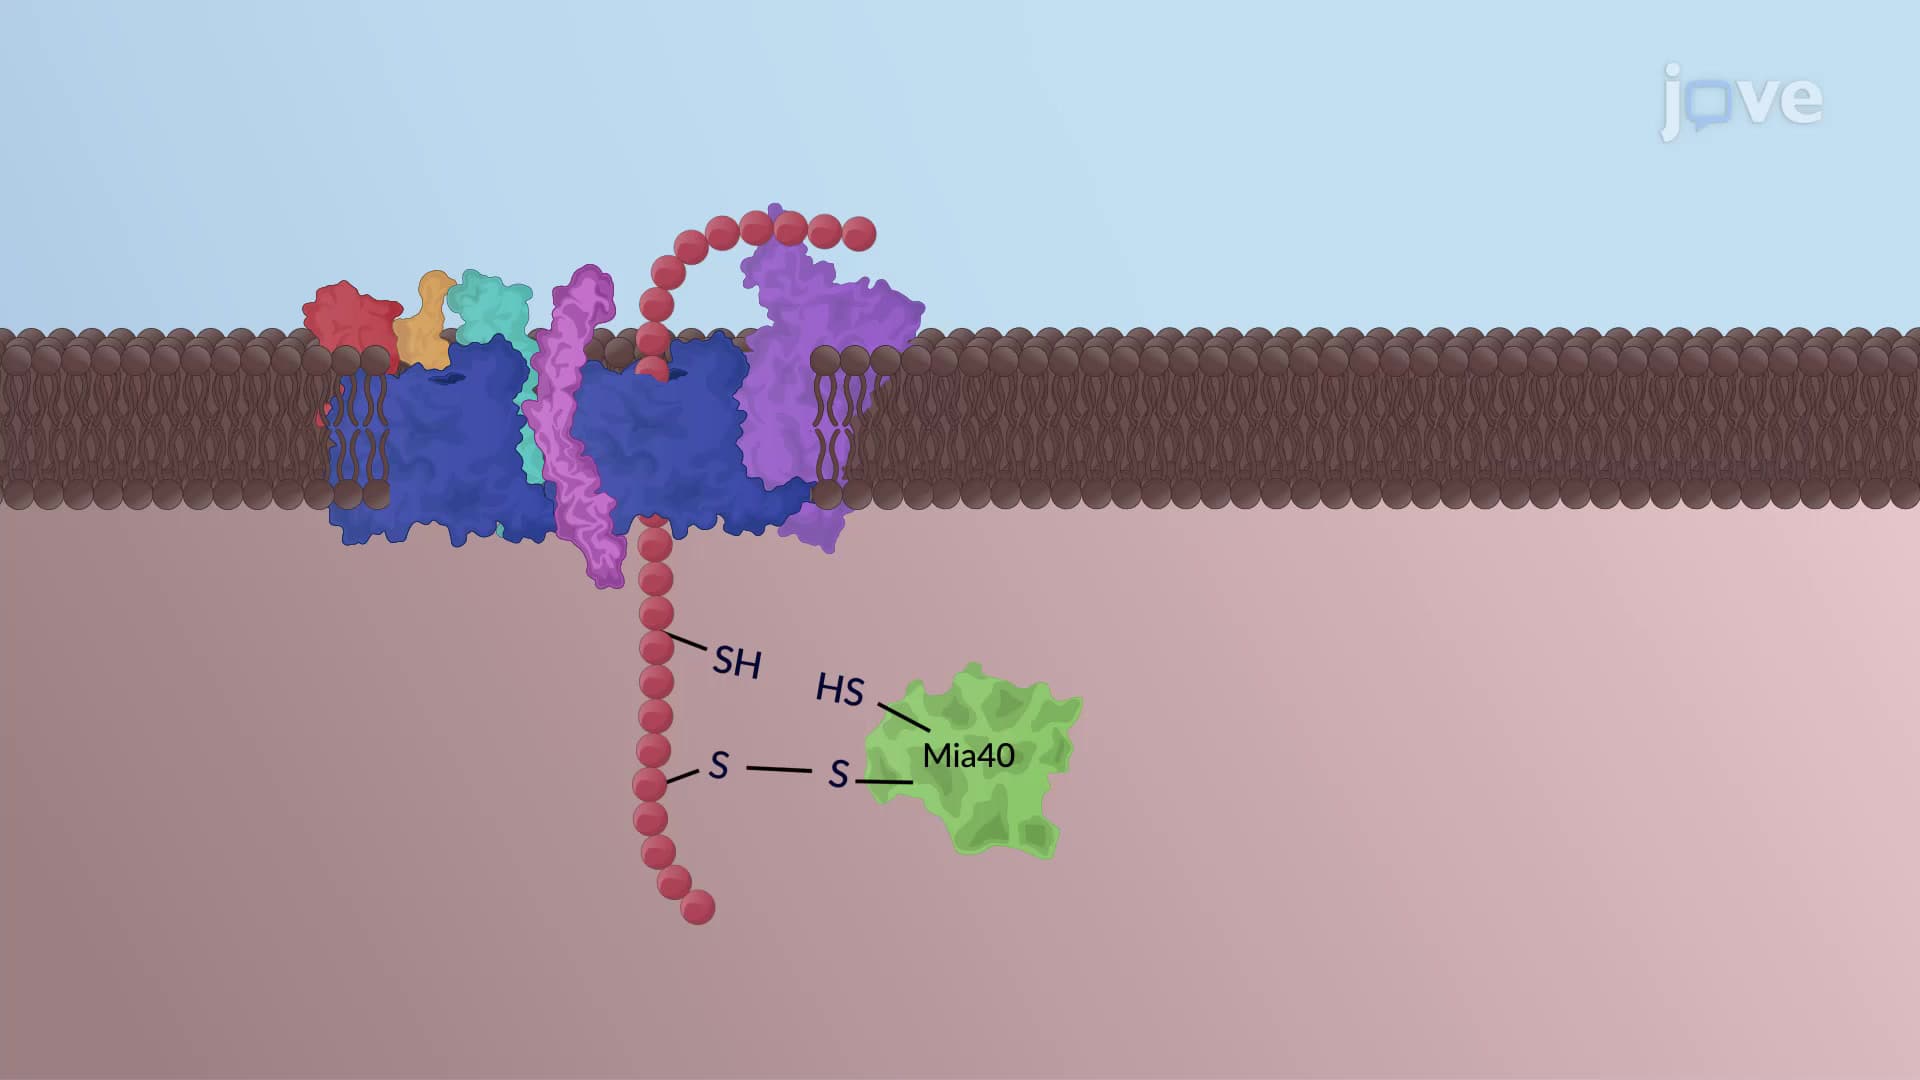
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:14
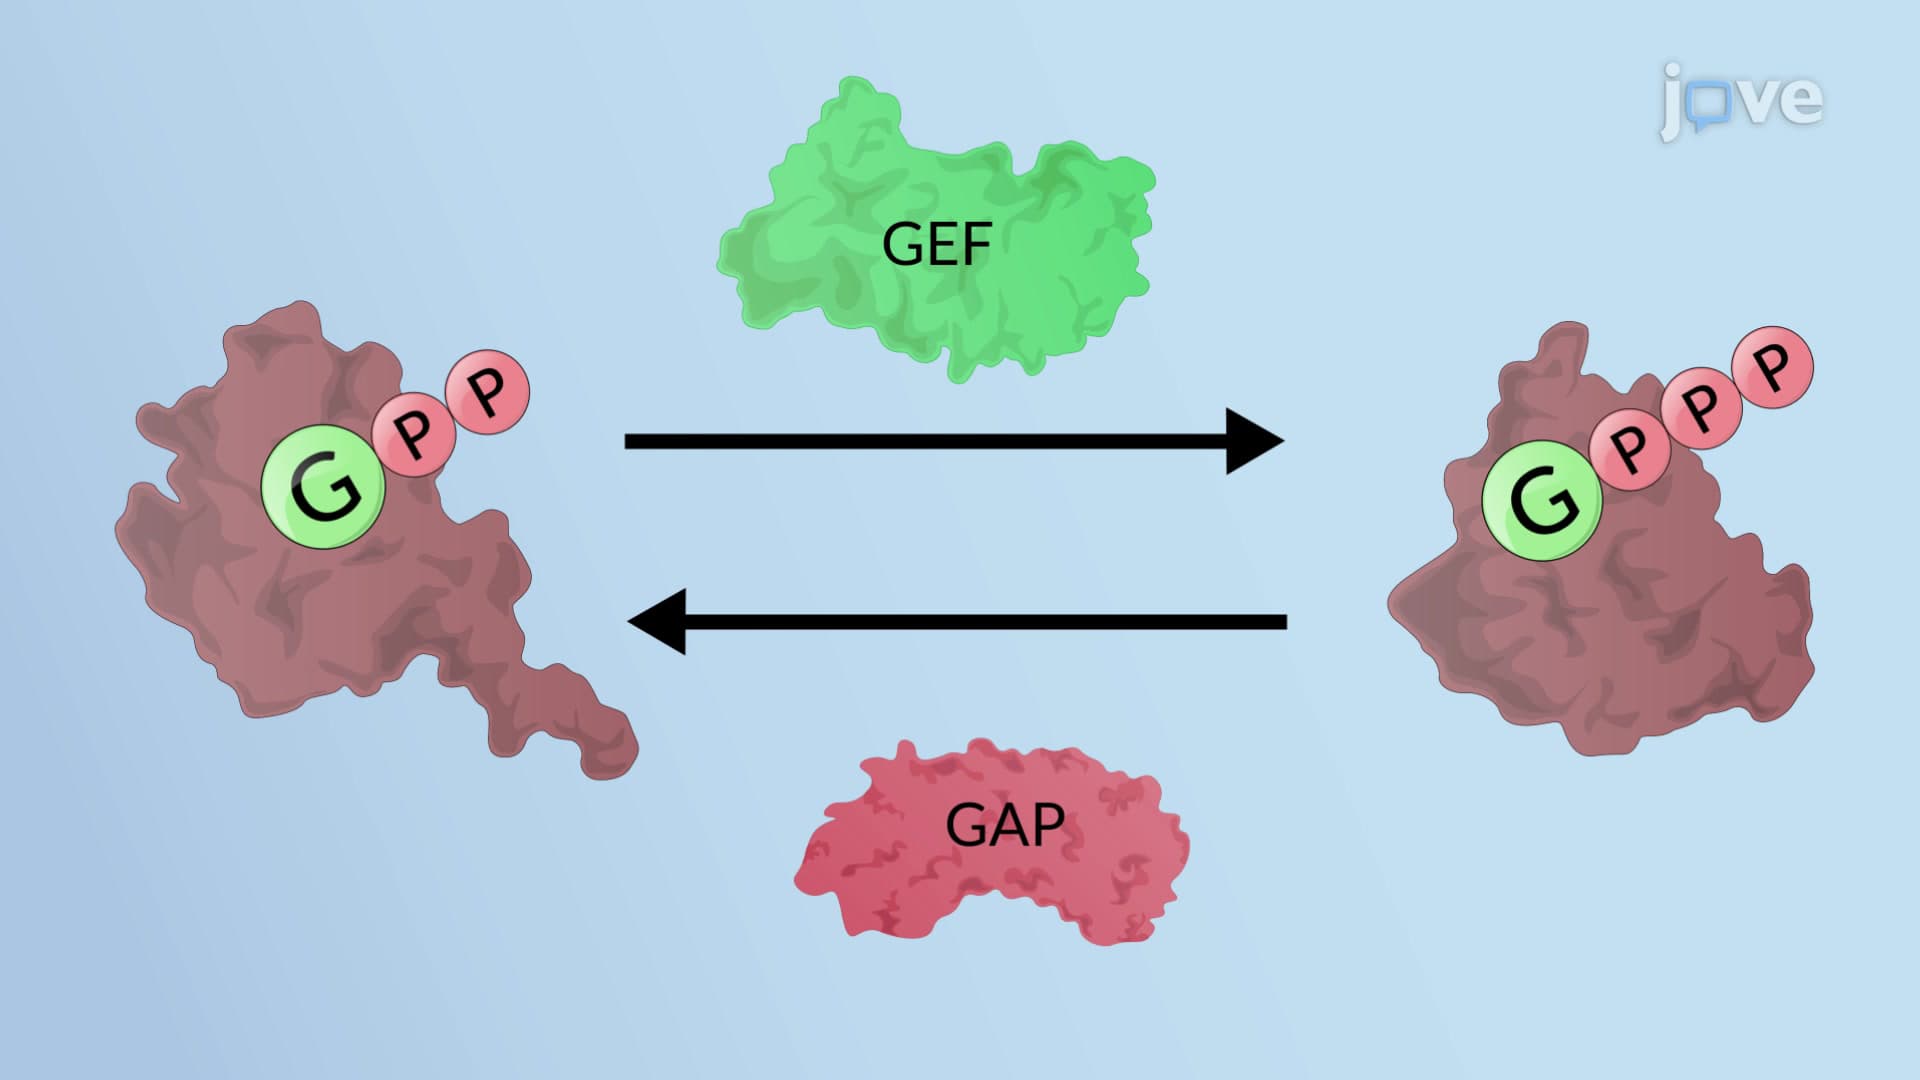
Rab Proteins
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...