Related Experiment Video
Updated: Jul 10, 2026
Monitoring the Assembly of a Secreted Bacterial Virulence Factor Using Site-specific Crosslinking
Published on: December 17, 2013
A conserved alpha helical domain at the N-terminus of Pex14p is required for PTS1 and PTS2 protein import in
Bart de Vries1, Jan A K W Kiel, Ruud Scheek
1Molecular Cell Biology, Groningen Biomolecular Sciences and Biotechnology Institute (GBB), University of Groningen, 9750 AA, Haren, The Netherlands.

Abstract:
We have analyzed the highly conserved N-terminus of Hansenula polymorpha Pex14p for its function in peroxisomal matrix protein import. The region comprising aa 10-54 of HpPex14p is predicted to contain three alpha-helices. Its alpha-helical structure was confirmed by CD analysis of a synthetic peptide, corresponding to residues 8-58. Deletion of aa 1-21 of HpPex14p, but not of aa 1-9, completely abolished PTS1 and PTS2 matrix protein import. An extensive mutational analysis of the first alpha-helix (aa 10-21) demonstrated that its secondary structure, as well as residues Phe20 and Leu21, are essential for PTS1 and PTS2 matrix protein import.
More Related Videos
Related Concept Videos
 01:27
Protein Import into the Peroxisomes
Peroxisomal Protein Import:
Peroxisomes lack the genetic machinery required to code for their own proteins. Hence, most peroxisomal membrane, lumenal and transmembrane proteins are synthesized in the cytoplasm or ER and transported to the peroxisome...
 01:21
Structure of Porins
 01:20
Cotranslational Protein Translocation
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
 01:19
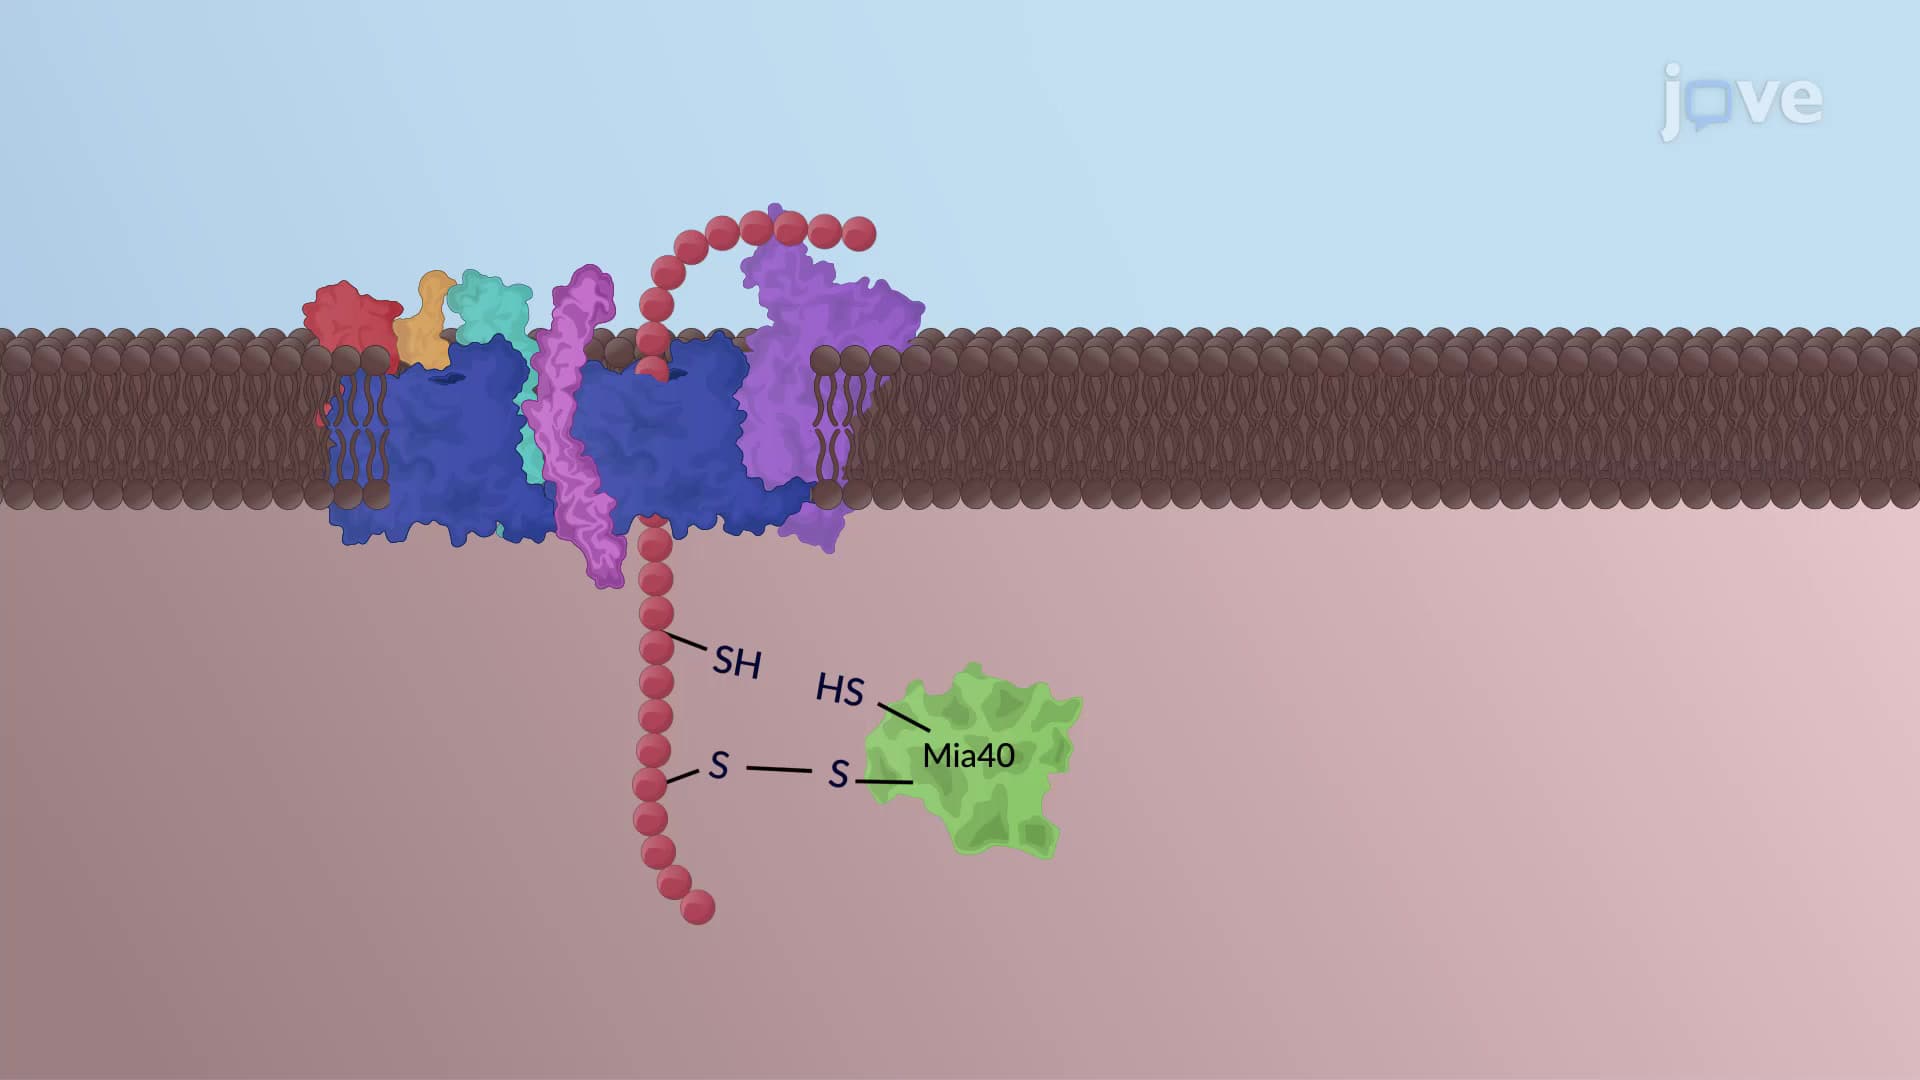
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:45
Tail-anchoring of Proteins in the ER Membrane
 01:46
Nuclear Localization Signals and Import