Related Experiment Video
Updated: Jul 9, 2026
Transmembrane Domain Oligomerization Propensity determined by ToxR Assay
Published on: May 26, 2011
Oligomerization of membrane-bound diphtheria toxin (CRM197) facilitates a transition to the open form and deep
1Sandia National Laboratories, Albuquerque, New Mexico, USA. mskent@sandia.gov

Abstract:
Diphtheria toxin (DT) contains separate domains for receptor-specific binding, translocation, and enzymatic activity. After binding to cells, DT is taken up into endosome-like acidic compartments where the translocation domain inserts into the endosomal membrane and releases the catalytic domain into the cytosol. The process by which the catalytic domain is translocated across the endosomal membrane is known to involve pH-induced conformational changes; however, the molecular mechanisms are not yet understood, in large part due to the challenge of probing the conformation of the membrane-bound protein. In this work neutron reflection provided detailed conformational information for membrane-bound DT (CRM197) in situ. The data revealed that the bound toxin oligomerizes with increasing DT concentration and that the oligomeric form (and only the oligomeric form) undergoes a large extension into solution with decreasing pH that coincides with deep insertion of residues into the membrane. We interpret the large extension as a transition to the open form. These results thus indicate that as a function of bulk DT concentration, adsorbed DT passes from an inactive state with a monomeric dimension normal to the plane of the membrane to an active state with a dimeric dimension normal to the plane of the membrane.
Related Concept Videos
 01:26
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:28
Diphtheria
 01:29
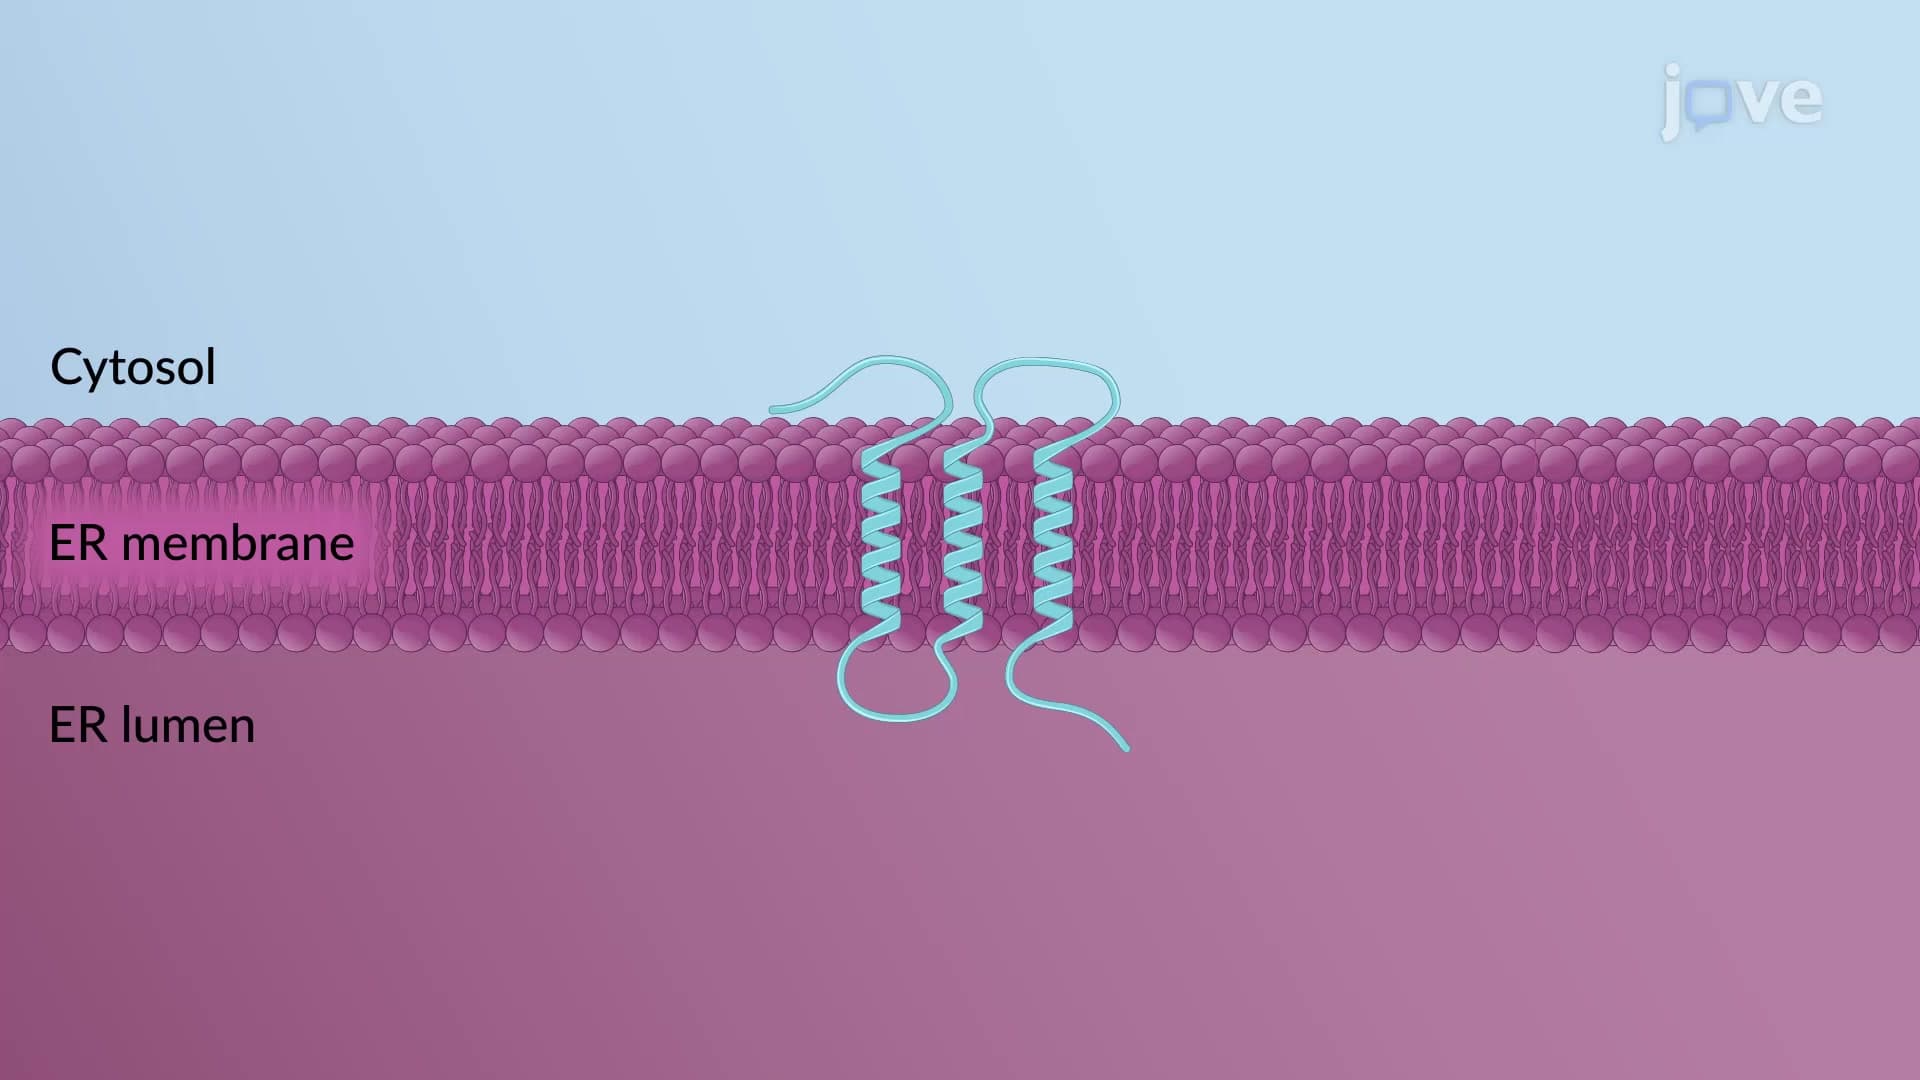
Insertion of Multi-pass Transmembrane Proteins in the RER
The multipass transmembrane proteins are the type IV integral membrane proteins with multiple topogenic sequences determining their spatial arrangement in the ER membrane. Nearly all multipass proteins lack a cleavable signal sequence and use...
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
 01:28
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.