Related Experiment Video
Updated: Jul 7, 2026

Cycloheximide Chase Analysis of Protein Degradation in Saccharomyces cerevisiae
Published on: April 18, 2016
Endoplasmic reticulum-associated degradation of mutant CFTR requires a guanine nucleotide-sensitive step
Béatrice De Keukeleire1, Julien Micoud, Julie Biard
1CNRS, UMR 5249, 17 Rue des Martyrs, Grenoble F-38054, France.

Abstract:
Proteasome degradation of endoplasmic reticulum (ER)-misfolded proteins requires retrograde transport from ER to the cytosol. To date, it is not clear whether this event constitutes the exclusive ER degradation process for non-native membrane proteins. Here we describe the role of GTP in the degradation of DeltaF508-CFTR and the alpha subunit of the T-cell receptor (TCRalpha), representative misfolded ER membrane proteins. Selective intracellular GTP depletion extended the DeltaF508-CFTR half-life sixfold, whereas ATP depletion accelerated its turnover and inhibited only 80% of the proteasome activity that was not affected by GTP depletion. AlF(4)(-), a well-known inhibitor of heterotrimeric G proteins, but not of AlF(3), delayed the mutant CFTR turnover in vivo, in semi-intact cells and in ER-enriched microsomes, without affecting ER to Golgi cargo transport. DeltaF508-CFTR degradation was also inhibited by alkaline stripping of ER-associated membrane proteins. We propose that at the ER, GTP may participate in the disposal of misfolded membrane proteins through activation of heterotrimeric G proteins.
More Related Videos
Related Concept Videos
 01:32
Export of Misfolded Proteins out of the ER
 01:12
GPCR Desensitization
 01:25
Rab Cascades
 01:37
The Unfolded Protein Response
 01:14
Rab Proteins
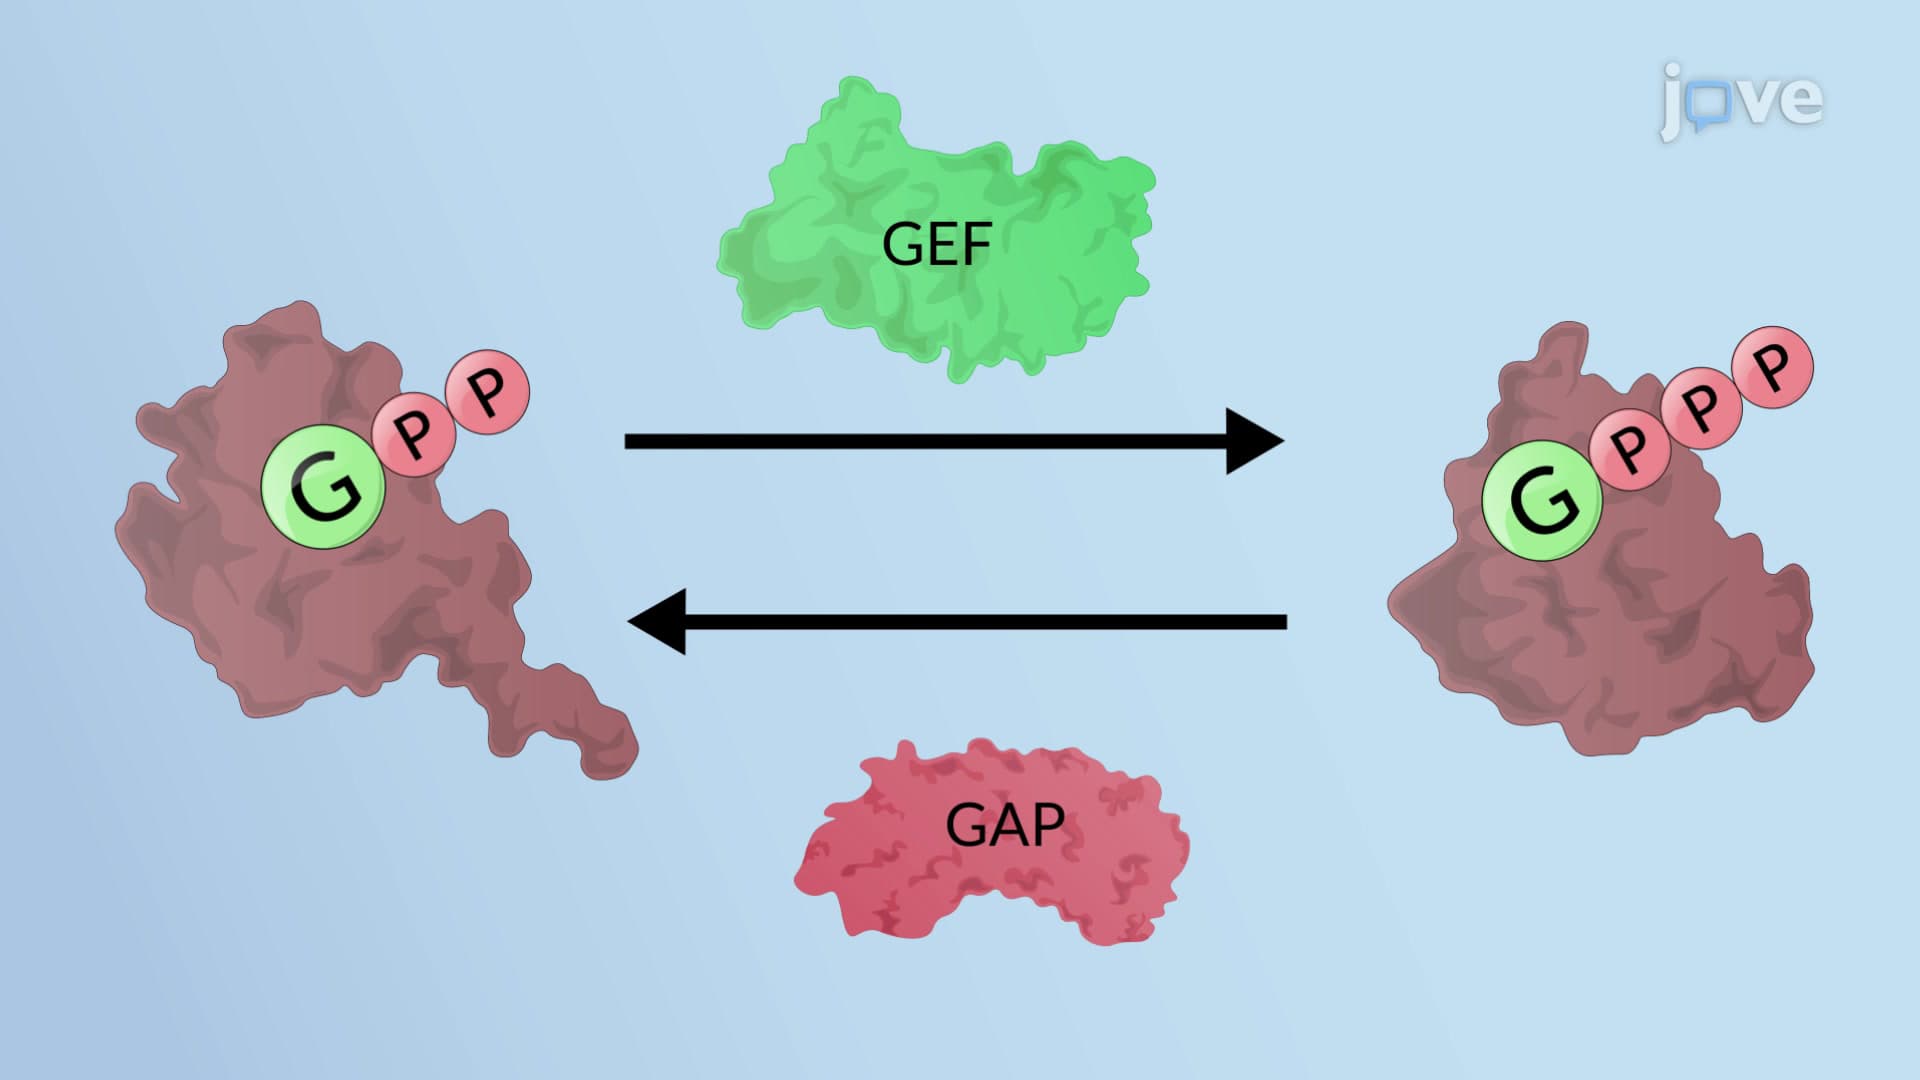
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...
 01:29
Protein Folding Quality Check in the RER