A calmodulin-activated (Ca(2+)-Mg2+)-ATPase is involved in Ca2+ transport by plasma membrane vesicles from
G Benaim1, S Losada, F R Gadelha
1Department of Veterinary Pathobiology, University of Illinois, Urbana 61801.

Abstract:
High-affinity Ca(2+)-activated ATPases that do not show any demonstrable dependence on Mg2+ have been reported in the plasma membranes of different trypanosomatids, and it has been suggested [McLaughlin (1985) Mol. Biochem. Parasitol. 15, 189-201; Ghosh, Ray, Sarkar & Bhaduri (1990) J. Biol. Chem. 265, 11345-11351] that these enzymes may have a role in Ca2+ transport by the plasma membrane and in the regulation of intracellular Ca2+ in these parasites. In this report we investigated Ca2+ transport by Trypanosoma cruzi plasma membrane vesicles using Arsenazo III as a Ca2+ indicator. These vesicles accumulated Ca2+ upon addition of ATP only when Mg2+ was present and released it in response to the Ca2+ ionophore A23187, but were insensitive to inositol 1,4,5-trisphosphate. Ca2+ transport was insensitive to antimycin A, oligomycin and carbonyl cyanide p-trifluorophenylhydrazone, ruling out any mitochondrial contamination. Staurosporine and phorbol myristate acetate had no effect on this activity, while low concentrations of vanadate (10 microM) completely inhibited it. In addition, we describe a high-affinity vanadate-sensitive (Ca(2+)-Mg2+)-ATPase in the highly enriched plasma membrane fraction of T. cruzi. Kinetic studies indicated that the apparent Km for free Ca2+ was 0.3 microM. On the other hand, Ca(2+)-ATPase activity and Ca2+ transport were both stimulated by bovine brain calmodulin and by endogenous calmodulin purified from these cells. In addition, trifluoperazine and calmidazolium, at concentrations in the range in which they normally exert anti-calmodulin effects, inhibited the calmodulin-stimulated Ca(2+)-ATPase activity. These observations support the notion that a Mg(2+)-dependent plasma membrane Ca2+ pump is present in these parasites.
Related Concept Videos
 01:19
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:37
Energy to Drive Translocation
Generally, polypeptides are unfolded by two distinct...
 01:34
ATP Driven Pumps II: P-type Pumps
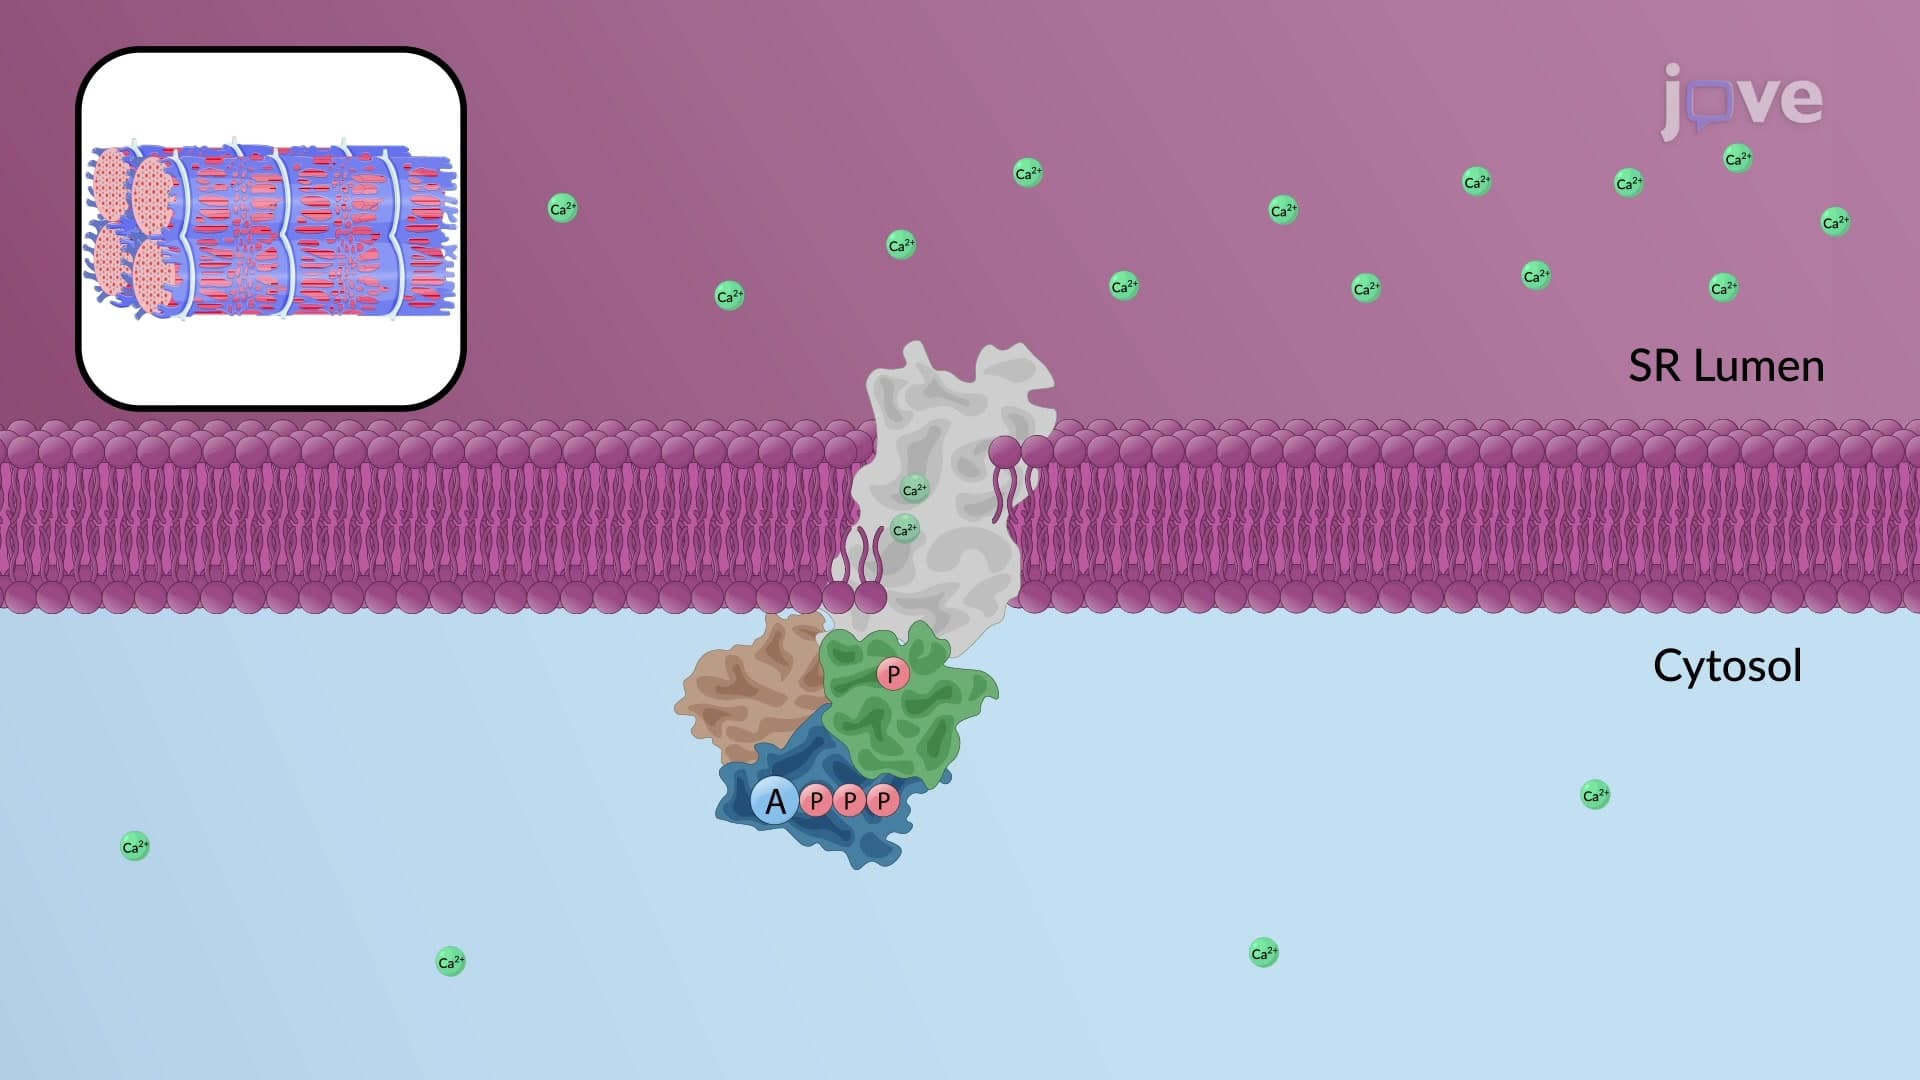
A typical P-type pump has three cytosolic domains: nucleotide-binding (N), phosphorylation (P), and activator (A) domains. These domains are connected to the membrane-spanning helices by short amino acid segments. ATP hydrolysis and covalent phosphoenzyme intermediate formation are crucial parts of the catalytic cycle. At the highly...
 01:19
Membrane Asymmetry Regulating Transporters
Flippase
Eukaryotic flippases are type-IV P-type ATPases or P4-ATPases belonging to P-type ATPase family proteins that are membrane-bound pumps involved in the ATP-mediated transport of ions and molecules across the membrane. Flippases flip specific phospholipids from the outer to the inner leaflet of a membrane. All P4-ATPases have one...
 01:27
Feedback Regulation of Calcium Concentration
Various transmembrane receptors, such as G protein-coupled receptors (GPCRs), elicit a response to extracellular signals by increasing cytosolic calcium. Activated GPCRs...
 01:16
Calmodulin-dependent Signaling
The Ca2+-CaM complex does not have enzymatic activity by itself. Instead, the complex binds downstream target proteins, including membrane proteins or enzymes,...