
SUMO-1 transiently localizes to Cajal bodies in mammalian neurons
J Navascues1, R Bengoechea, O Tapia
1Departamento de Anatomia y Biologia Celular, Unidad de Biomedicina (C.S.I.C), Universidad de Cantabria, Santander, y Centro de Investigación Biomedica en Red sobre Enfermedades Neurodegenerativas (CIBERNED), Spain.

Abstract:
Cajal bodies (CBs) are nuclear organelles involved in the maturation of small nuclear ribonucleoproteins required for the processing of pre-mRNAs. They concentrate coilin, splicing factors and the survival of motor neuron protein (SMN). By using immunocytochemistry and transfection experiments with GFP-SUMO-1, DsRed1-Ubc9, GFP-coilin and GFP-SMN constructs we demonstrate the presence of SUMO-1 and the SUMO conjugating enzyme (Ubc9) in a subset of CBs in undifferentiated neuron-like UR61 cells. Furthermore, SUMO-1 is transiently localized into neuronal CBs from adult nervous tissue in response to osmotic stress or inhibition of methyltransferase activity. SUMO-1-positive CBs contain coilin, SMN and small nuclear ribonucleoproteins, suggesting that they are functional CBs involved in pre-mRNA processing. Since coilin and SMN have several putative motifs of SUMO-1 modification, we suggest that the sumoylation of coilin and/or SMN might play a role in the molecular reorganization of CBs during the neuronal differentiation or stress-response.
Related Concept Videos
 01:26
Fusion of Secretory Vesicles with the Plasma Membrane
In 1993, Jim Rothman proposed that the antiparallel pairing of vesicular and transmembrane SNAREs, or...
 01:46
Nuclear Localization Signals and Import
 01:12
Golgi Matrix Proteins
One of the first identified Golgi matrix proteins was GM130, a rod-like protein located in the cis-Golgi. Subsequently, many Golgi...
 02:10
Additional Subnuclear Structures
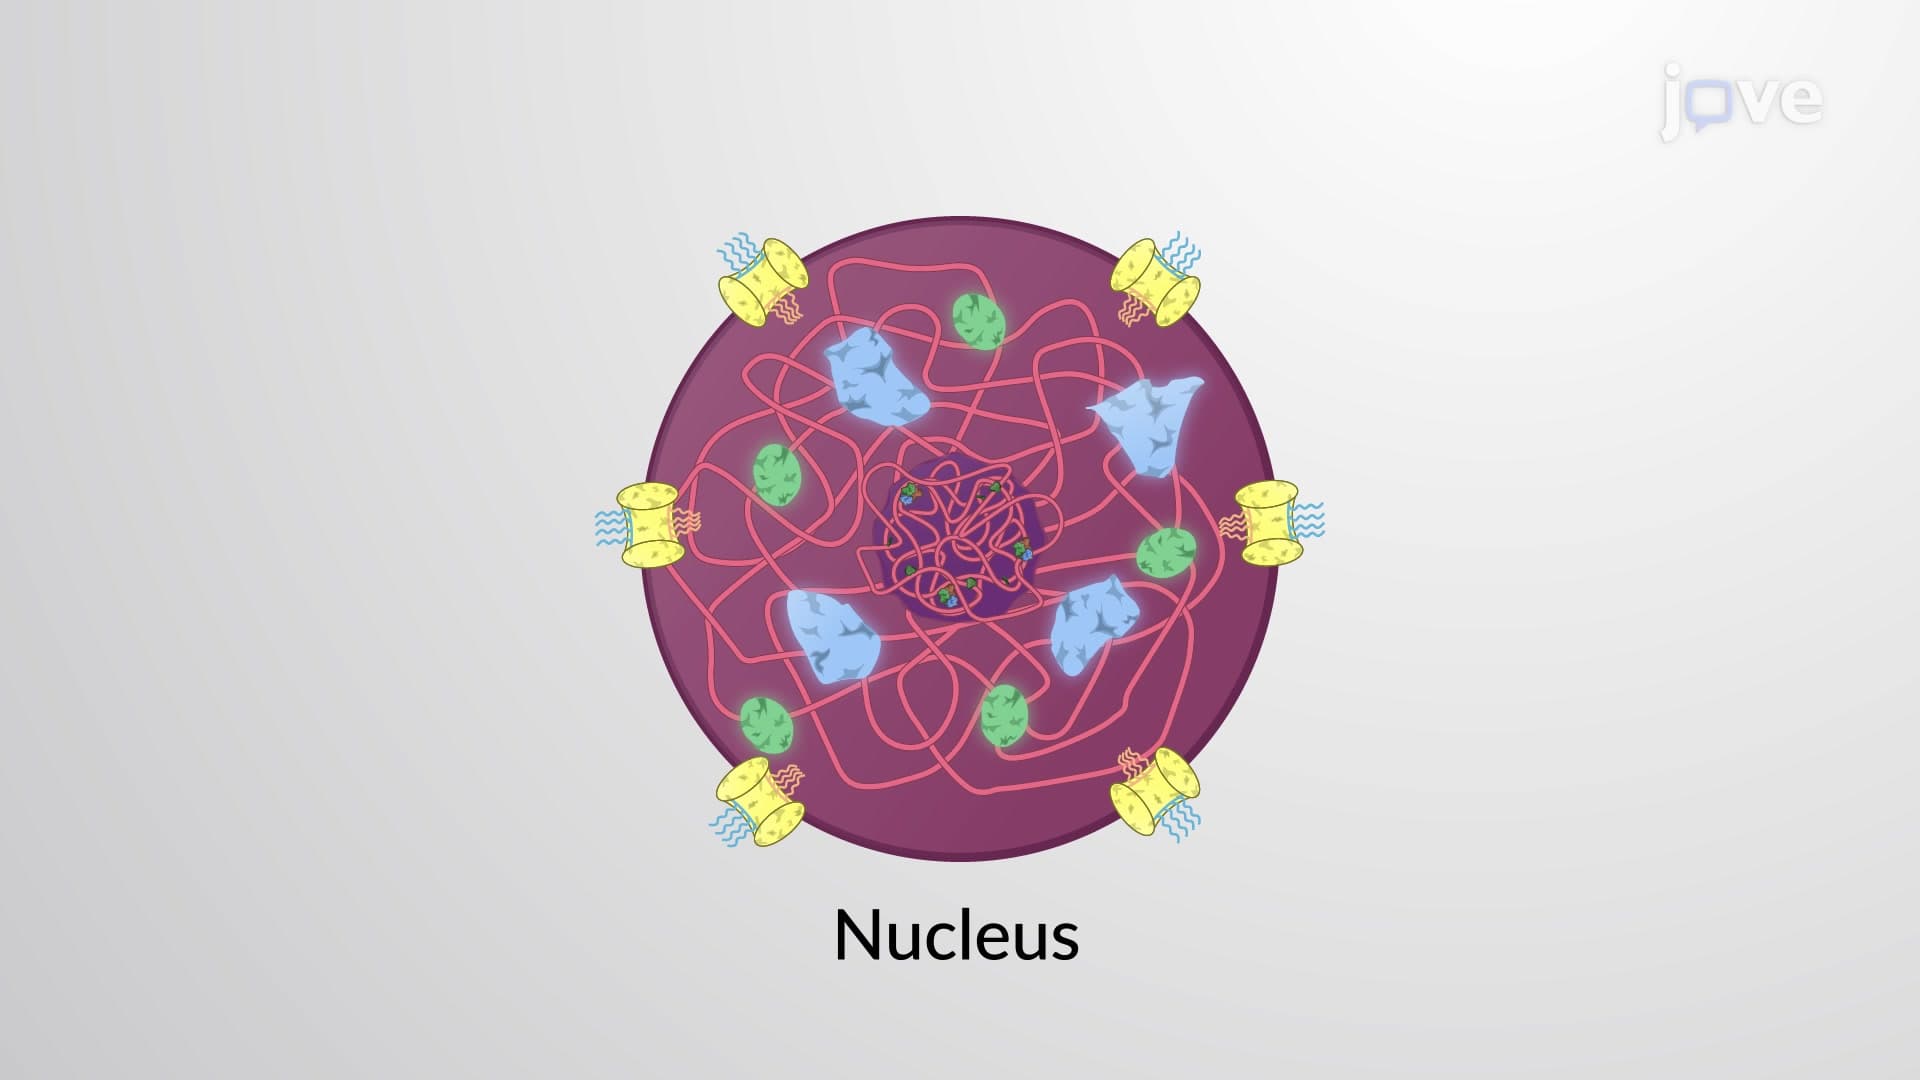
The nucleus contains many membrane-less subnuclear organelles or nuclear bodies, such as nucleoli, Cajal bodies, speckles, paraspeckles, etc. These nuclear...
 01:27
Post-translational Translocation of Proteins to the RER
Targeting proteins to the ER
Hsp40 and Hsp70 chaperone molecules bind the translated proteins in the cytosol to prevent their folding. The chaperone binding helps to keep the signal...
 01:13
Cytoskeletal Accessory Proteins