Role of the N-terminal domain of phiC31 integrase in attB-attP synapsis

Paul A Rowley1, Margaret C M Smith

  • 1Institute of Medical Sciences, University of Aberdeen, Foresterhill, Aberdeen AB25 2ZD, United Kingdom.

Journal of Bacteriology
|August 12, 2008
PubMed

Related Concept Videos

Mechanism of Conjugation01:19

Mechanism of Conjugation

Bacterial conjugation is a mechanism of horizontal gene transfer that enables the exchange of genetic material between bacterial cells through direct contact. This process is facilitated by a donor cell carrying a conjugative plasmid, which encodes genes necessary for pilus formation, DNA replication, and transfer. The conjugative plasmid plays a central role in initiating and executing the transfer of genetic material.The tra region of the conjugative plasmid encodes proteins responsible for...
LTR Retrotransposons03:08

LTR Retrotransposons

LTR retrotransposons are class I transposable elements with long terminal repeats flanking an internal coding region. These elements are less abundant in mammals compared to other class I transposable elements. About 8 percent of human genomic DNA comprises LTR retrotransposons. Some of the common examples of LTR retrotransposons are Ty elements in yeast and Copia elements in Drosophila.
The internal coding region of LTR retrotransposons and their mechanism of transposition closely resembles a...
Tail-anchoring of Proteins in the ER Membrane01:45

Tail-anchoring of Proteins in the ER Membrane

Tail-anchored, or TA, proteins are estimated to make up to 3-5% of membrane proteins found in the eukaryotic cell. Such proteins have a single transmembrane domain located approximately 30 amino acid residues upstream from the C-terminal end. As a result, the signal recognition particle (SRP) cannot guide a TA protein to the ER membrane for cotranslational insertion. Hence, they are integrated into the ER membrane post-translationally using their C-terminal end as the anchor. TA proteins...
Phosphoinositides and PIPs01:42

Phosphoinositides and PIPs

Phosphoinositides are a group of phospholipids containing a glycerol backbone with two fatty acid chains and a phosphate attached to a myoinositol sugar ring. The inositol head group extends into the cytoplasm, where it is modified by adding phosphate groups to form phosphatidylinositol phosphates or PIPs.
Different phosphoinositides are synthesized and recruited on the cytosolic face of the plasma membrane. The localization of specific phosphoinositides concentrated in separate membrane...
Protein Transport into the Inner Mitochondrial Membrane01:34

Protein Transport into the Inner Mitochondrial Membrane

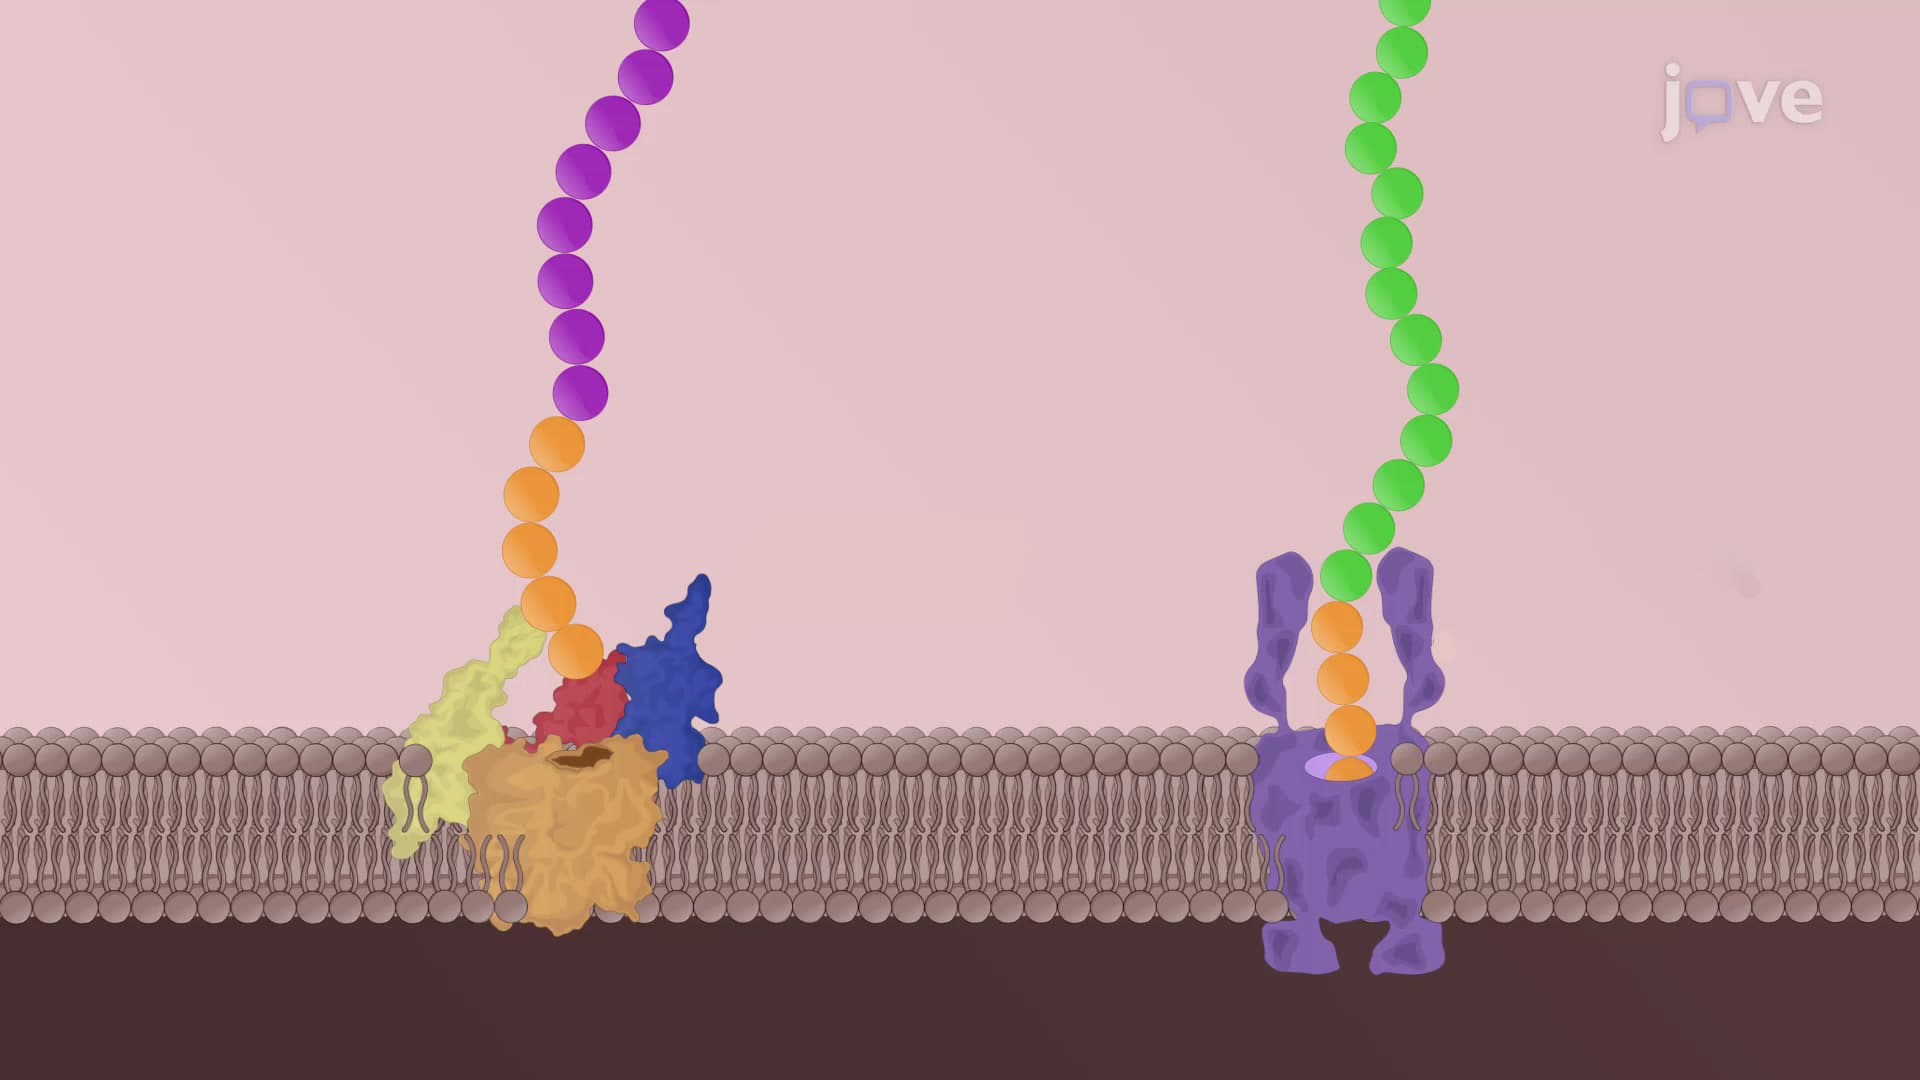
Nuclear encoded mitochondrial precursors are imported to the inner membrane in a multistep process involving two separate translocons, TIM22 and TIM23. TIM23 is a cation-selective pore that remains closed by the N terminal segment of the protein. Negative charges on the TIM23 act as a receptor for the incoming precursor, pulling the positively charged matrix-targeting sequence for peptide insertion and translocation.
Transport of mitochondrial precursors across the TIM23 channel is driven by...
Translocation of Proteins into the Mitochondria01:19

Translocation of Proteins into the Mitochondria

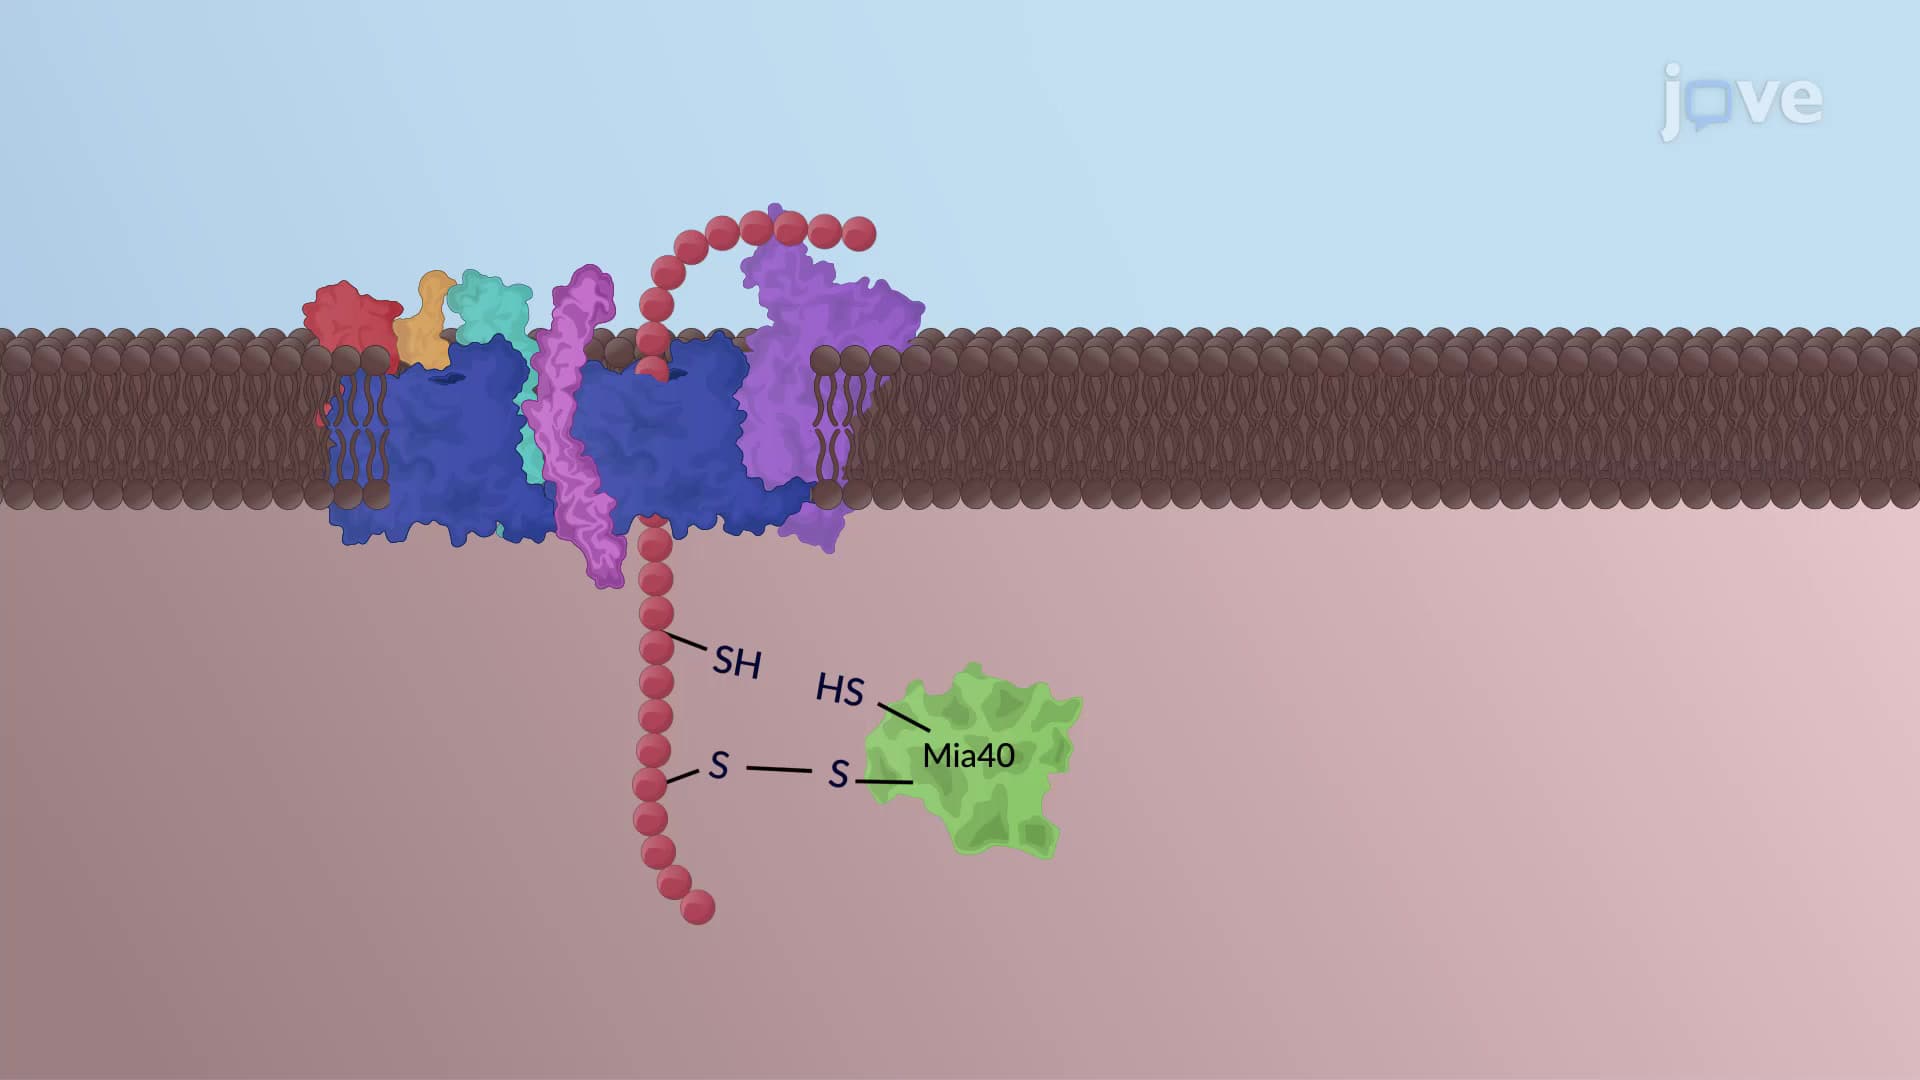
Mitochondrial precursors are translocated to the internal subcompartments via independent mechanisms involving distinct protein machineries called translocases.
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...