Related Experiment Video
Updated: Jun 27, 2026

Single-molecule Super-resolution Imaging of Phosphatidylinositol 4,5-bisphosphate in the Plasma Membrane with Novel Fluorescent Probes
Published on: October 15, 2016
Myelin basic protein co-distributes with other PI(4,5)P2-sequestering proteins in Triton X-100 detergent-resistant
Abdiwahab A Musse1, Wen Gao, Godha Rangaraj
1Department of Molecular and Cellular Biology, University of Guelph, 50 Stone Road East, Guelph, Ontario, Canada.

Abstract:
The 18.5kDa isoform of myelin basic protein (MBP) has recently been shown to sequester phosphatidylinositol-(4,5)-bis-phosphate (PI(4,5)P(2)) in vesicular membranes in vitro, as do domains of other membrane- and cytoskeleton-associated proteins such as MARCKS (myristoylated alanine-rich C kinase substrate) and GAP-43 (growth-associated protein of 43kDa), known collectively as "PI(4,5)P(2)-modulins" [Musse et al., Biochemistry, 47 (2008) 10372-10382 (doi:10.1021/bi801302b)]. Here, we demonstrate co-localisation of MBP and MARCKS in primary rat oligodendrocytes, and co-distribution of MBP, MARCKS, and GAP-43 in lipid raft fractions recovered from Triton X-100 detergent-extracted isolated myelin and brain homogenates. The results lend further support to MBP's multifunctionality, particularly as an additional modulator of PI(4,5)P(2) availability in myelin.
Insights
Myelin basic protein (MBP) sequesters phosphatidylinositol-(4,5)-bis-phosphate (PI(4,5)P(2)), similar to other PI(4,5)P(2)-modulins. This study shows MBP, MARCKS, and GAP-43 co-localize in myelin, supporting MBP's role in regulating PI(4,5)P(2) in myelin.
Area of Science:
- Neuroscience
- Cell Biology
- Biochemistry
Background:
- Myelin basic protein (MBP) is a key component of myelin.
- Certain proteins, known as PI(4,5)P(2)-modulins, bind and sequester phosphatidylinositol-(4,5)-bis-phosphate (PI(4,5)P(2)).
- MBP's interaction with PI(4,5)P(2) was previously demonstrated in vitro.
Purpose of the Study:
- To investigate the co-localization and co-distribution of MBP with other known PI(4,5)P(2)-modulins.
- To explore the role of MBP in modulating PI(4,5)P(2) availability within myelin.
Main Methods:
- Co-localization studies in primary rat oligodendrocytes.
- Analysis of lipid raft fractions from isolated myelin and brain homogenates.
- Triton X-100 detergent extraction.
Main Results:
- MBP and Myristoylated alanine-rich C kinase substrate (MARCKS) were found to co-localize in primary rat oligodendrocytes.
- MBP, MARCKS, and Growth-associated protein of 43kDa (GAP-43) co-distributed in lipid raft fractions.
- Evidence supports MBP's role as a PI(4,5)P(2) modulator in myelin.
Conclusions:
- MBP functions similarly to other PI(4,5)P(2)-modulins.
- MBP, MARCKS, and GAP-43 are present together in myelin lipid rafts.
- These findings highlight MBP's multifunctional nature and its involvement in regulating PI(4,5)P(2) in the myelin sheath.
More Related Videos
 10:31
A Liposome Membrane Permeability Assay for Investigating the Effects of Phosphatidylinositol Phosphate Groups on Membranotropic Action of Venom PLA2
Published on: September 26, 2025
 04:25
Enriching Subcellular Proteins in Leptospira Using a Triton X-114-Based Fractionation Approach
Published on: August 8, 2025
Related Concept Videos
 01:42
Phosphoinositides and PIPs
Different phosphoinositides are synthesized and recruited on the cytosolic face of the plasma membrane. The localization of specific phosphoinositides concentrated in separate membrane...
 01:18
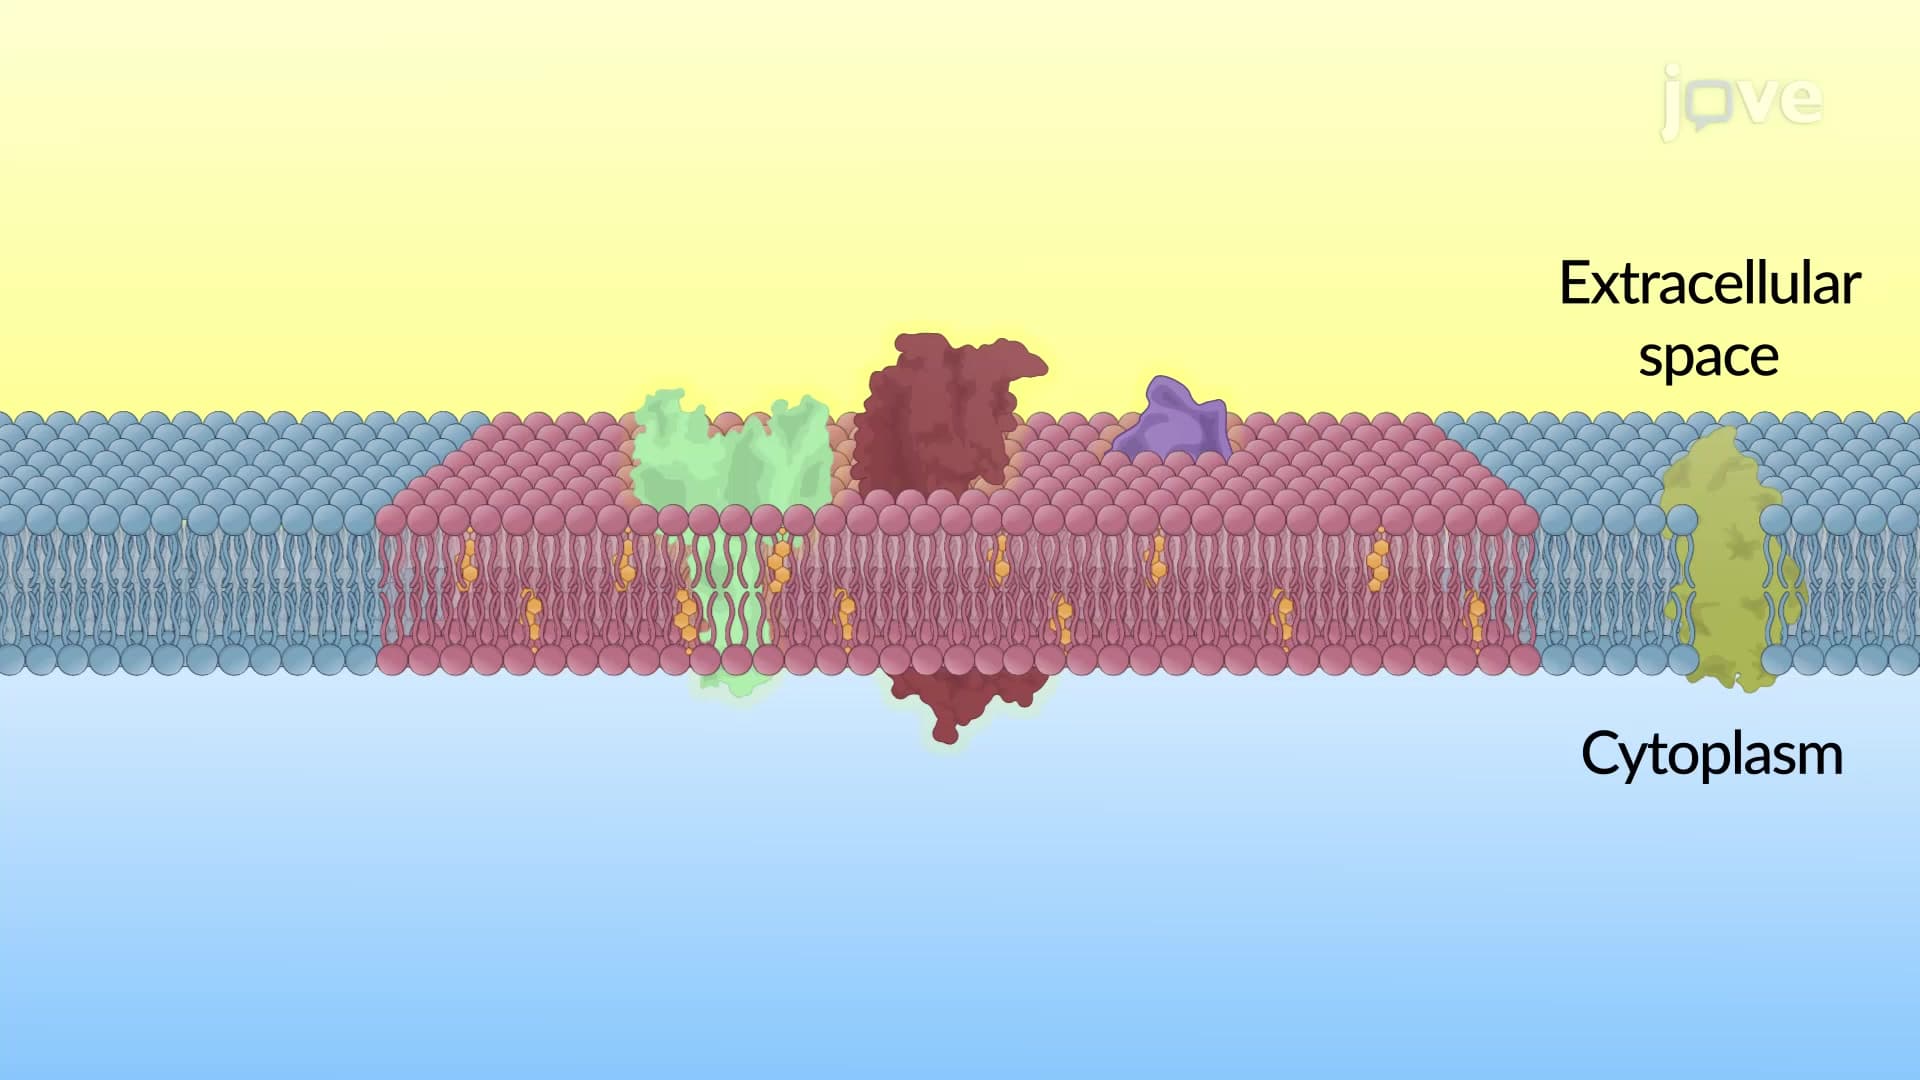
Membrane Domains
Protein Domains
The membrane comprises a group of distinct proteins responsible for carrying out a cell's specific function. For example, the plasma membrane of the human sperm, or a single germ cell, contains a unique set of proteins in the anterior...
 01:26
Membrane Fluidity
Mosaic nature of the membrane
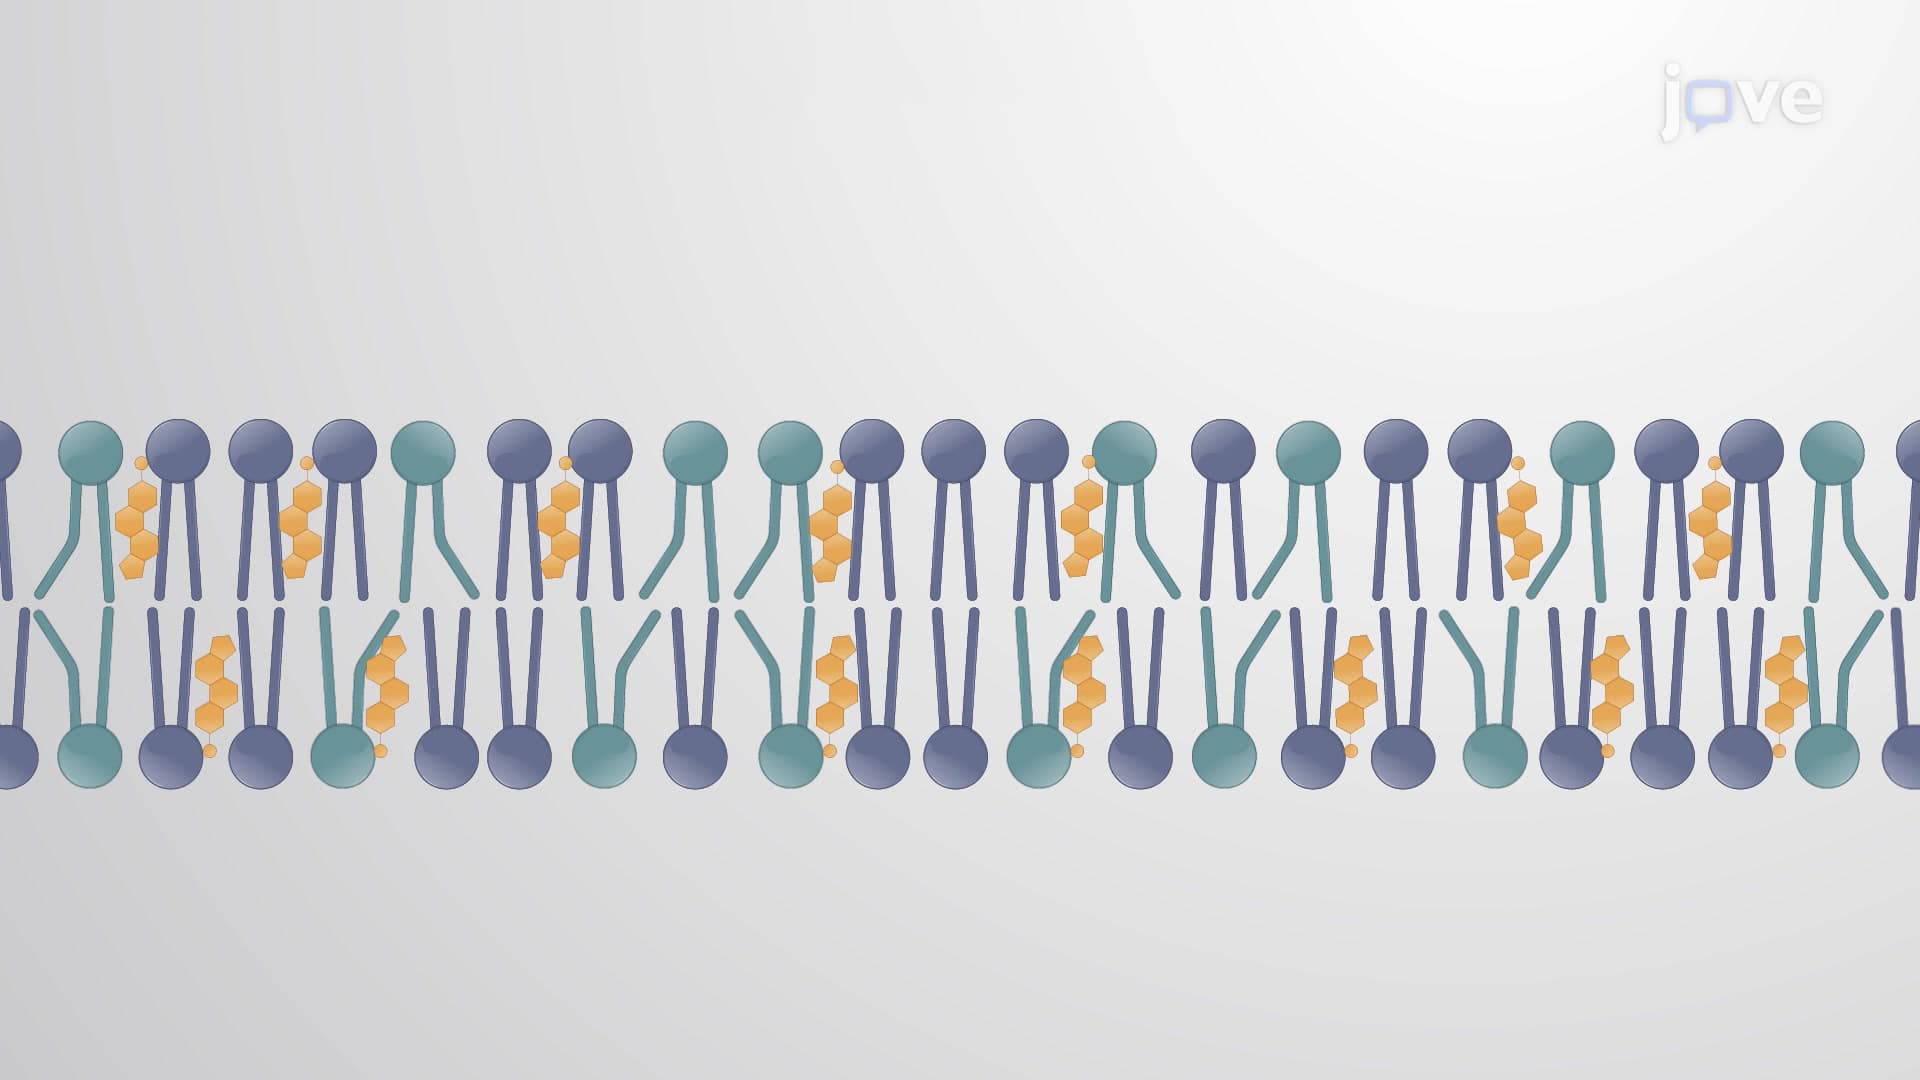
The mosaic characteristic of the membrane helps the plasma membrane remain fluid. The integral proteins and lipids exist as separate but loosely-attached molecules in the membrane. The membrane is a relatively...
 01:21
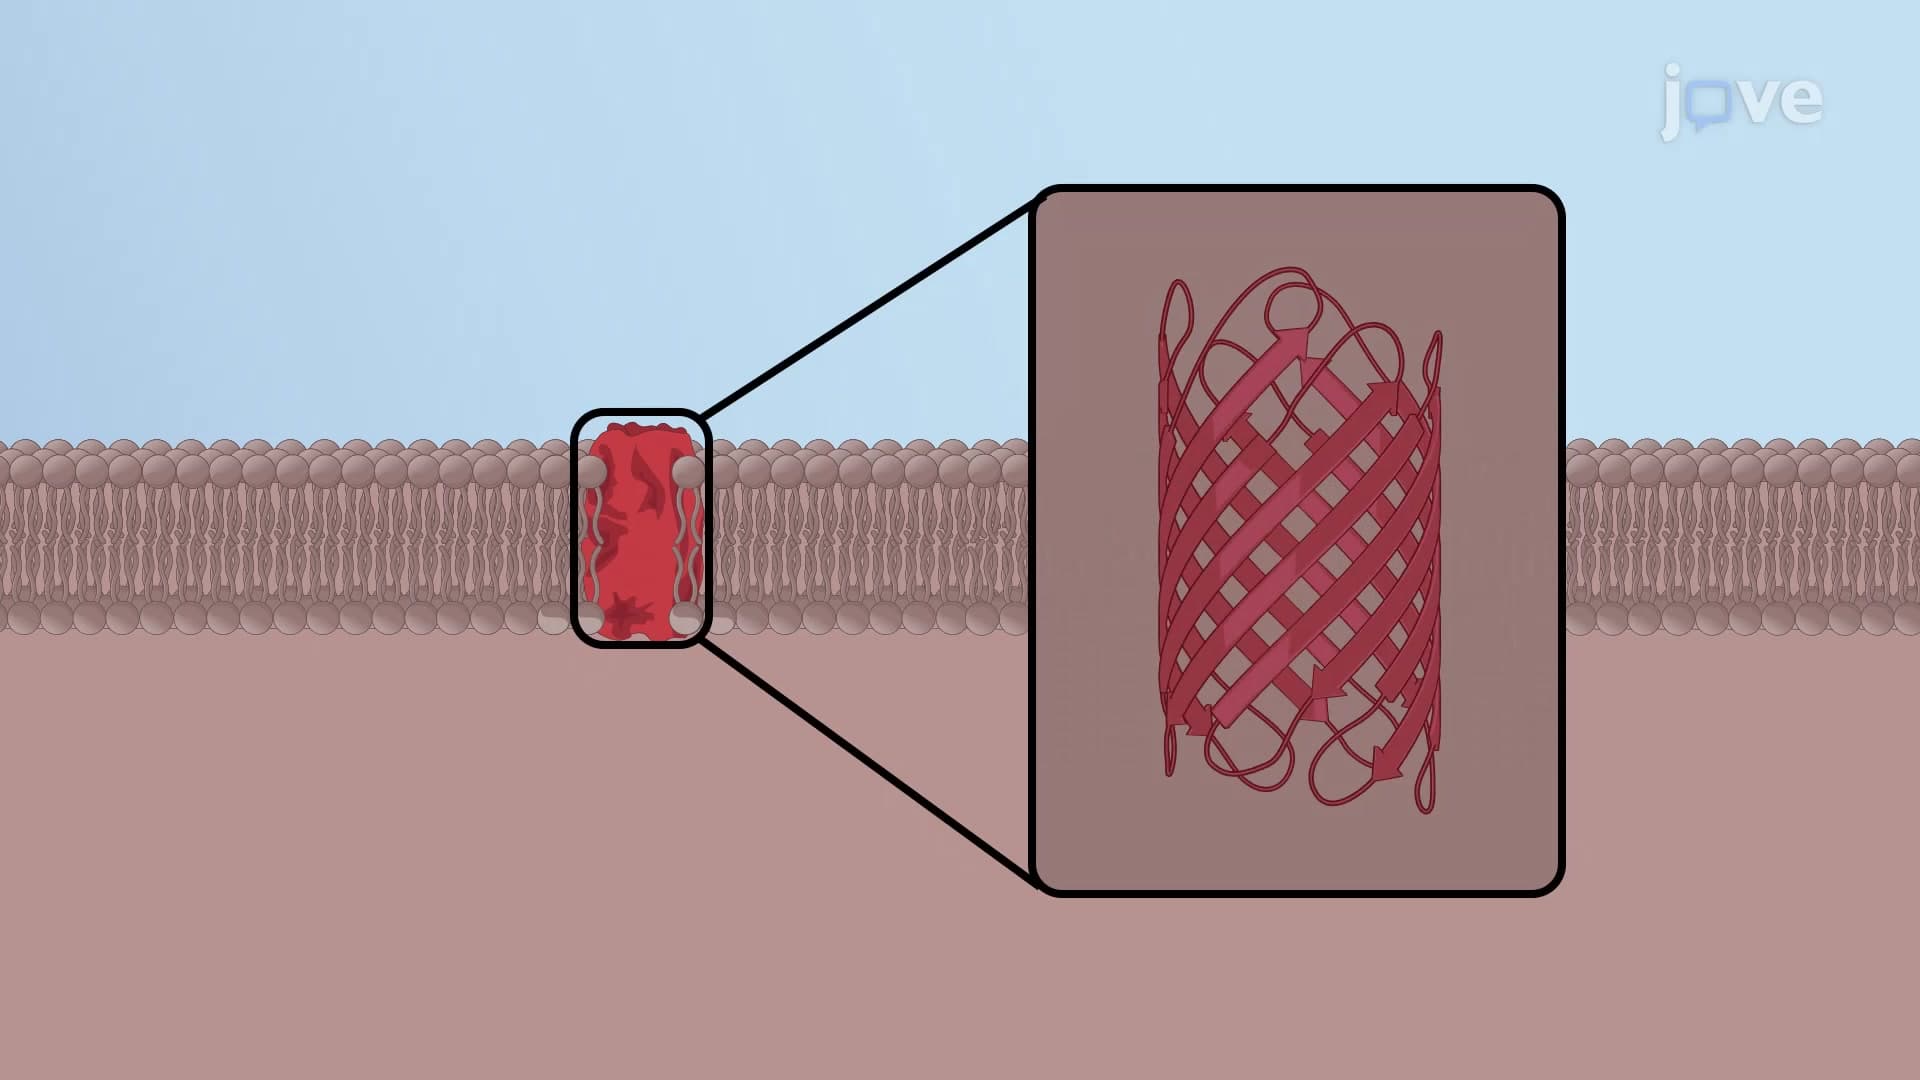
Structure of Porins
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...
 01:19
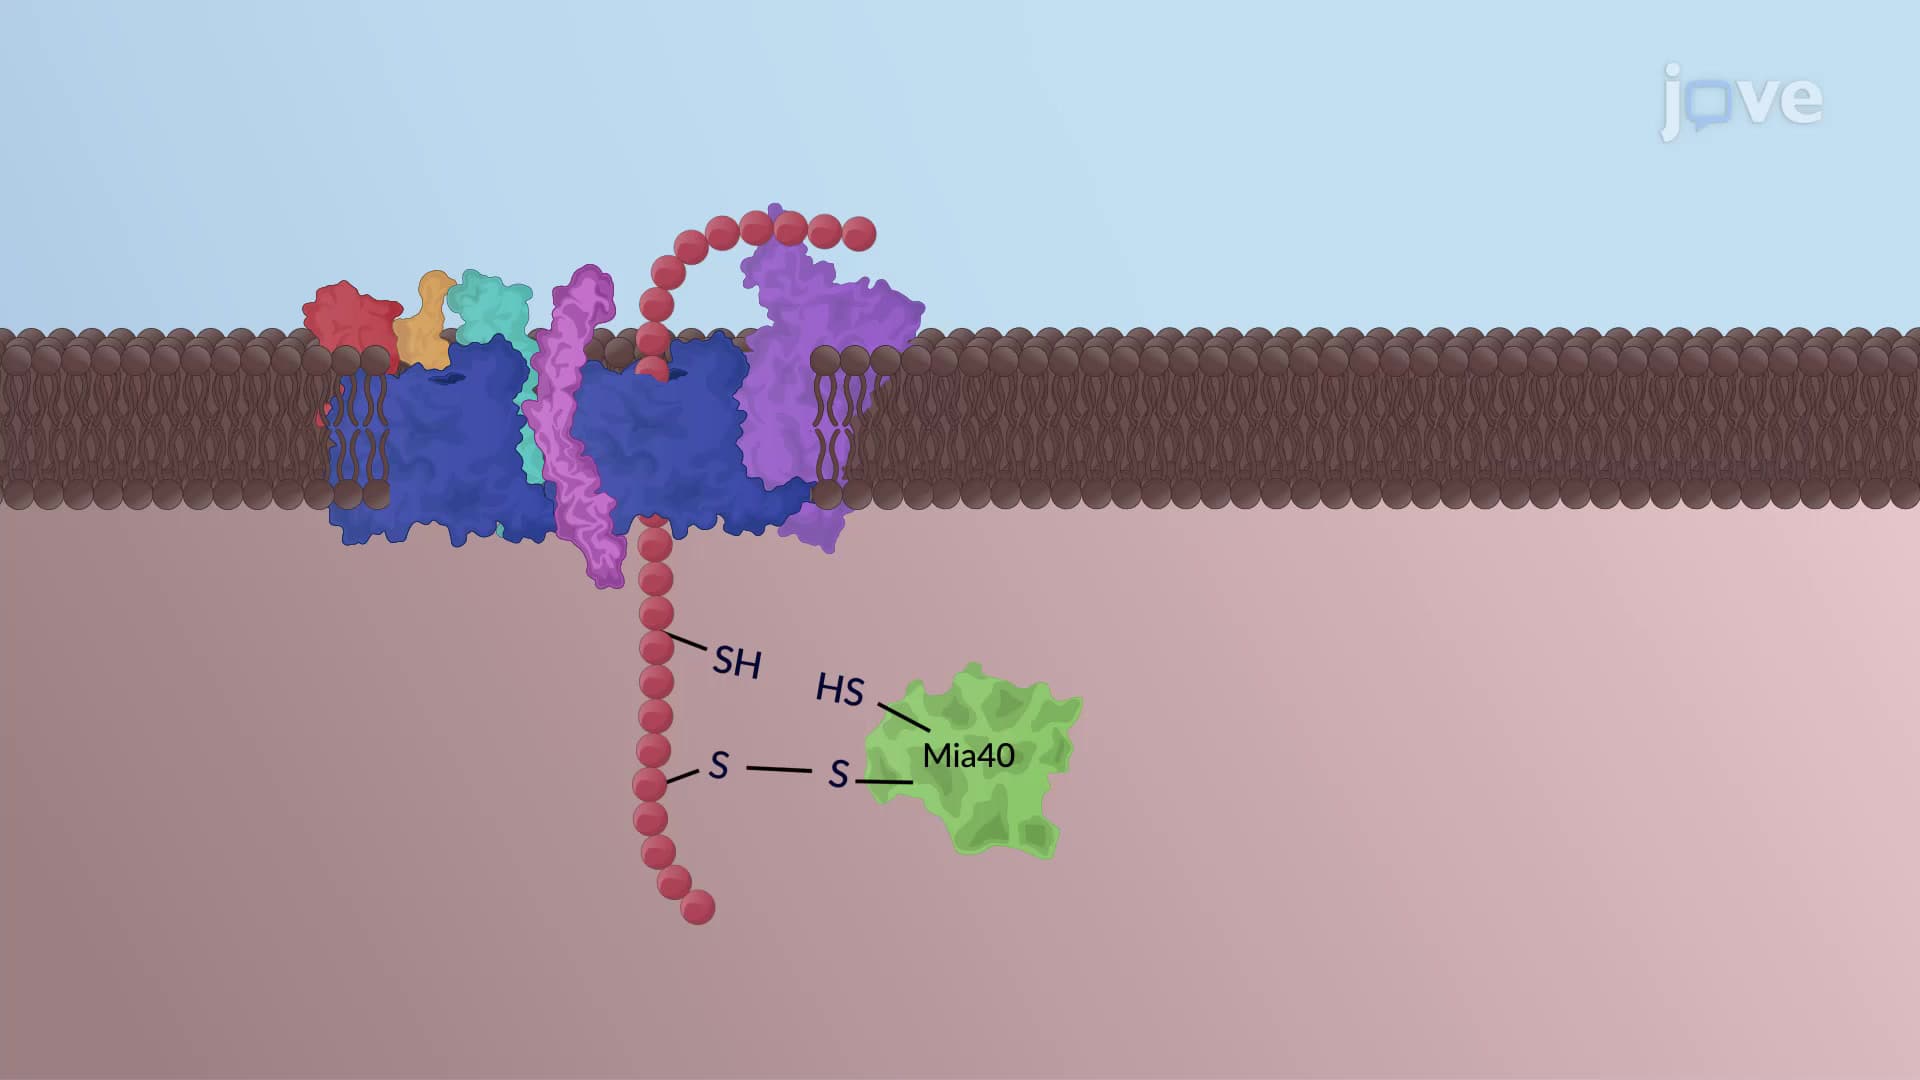
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...