Related Experiment Video
Updated: Jun 27, 2026

Temporal Analysis of the Nuclear-to-cytoplasmic Translocation of a Herpes Simplex Virus 1 Protein by Immunofluorescent Confocal Microscopy
Published on: November 4, 2018
Nuclear import of HSV-1 DNA polymerase processivity factor UL42 is mediated by a C-terminally located bipartite
Gualtiero Alvisi1, Simone Avanzi, Daniele Musiani
1Dipartimento di Ematologia e Scienze Oncologiche L.A. Seragnoli, Universita degli Studi di Bologna, Bologna, Italia. gualtiero.alvisi3@unibo.it

Abstract:
The polymerase accessory protein of the human herpes simplex virus type 1 (HSV-1) DNA polymerase UL42 plays an essential role in viral replication, conferring processivity to the catalytic subunit UL30. We show here that UL42 is imported to the nucleus of living cells in a Ran- and energy-dependent fashion, through a process that requires a C-terminally located bipartite nuclear localization signal (UL42-NLSbip; PTTKRGRSGGEDARADALKKPK(413)). Moreover cytoplasmic mutant derivatives of UL42 lacking UL42-NLSbip are partially relocalized into the cell nucleus upon HSV-1 infection or coexpression with UL30, implying that the HSV-1 DNA polymerase holoenzyme can assemble in the cytoplasm before nuclear translocation occurs, thus explaining why the UL42 C-terminal domain is not strictly required for viral replication in cultured cells. However, mutation of both UL30 and UL42 NLS results in retention of the DNA polymerase holoenzyme in the cytoplasm, suggesting that simultaneous inhibition of both NLSs could represent a viable strategy to hinder HSV-1 replication. Intriguingly, UL42-NLSbip is composed of two stretches of basic amino acids matching the consensus for classical monopartite NLSs (NLSA, PTTKRGR(397); NLSB, KKPK(413)), neither of which are capable of targeting GFP to the nucleus on their own, consistent with the hypothesis that P and G residues in position +3 of monopartite NLSs are not compatible with nuclear transport in the absence of additional basic sequences located in close proximity. Our results showing that substitution of G or P of the NLS with an A residue partially confers NLS function will help to redefine the consensus for monopartite NLSs.
Insights
The human herpes simplex virus type 1 (HSV-1) DNA polymerase accessory protein UL42 is imported into the nucleus via a bipartite nuclear localization signal. Inhibiting both UL42 and UL30 nuclear localization signals may block HSV-1 replication.
Area of Science:
- Virology
- Molecular Biology
- Cell Biology
Background:
- The human herpes simplex virus type 1 (HSV-1) DNA polymerase accessory protein UL42 is crucial for viral replication.
- UL42 enhances the processivity of the catalytic subunit UL30.
Purpose of the Study:
- To investigate the nuclear import mechanism of HSV-1 UL42.
- To explore the role of UL42's nuclear localization signal (NLS) in viral replication.
- To assess the potential of targeting NLSs for antiviral strategies.
Main Methods:
- Studied UL42 nuclear import in living cells using Ran- and energy-dependent assays.
- Utilized mutant UL42 derivatives lacking the bipartite NLS (UL42-NLSbip).
- Examined nuclear translocation of the HSV-1 DNA polymerase holoenzyme (UL42 and UL30) upon infection or coexpression.
- Investigated the function of individual NLS components and their impact on nuclear transport.
Main Results:
- UL42 is imported into the nucleus via a C-terminal bipartite NLS (UL42-NLSbip) in a Ran- and energy-dependent manner.
- Cytoplasmic UL42 mutants relocalize to the nucleus upon HSV-1 infection or UL30 coexpression, suggesting cytoplasmic holoenzyme assembly.
- Simultaneous mutation of UL42 and UL30 NLSs retains the holoenzyme in the cytoplasm, inhibiting viral replication.
- Individual NLS components (NLSA and NLSB) are insufficient for nuclear targeting alone, indicating a requirement for cooperative function.
- Substitution of specific residues (P or G) in the NLS with alanine partially restores nuclear import function.
Conclusions:
- The HSV-1 DNA polymerase holoenzyme can assemble in the cytoplasm before nuclear translocation.
- Targeting both UL42 and UL30 NLSs presents a potential strategy to inhibit HSV-1 replication.
- The findings redefine the consensus for monopartite NLSs, highlighting the importance of adjacent basic residues and specific amino acid compatibility (e.g., P/G at position +3).
Related Concept Videos
 01:46
Nuclear Localization Signals and Import
 01:42
Nuclear Export
NES are of three types- the canonical 10-residue long leucine-rich signal and other...
 01:34
Nuclear Protein Sorting
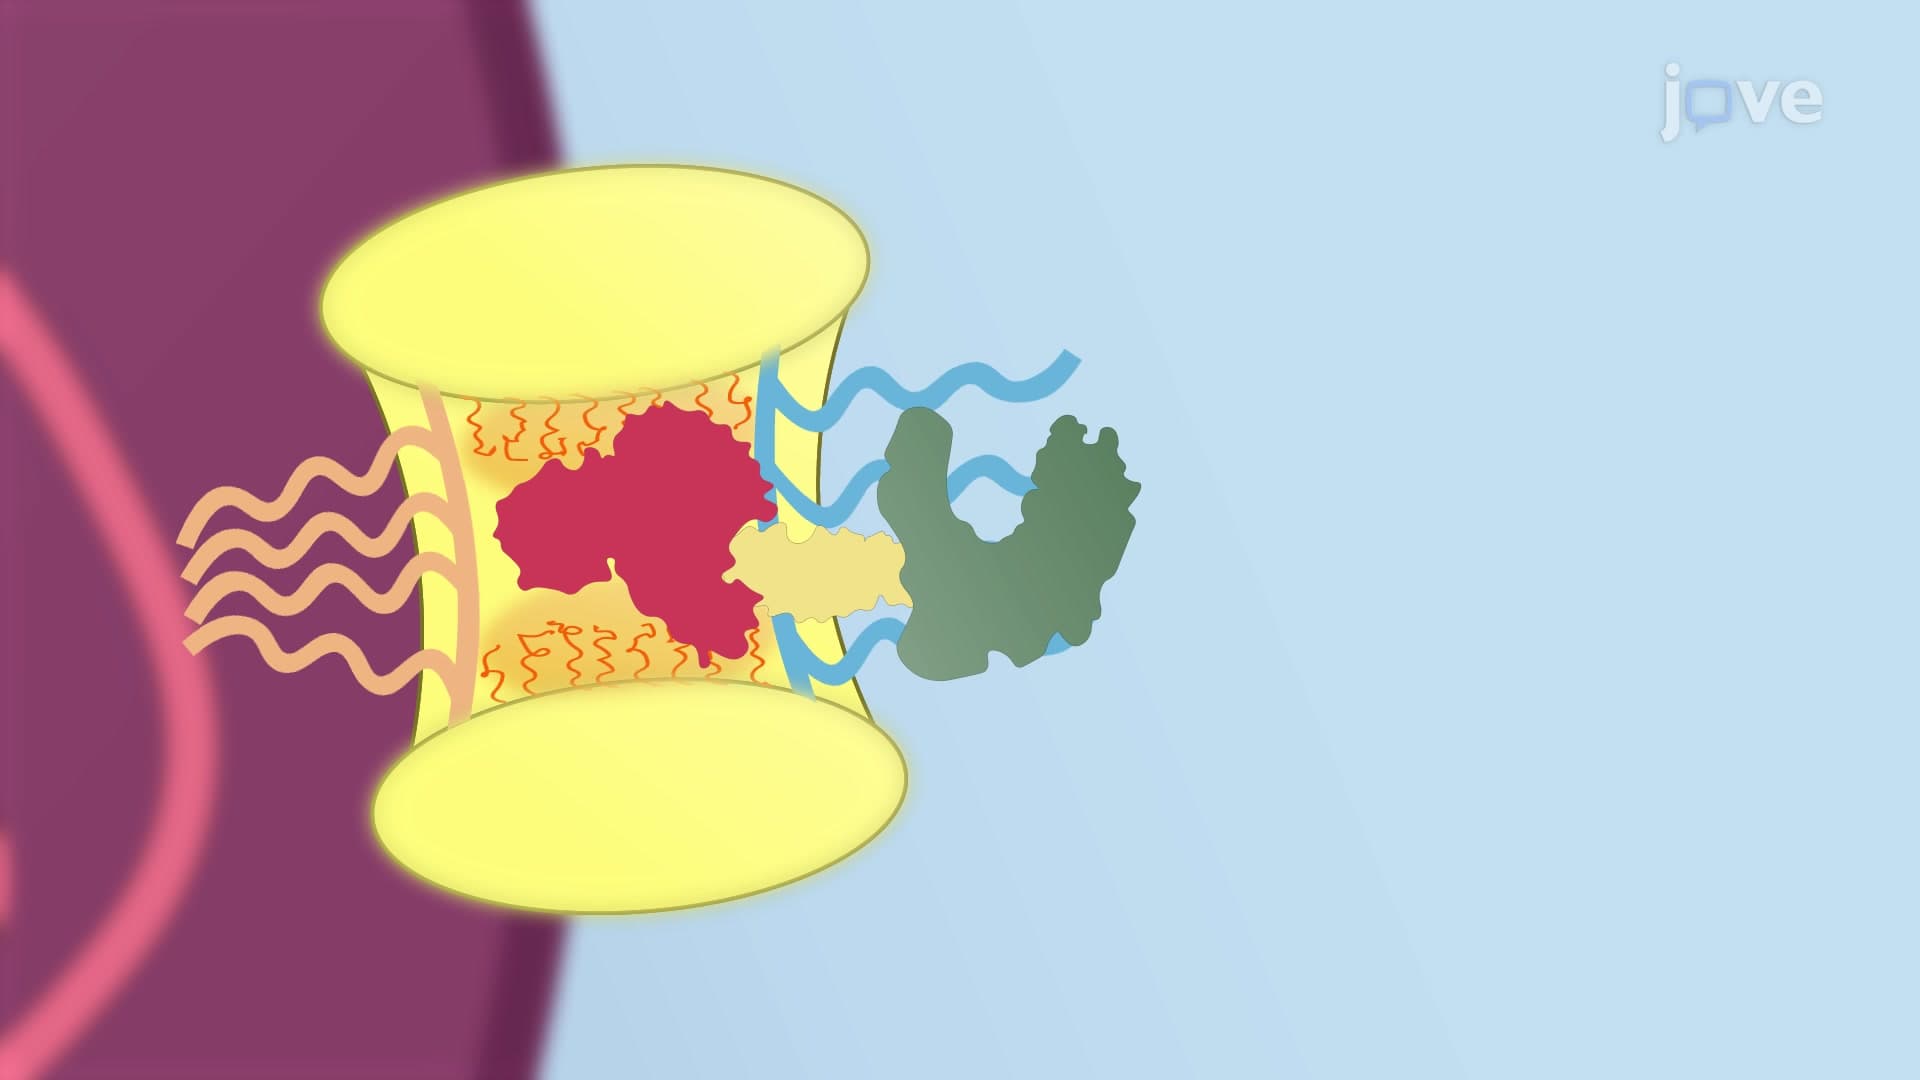
Proteins targeted to the nucleus carry nuclear localization signals or NLS recognized by import receptors in the cytosol. Similarly, proteins with nuclear export signals are recognized by export receptors. Import and export receptors are...
 01:45
Regulation of Nuclear Protein Sorting
 01:42
Directionality of Nuclear Transport
 01:38
Intralumenal Vesicles and Multivesicular Bodies