Related Experiment Video
Updated: Jun 24, 2026
Analysis of Group IV Viral SSHHPS Using In Vitro and In Silico Methods
Published on: December 21, 2019
The protease-associated domain and C-terminal extension are required for zymogen processing, sorting within the
Anna Cedzich1, Franziska Huttenlocher, Benjamin M Kuhn
1Institute of Plant Physiology and Biotechnology, Life Science Center, and Institute of Physiology, Department of Biosensorics, University of Hohenheim, D-70593 Stuttgart, Germany.

Abstract:
A transgenic plant cell suspension culture was established as a versatile and efficient expression system for the subtilase SlSBT3 from tomato. The recombinant protease was purified to homogeneity from culture supernatants by fractionated ammonium sulfate precipitation, batch adsorption to cation exchange material, and anion exchange chromatography. Purified SlSBT3 was identified as a 79-kDa glycoprotein with both complex and paucimannosidic type glycan chains at Asn(177), Asn(203), Asn(376), Asn(697), and Asn(745). SlSBT3 was found to be a very stable enzyme, being fully active at 60 degrees C and showing highest activity at alkaline conditions with a maximum between pH 7.5 and 8.0. Substrate specificity of SlSBT3 was analyzed in detail, revealing a preference for Gln and Lys in the P(1) and P(2) positions of oligopeptide substrates, respectively. Similar to bacterial, yeast, and mammalian subtilases, SlSBT3 is synthesized as a preproenzyme, and processing of the prodomain in the endoplasmic reticulum is a prerequisite for passage through the secretory pathway. SlSBT3 S538A and S538C active site mutants accumulated intracellularly as unprocessed zymogens, indicating that prodomain cleavage occurs autocatalytically. The wild-type SlSBT3 protein failed to cleave the prodomain of the S538A mutant in trans, demonstrating that zymogen maturation is an intramolecular process. Distinguishing features of plant as compared with mammalian subtilases include the insertion of a large protease-associated domain between the His and Ser residues of the catalytic triad and the C-terminal extension to the catalytic domain. Both features were found to be required for SlSBT3 activity and, consequently, for prodomain processing and secretion.
More Related Videos
 05:20
A Colorimetric Assay that Specifically Measures Granzyme B Proteolytic Activity: Hydrolysis of Boc-Ala-Ala-Asp-S-Bzl
Published on: November 28, 2014
 09:22
Budding Yeast Protein Extraction and Purification for the Study of Function, Interactions, and Post-translational Modifications
Published on: October 30, 2013
Related Concept Videos
 01:19
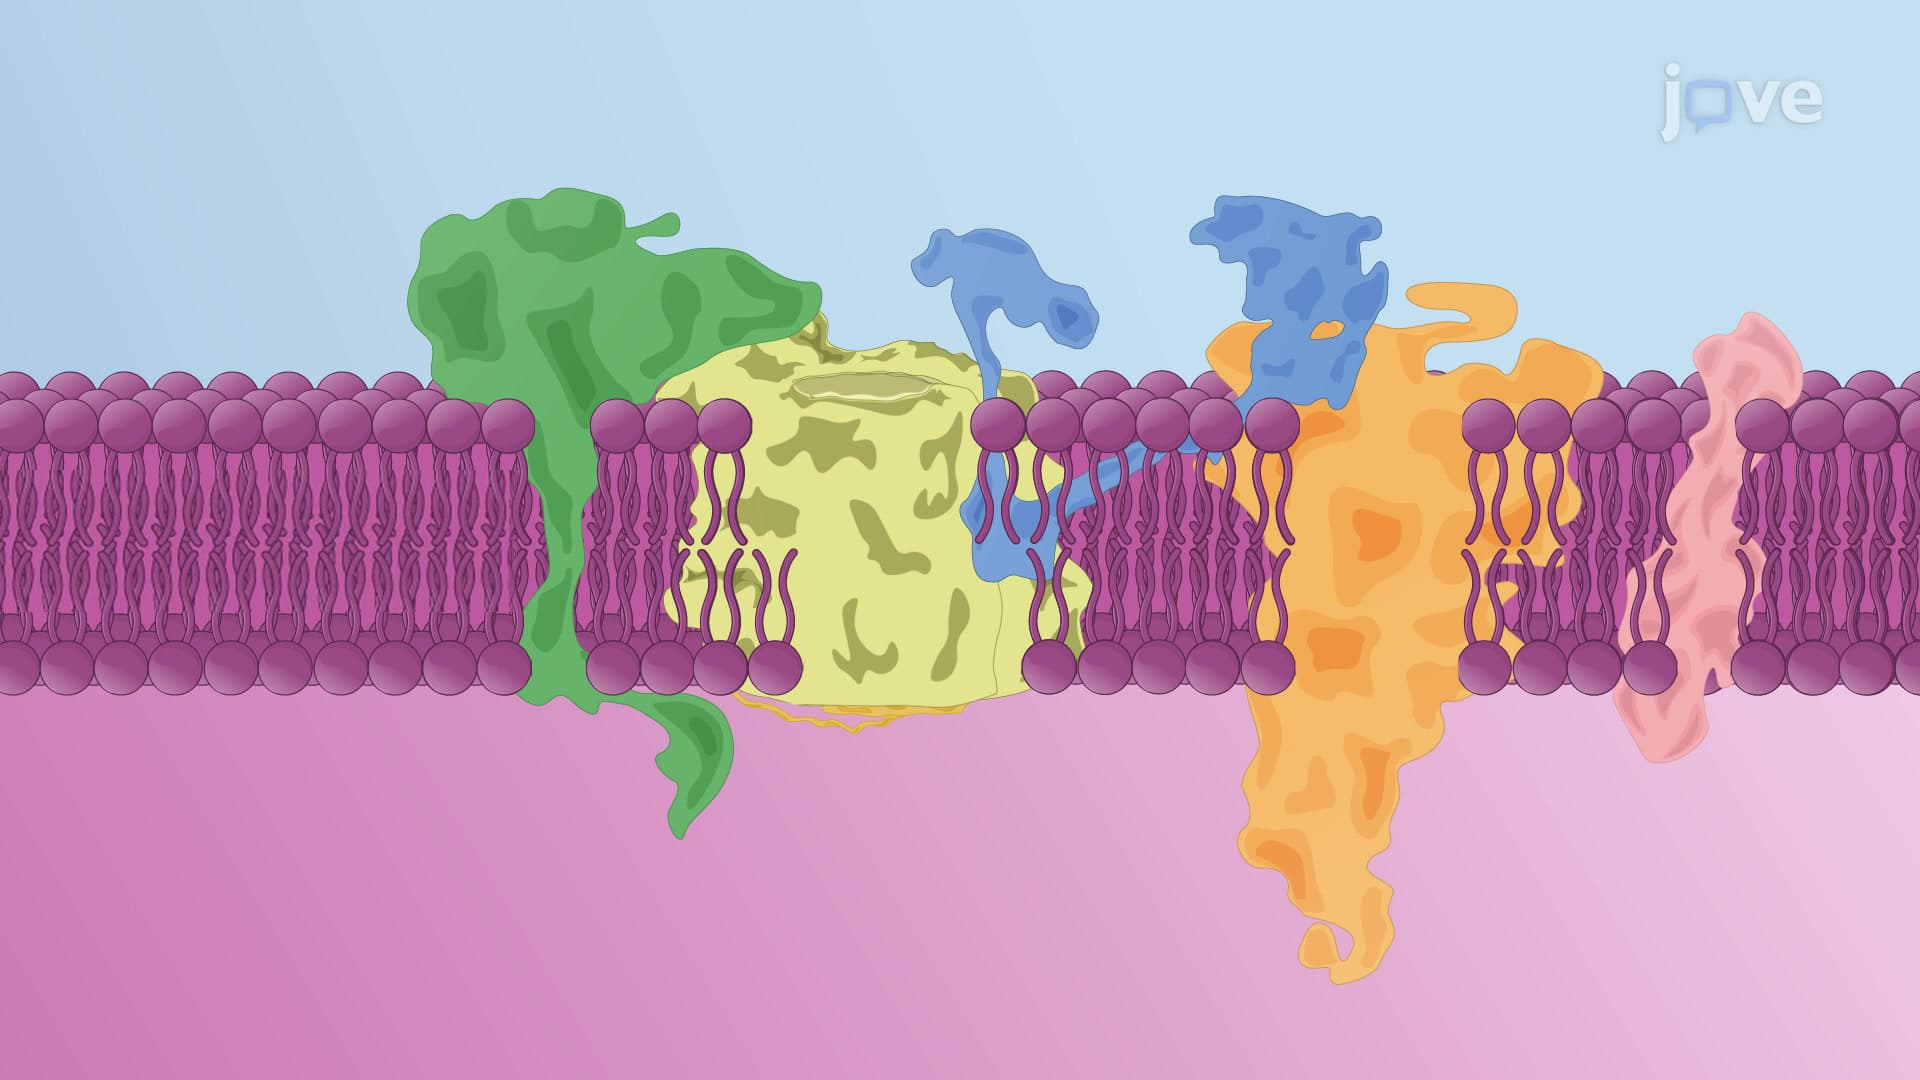
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:28
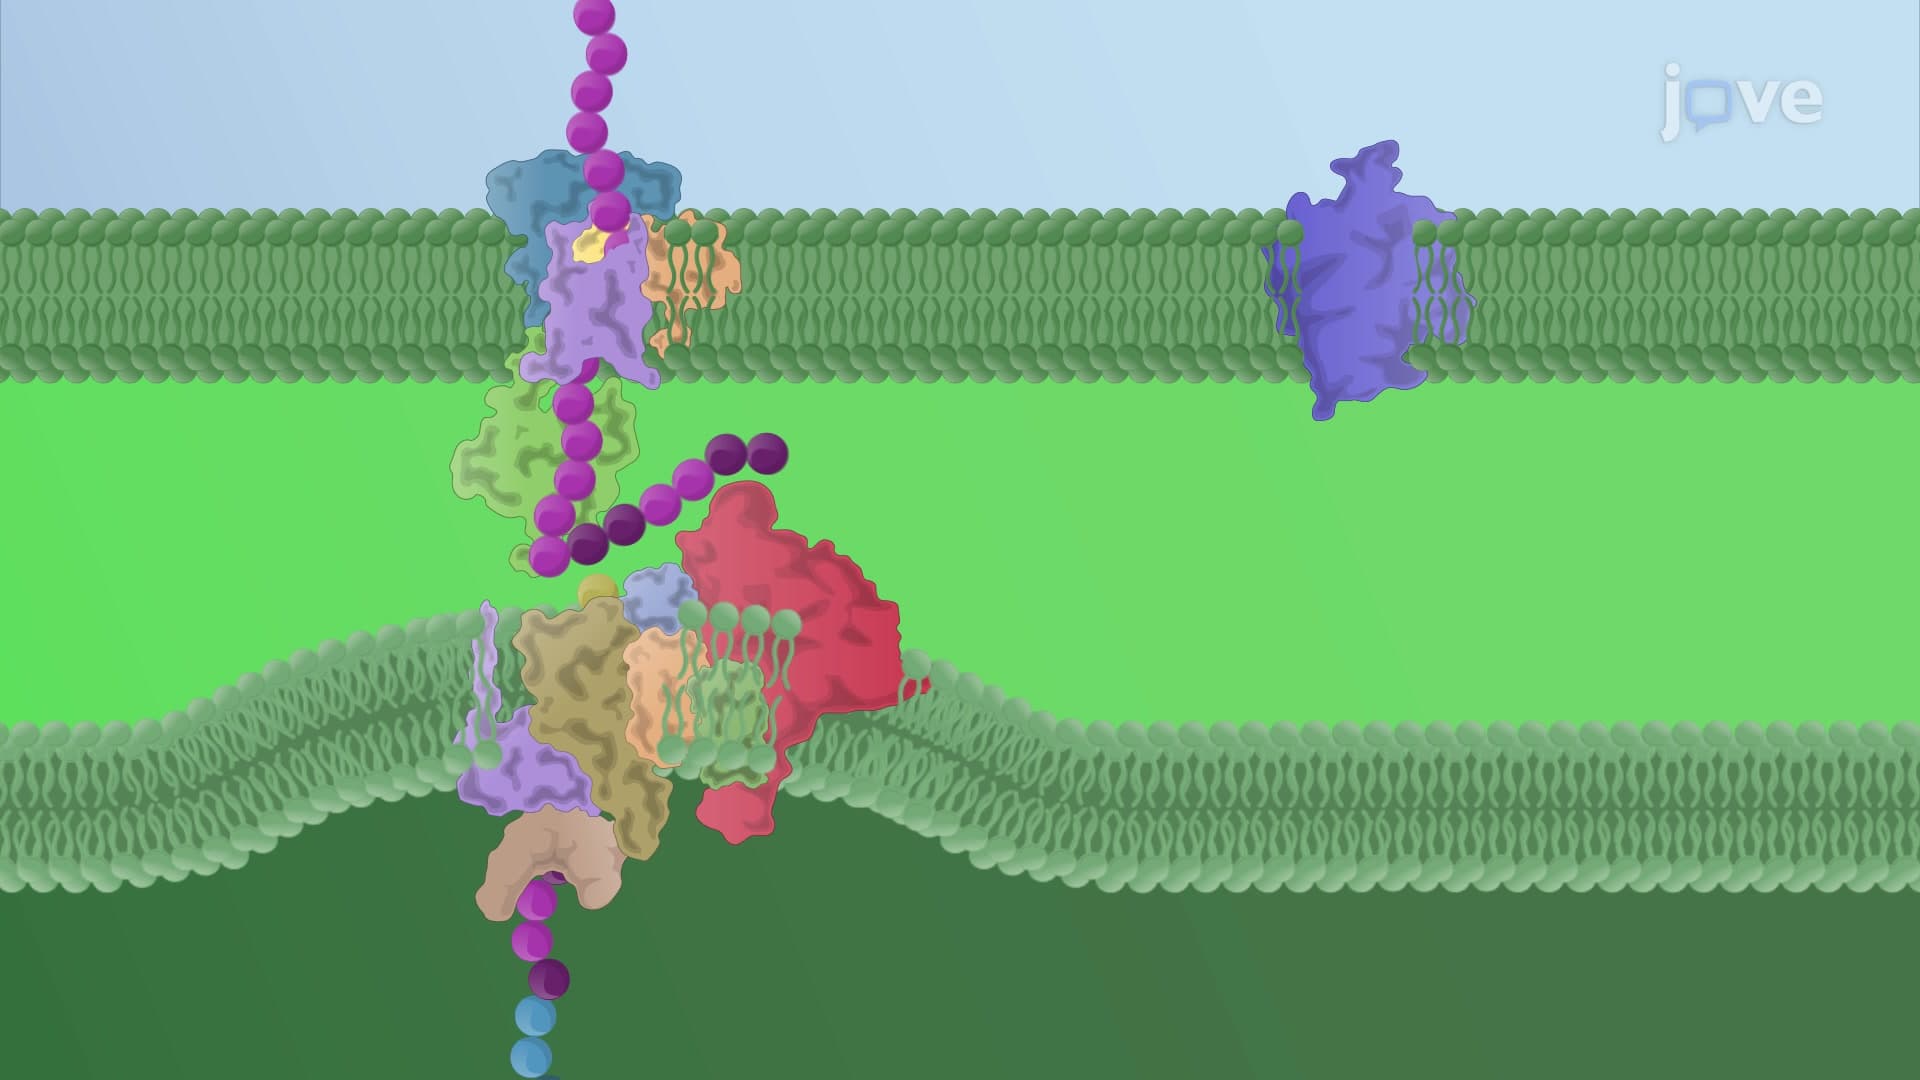
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.
 01:11
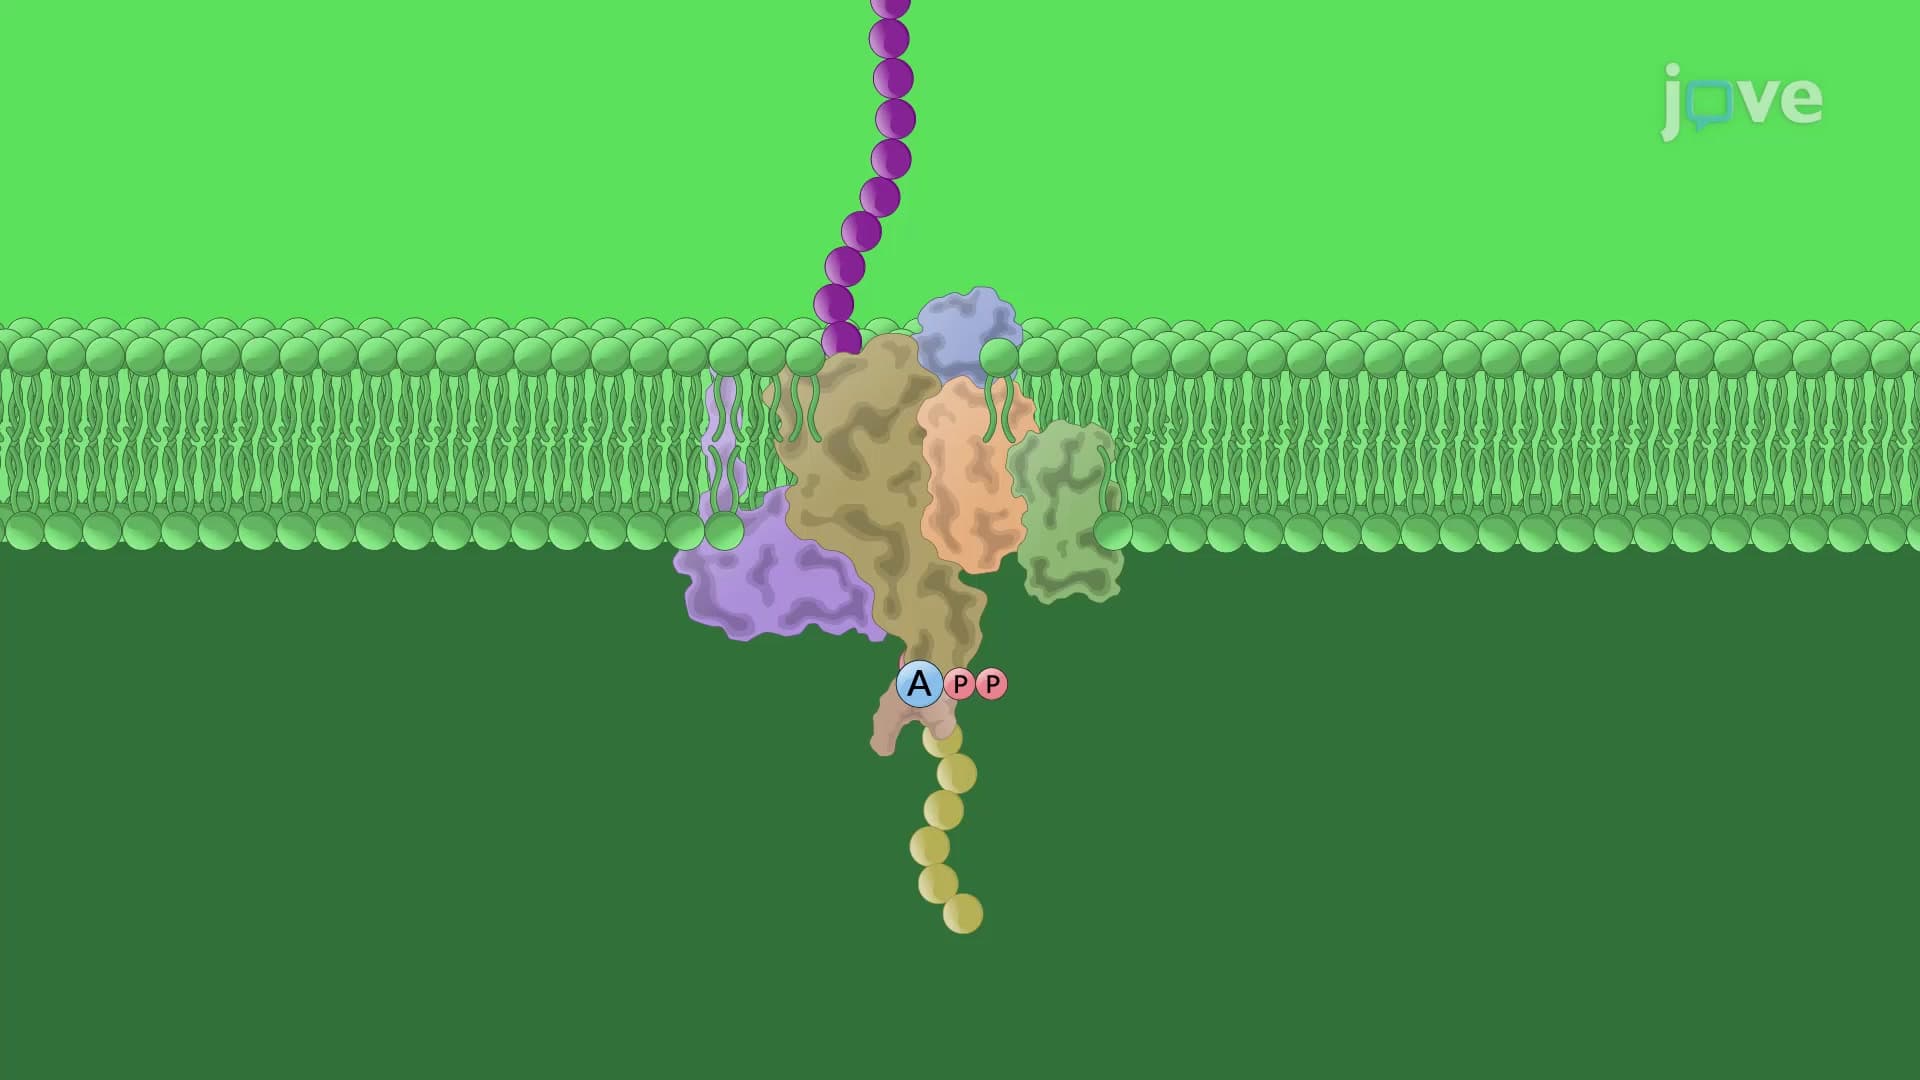
Protein Transport to the Outer Chloroplast Membrane
Two models describe the mechanism of precursor recognition and entry across the outer membrane through the TOC complex. Model 1 suggests the newly synthesized precursor binds to the TOC receptor 159 and forms a complex.
 01:39
Mitochondrial Protein Sorting
Most of these mitochondrial proteins are encoded by the nucleus and imported to the mitochondria as unfolded or loosely folded precursors. Mitochondrial precursors...
 01:22
Protein Transport to the Thylakoids
 01:24
Protein Transport to the Stroma
Protein complexes called the translocon of the outer chloroplast membrane or TOC complex, and the translocon of the inner chloroplast membrane or TIC complex mediate the...