
Remnant signal peptides on non-exported enzymes: implications for the evolution of prokaryotic respiratory chains
Bérengère Ize1, Sarah J Coulthurst2, Kostas Hatzixanthis1
1School of Biological Sciences, University of East Anglia, Norwich NR4 7TJ, UK.

Abstract:
The twin-arginine translocation (Tat) pathway is a prokaryotic protein targeting system dedicated to the transmembrane translocation of folded proteins. Substrate proteins are directed to the Tat translocase by signal peptides bearing a conserved SRRxFLK 'twin-arginine' motif. In Escherichia coli, most of the 27 periplasmically located Tat substrates are cofactor-containing respiratory enzymes, and many of these harbour a molybdenum cofactor at their active site. Molybdenum cofactor-containing proteins are not exclusively located in the periplasm, however, with the major respiratory nitrate reductase (NarG) and the biotin sulfoxide reductase (BisC), for example, being located at the cytoplasmic side of the membrane. Interestingly, both NarG and BisC contain 'N-tail' regions that bear some sequence similarity to twin-arginine signal peptides. In this work, we have examined the relationship between the non-exported N-tails and the Tat system. Using a sensitive genetic screen for Tat transport, variant N-tails were identified that displayed Tat transport activity. For the NarG 36-residue N-tail, six amino acid changes were needed to induce transport activity. However, these changes interfered with binding by the NarJ biosynthetic chaperone and impaired biosynthesis of the native enzyme. For the BisC 36-residue N-tail, only five amino acid substitutions were needed to restore Tat transport activity. These modifications also impaired in vivo BisC activity, but it was not possible to identify a biosynthetic chaperone for this enzyme. These data highlight an intimate genetic and evolutionary link between some non-exported redox enzymes and those transported across membranes by the Tat translocation system.
Related Concept Videos
 01:34
Directing Proteins to the Rough Endoplasmic Reticulum
 01:26
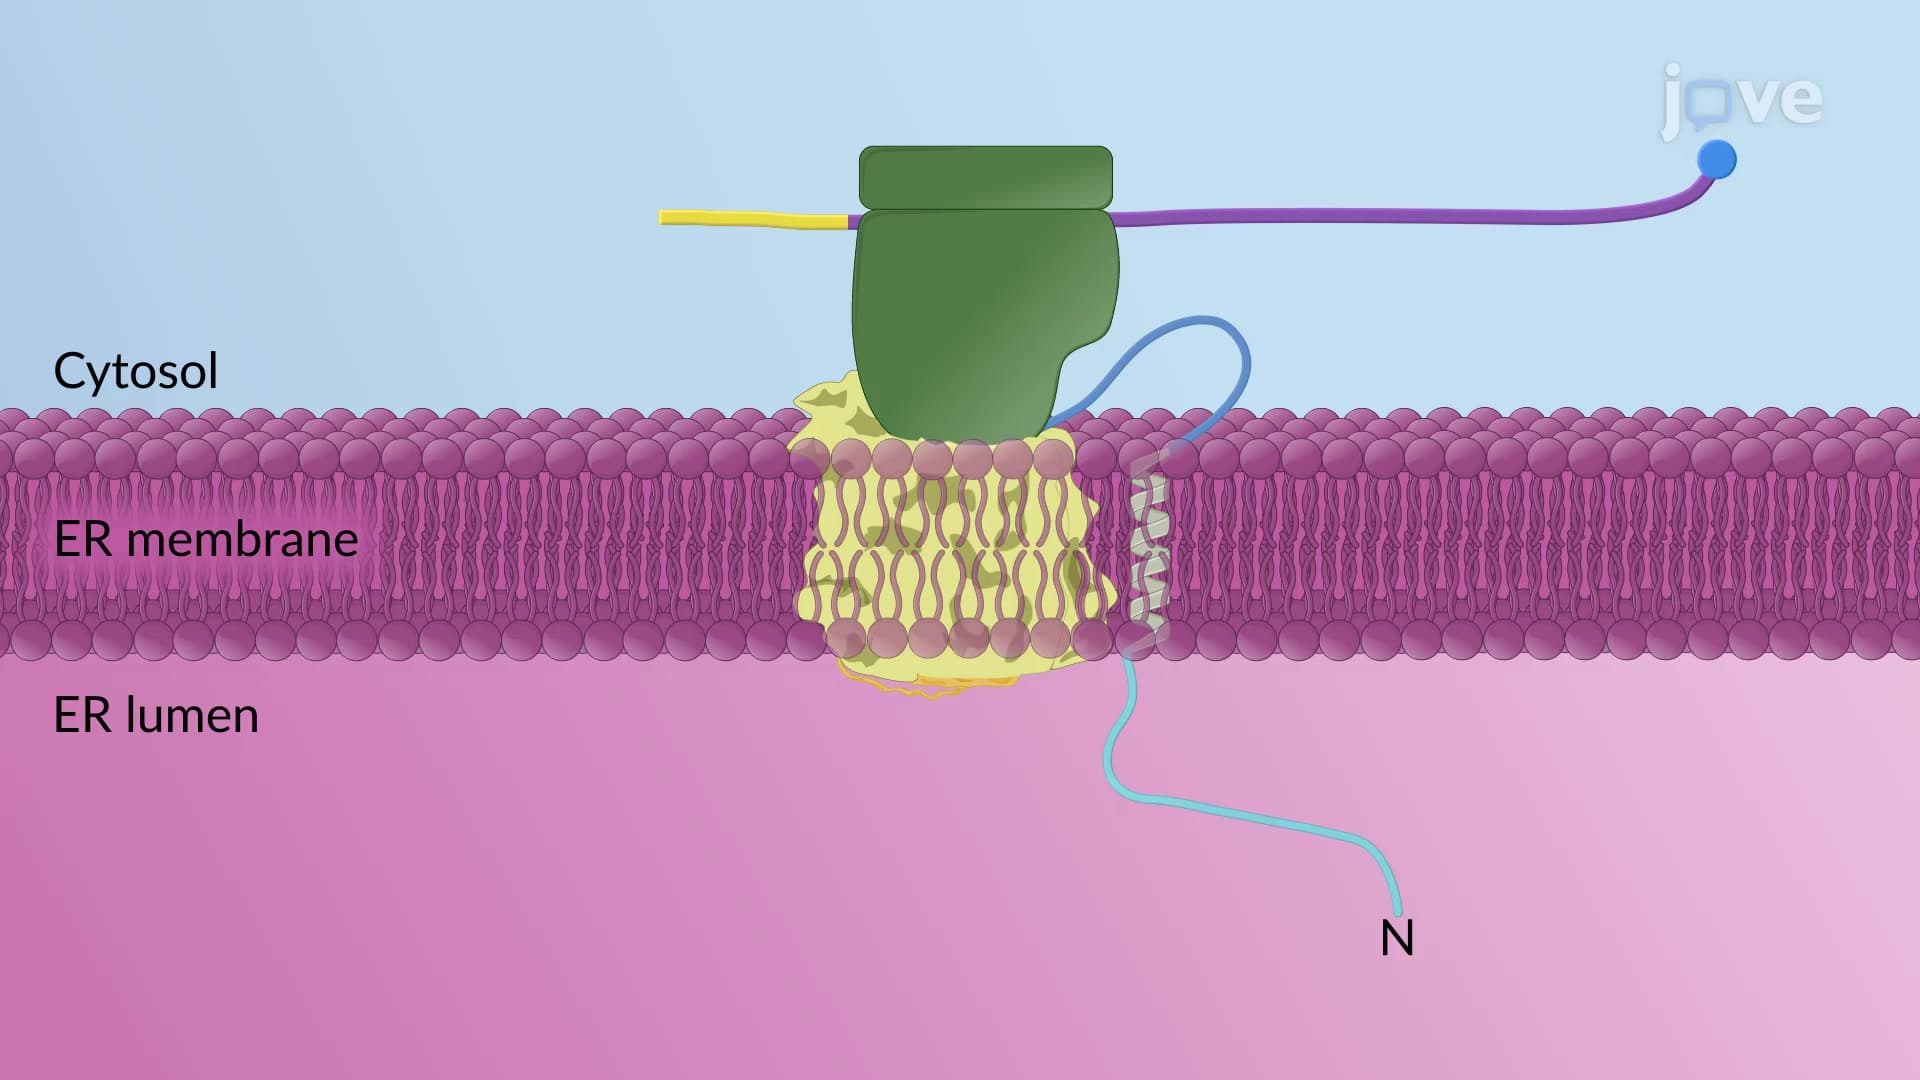
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...
 01:42
Nuclear Export
NES are of three types- the canonical 10-residue long leucine-rich signal and other...
 01:39
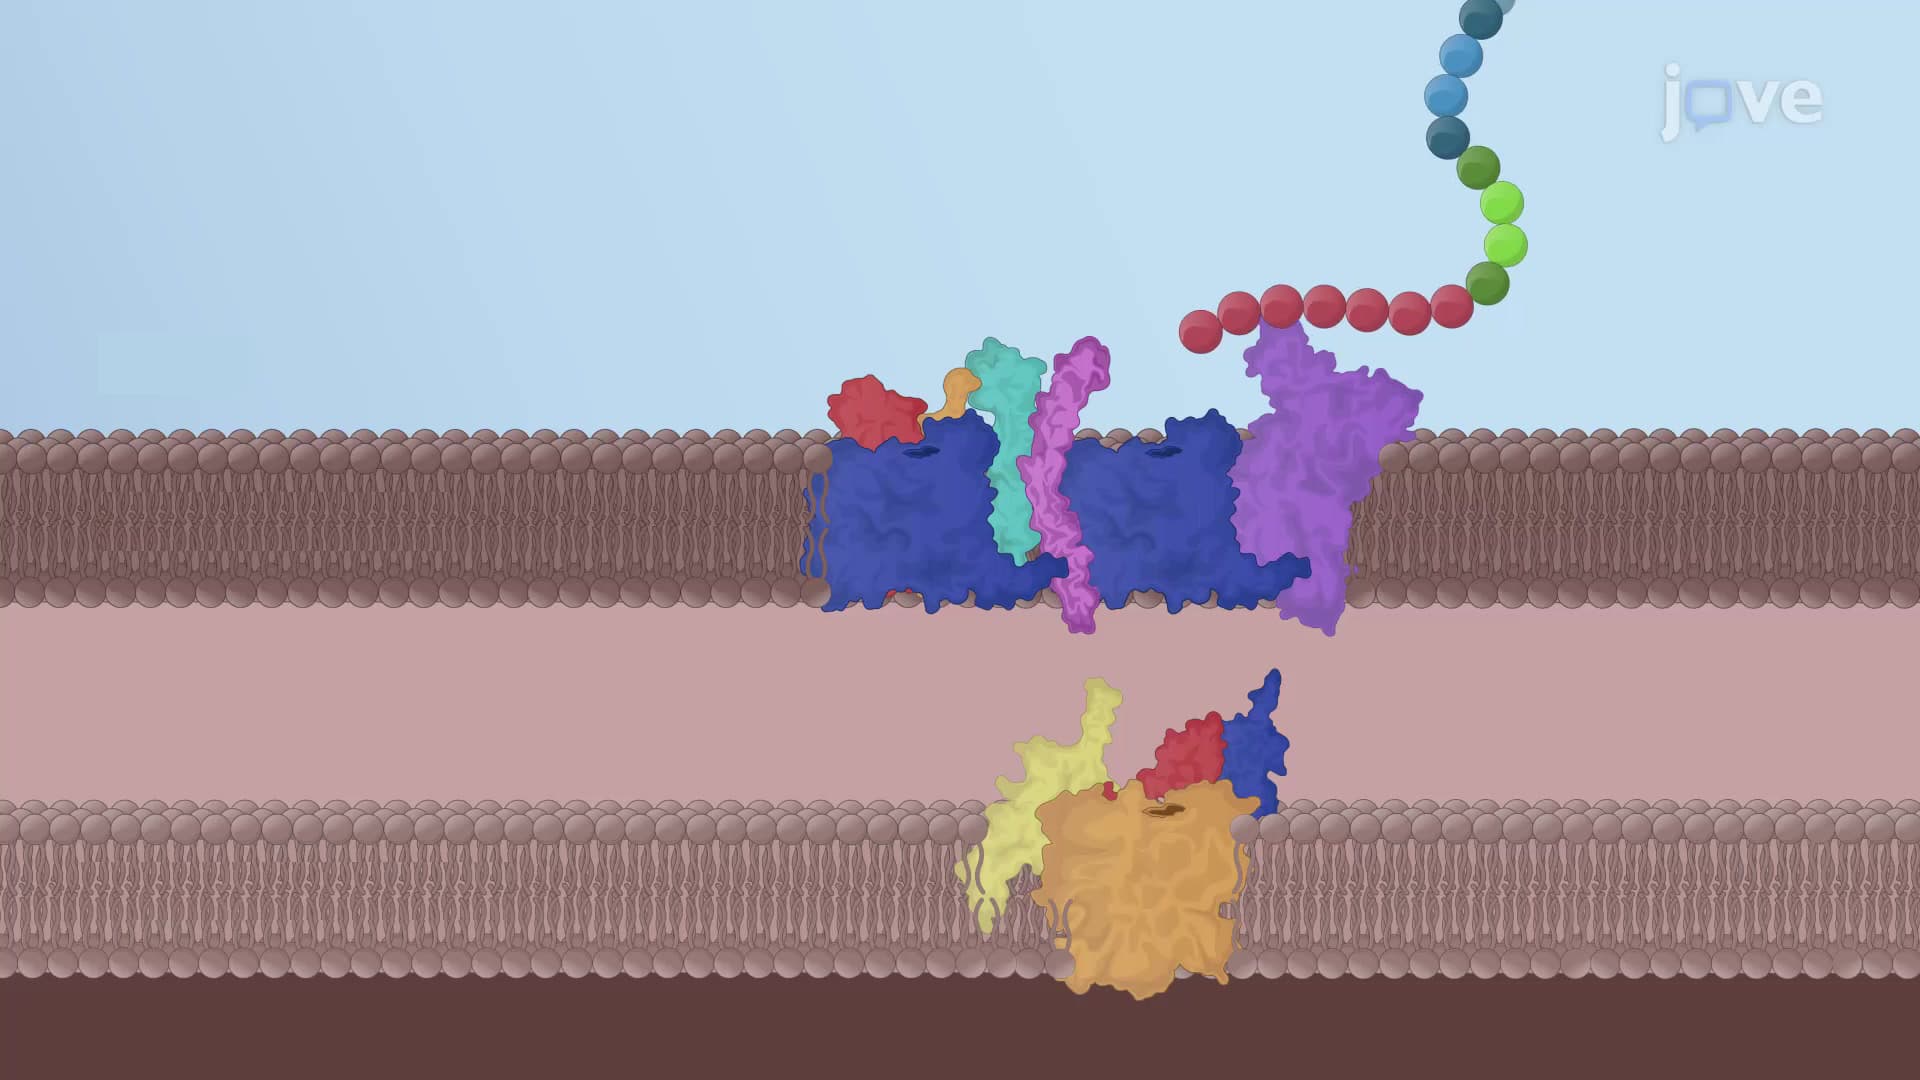
Mitochondrial Precursor Proteins
Most of the mitochondrial precursors...
 01:21
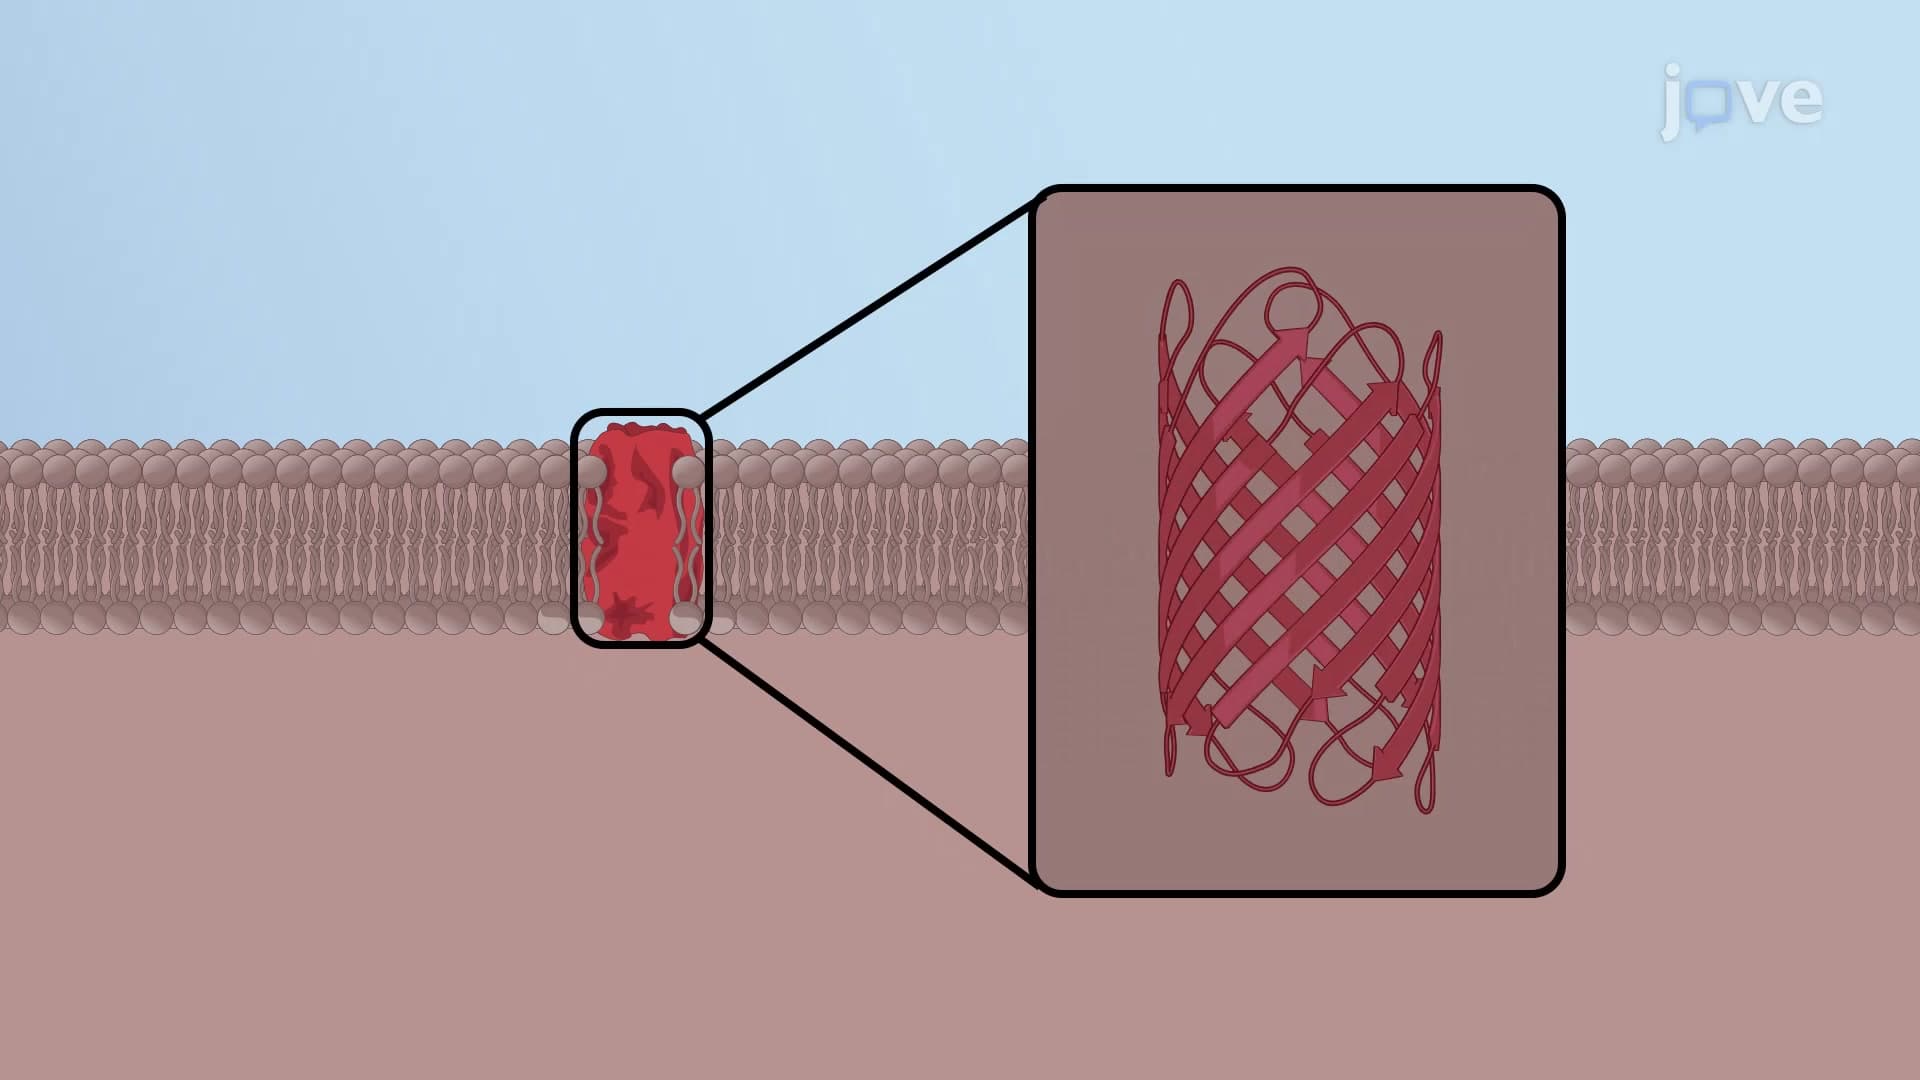
Structure of Porins
 01:27
Protein Import into the Peroxisomes
Peroxisomal Protein Import:
Peroxisomes lack the genetic machinery required to code for their own proteins. Hence, most peroxisomal membrane, lumenal and transmembrane proteins are synthesized in the cytoplasm or ER and transported to the peroxisome...