Backbone conformational flexibility of the lipid modified membrane anchor of the human N-Ras protein investigated by solid-state NMR and molecular dynamics simulation
Related Experiment Video
Updated: Jun 19, 2026
Method to Visualize and Analyze Membrane Interacting Proteins by Transmission Electron Microscopy
Published on: March 5, 2017
Alexander Vogel1, Guido Reuther, Matthew B Roark
1Junior Research Group Structural Biology of Membrane Proteins, Martin Luther University Halle-Wittenberg, Kurt-Mothes-Str. 3, D-06120 Halle, Germany. alexander.vogel@biochemtech.uni-halle.de

Abstract:
The lipid modified human N-Ras protein, implicated in human cancer development, is of particular interest due to its membrane anchor that determines the activity and subcellular location of the protein. Previous solid-state NMR investigations indicated that this membrane anchor is highly dynamic, which may be indicative of backbone conformational flexibility. This article aims to address if a dynamic exchange between three structural models exist that had been determined previously. We applied a combination of solid-state nuclear magnetic resonance (NMR) methods and replica exchange molecular dynamics (MD) simulations using a Ras peptide that represents the terminal seven amino acids of the human N-Ras protein. Analysis of correlations between the conformations of individual amino acids revealed that Cys 181 and Met 182 undergo collective conformational exchange. Two major structures constituting about 60% of all conformations could be identified. The two conformations found in the simulation are in rapid exchange, which gives rise to low backbone order parameters and nuclear spin relaxation as measured by experimental NMR methods. These parameters were also determined from two 300 ns conventional MD simulations, providing very good agreement with the experimental data.
Related Concept Videos
 00:52
¹H NMR of Conformationally Flexible Molecules: Temporal Resolution
 01:15
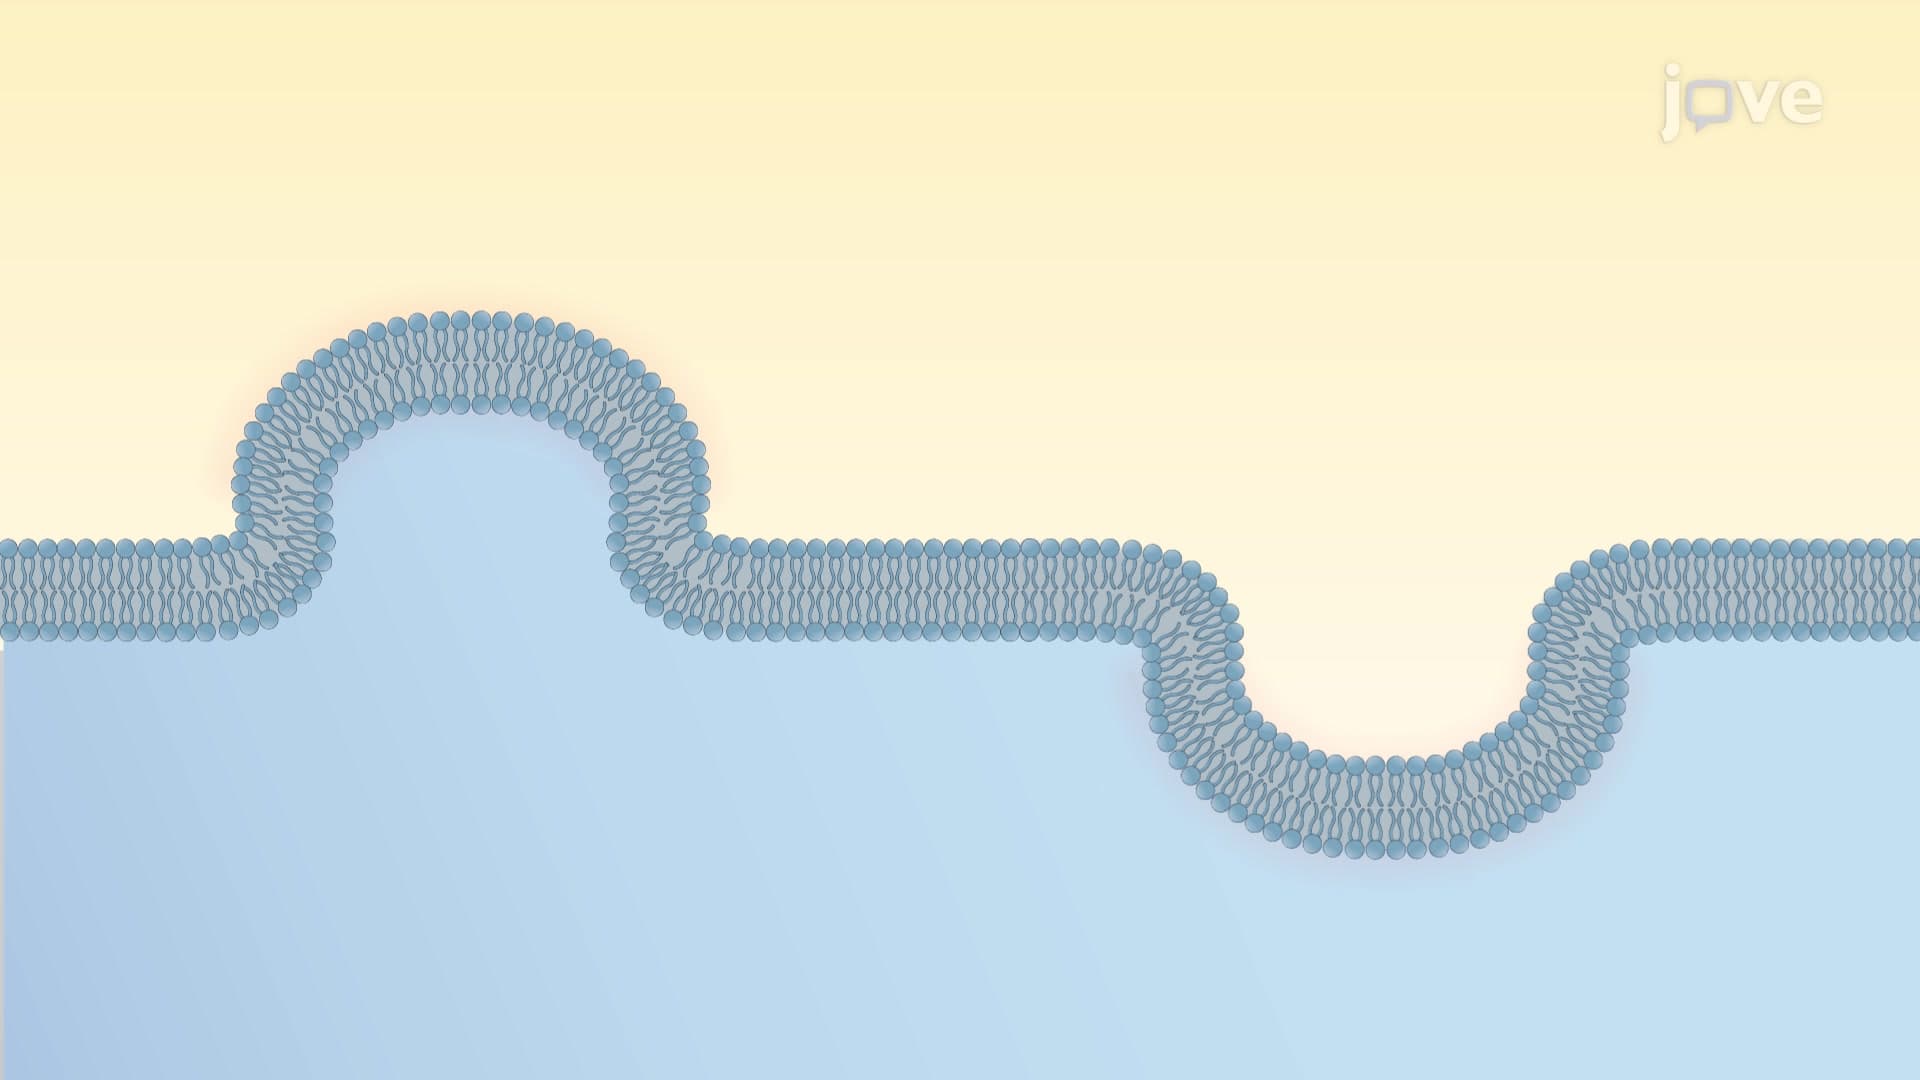
Mechanisms of Membrane-bending
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...
 01:32
Lipids as Anchors
The carboxy-terminal of most of the prenylated proteins, such as Ras proteins, contains the...
 01:15
¹H NMR of Conformationally Flexible Molecules: Variable-Temperature NMR
 01:26
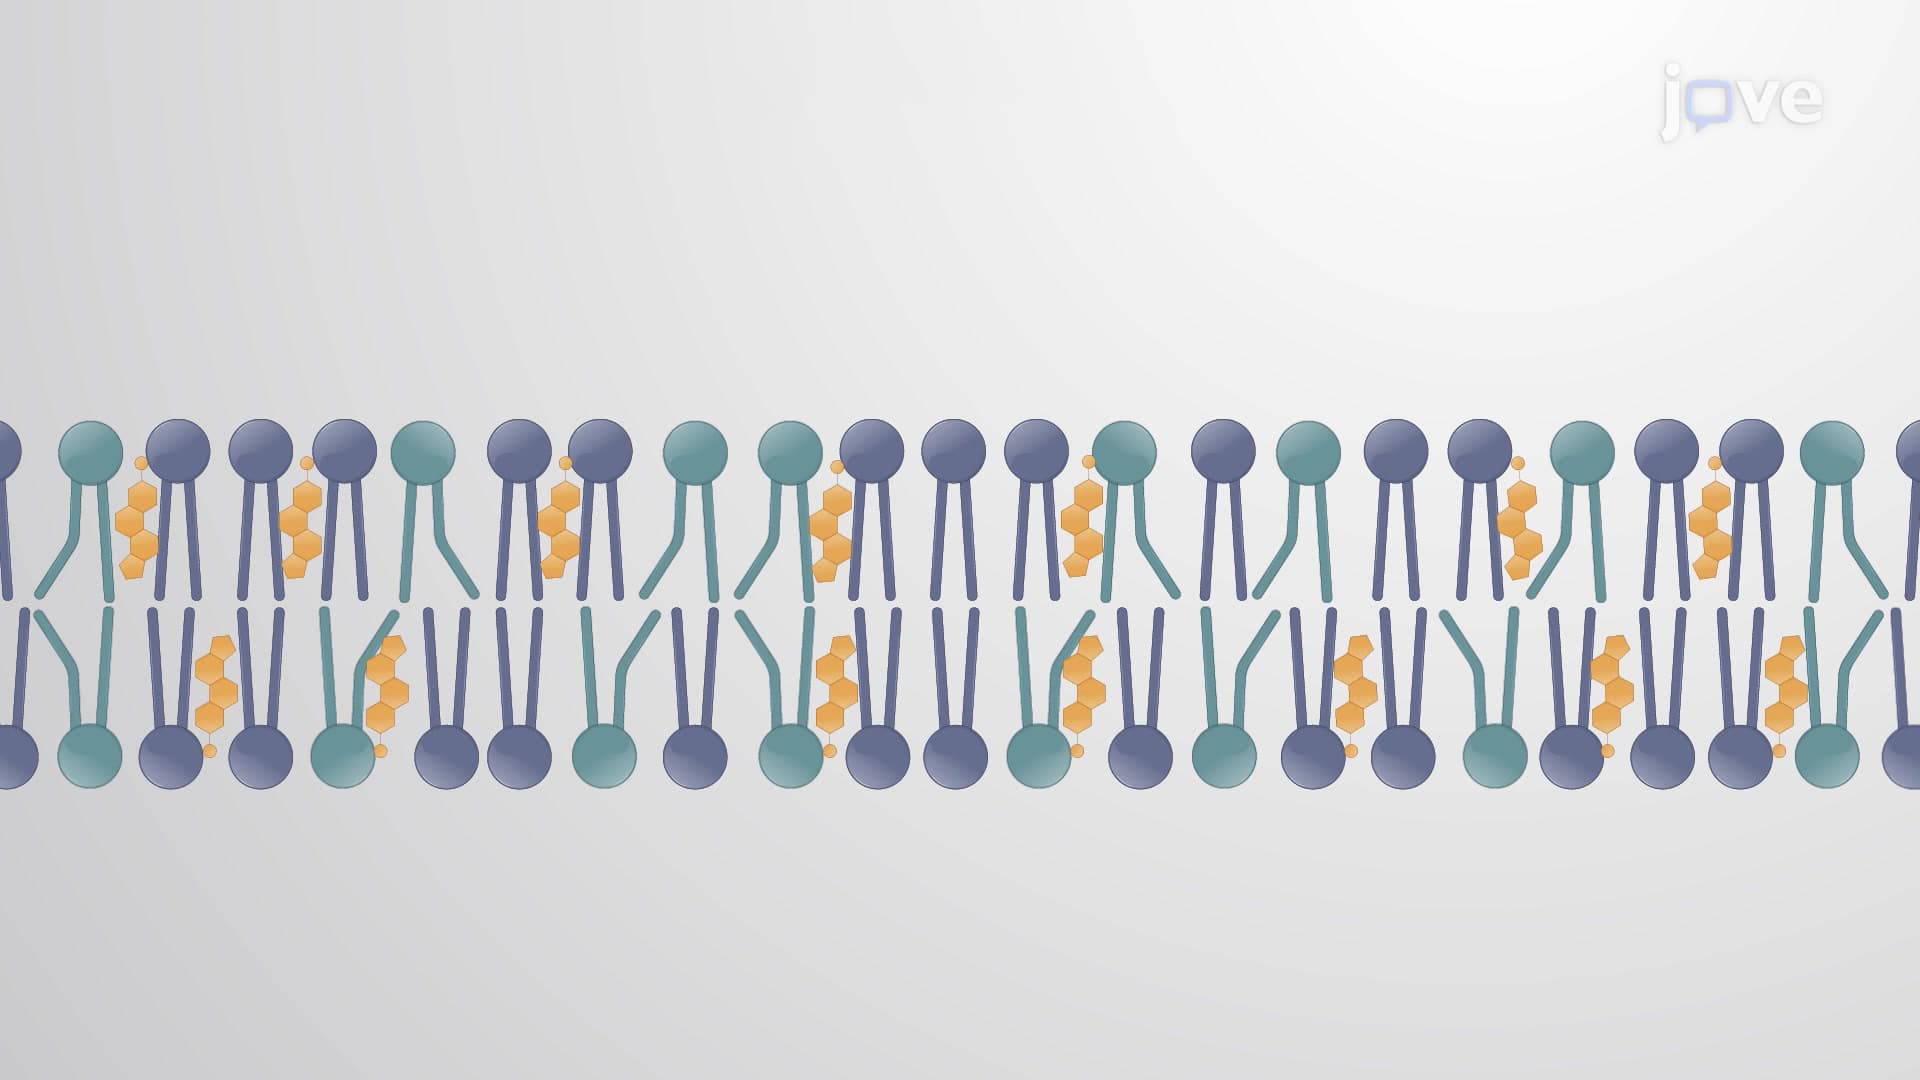
Membrane Fluidity
Mosaic nature of the membrane
The mosaic characteristic of the membrane helps the plasma membrane remain fluid. The integral proteins and lipids exist as separate but loosely-attached molecules in the membrane. The membrane is a relatively...
 01:45
Tail-anchoring of Proteins in the ER Membrane