Related Experiment Video
Updated: Jun 19, 2026

Helical Organization of Blood Coagulation Factor VIII on Lipid Nanotubes
Published on: June 3, 2014
The central portion of factor H (modules 10-15) is compact and contains a structurally deviant CCP module
Christoph Q Schmidt1, Andrew P Herbert, Haydyn D T Mertens
1Edinburgh Biomolecular NMR Unit, Centre for Chemical and Translational Biology, Schools of Biological Sciences and Chemistry, University of Edinburgh, Edinburgh EH9 3JJ, UK.

The first eight and the last two of 20 complement control protein (CCP) modules within complement factor H (fH) encompass binding sites for C3b and polyanionic carbohydrates. These binding sites cooperate self-surface selectively to prevent C3b amplification, thus minimising complement-mediated damage to host. Intervening fH CCPs, apparently devoid of such recognition sites, are proposed to play a structural role. One suggestion is that the generally small CCPs 10-15, connected by longer-than-average linkers, act as a flexible tether between the two functional ends of fH; another is that the long linkers induce a 180 degrees bend in the middle of fH. To test these hypotheses, we determined the NMR-derived structure of fH12-13 consisting of module 12, shown here to have an archetypal CCP structure, and module 13, which is uniquely short and features a laterally protruding helix-like insertion that contributes to a prominent electropositive patch. The unusually long fH12-13 linker is not flexible. It packs between the two CCPs that are not folded back on each other but form a shallow vee shape; analytical ultracentrifugation and X-ray scattering supported this finding. These two techniques additionally indicate that flanking modules (within fH11-14 and fH10-15) are at least as rigid and tilted relative to neighbours as are CCPs 12 and 13 with respect to one another. Tilts between successive modules are not unidirectional; their principal axes trace a zigzag path. In one of two arrangements for CCPs 10-15 that fit well with scattering data, CCP 14 is folded back onto CCP 13. In conclusion, fH10-15 forms neither a flexible tether nor a smooth bend. Rather, it is compact and has embedded within it a CCP module (CCP 13) that appears to be highly specialised given both its deviant structure and its striking surface charge distribution. A passive, purely structural role for this central portion of fH is unlikely.
The first eight and the last two of 20 complement control protein (CCP) modules within complement factor H (fH) encompass binding sites for C3b and polyanionic carbohydrates. These binding sites cooperate self-surface selectively to prevent C3b amplification, thus minimising complement-mediated damage to host. Intervening fH CCPs, apparently devoid of such recognition sites, are proposed to play a structural role. One suggestion is that the generally small CCPs 10-15, connected by longer-than-average linkers, act as a flexible tether between the two functional ends of fH; another is that the long linkers induce a 180 degrees bend in the middle of fH. To test these hypotheses, we determined the NMR-derived structure of fH12-13 consisting of module 12, shown here to have an archetypal CCP structure, and module 13, which is uniquely short and features a laterally protruding helix-like insertion that contributes to a prominent electropositive patch. The unusually long fH12-13 linker is not flexible. It packs between the two CCPs that are not folded back on each other but form a shallow vee shape; analytical ultracentrifugation and X-ray scattering supported this finding. These two techniques additionally indicate that flanking modules (within fH11-14 and fH10-15) are at least as rigid and tilted relative to neighbours as are CCPs 12 and 13 with respect to one another. Tilts between successive modules are not unidirectional; their principal axes trace a zigzag path. In one of two arrangements for CCPs 10-15 that fit well with scattering data, CCP 14 is folded back onto CCP 13. In conclusion, fH10-15 forms neither a flexible tether nor a smooth bend. Rather, it is compact and has embedded within it a CCP module (CCP 13) that appears to be highly specialised given both its deviant structure and its striking surface charge distribution. A passive, purely structural role for this central portion of fH is unlikely.
Related Concept Videos
 01:57
Protein Complexes with Interchangeable Parts
The SCF ubiquitin ligase is a protein complex of five individual proteins. This complex attaches ubiquitin to other target proteins to mark them for degradation. In order to...
01:57Protein Complexes with Interchangeable Parts
The SCF ubiquitin ligase is a protein complex of five individual proteins. This complex attaches ubiquitin to other target proteins to mark them for degradation. In order to...
 01:22
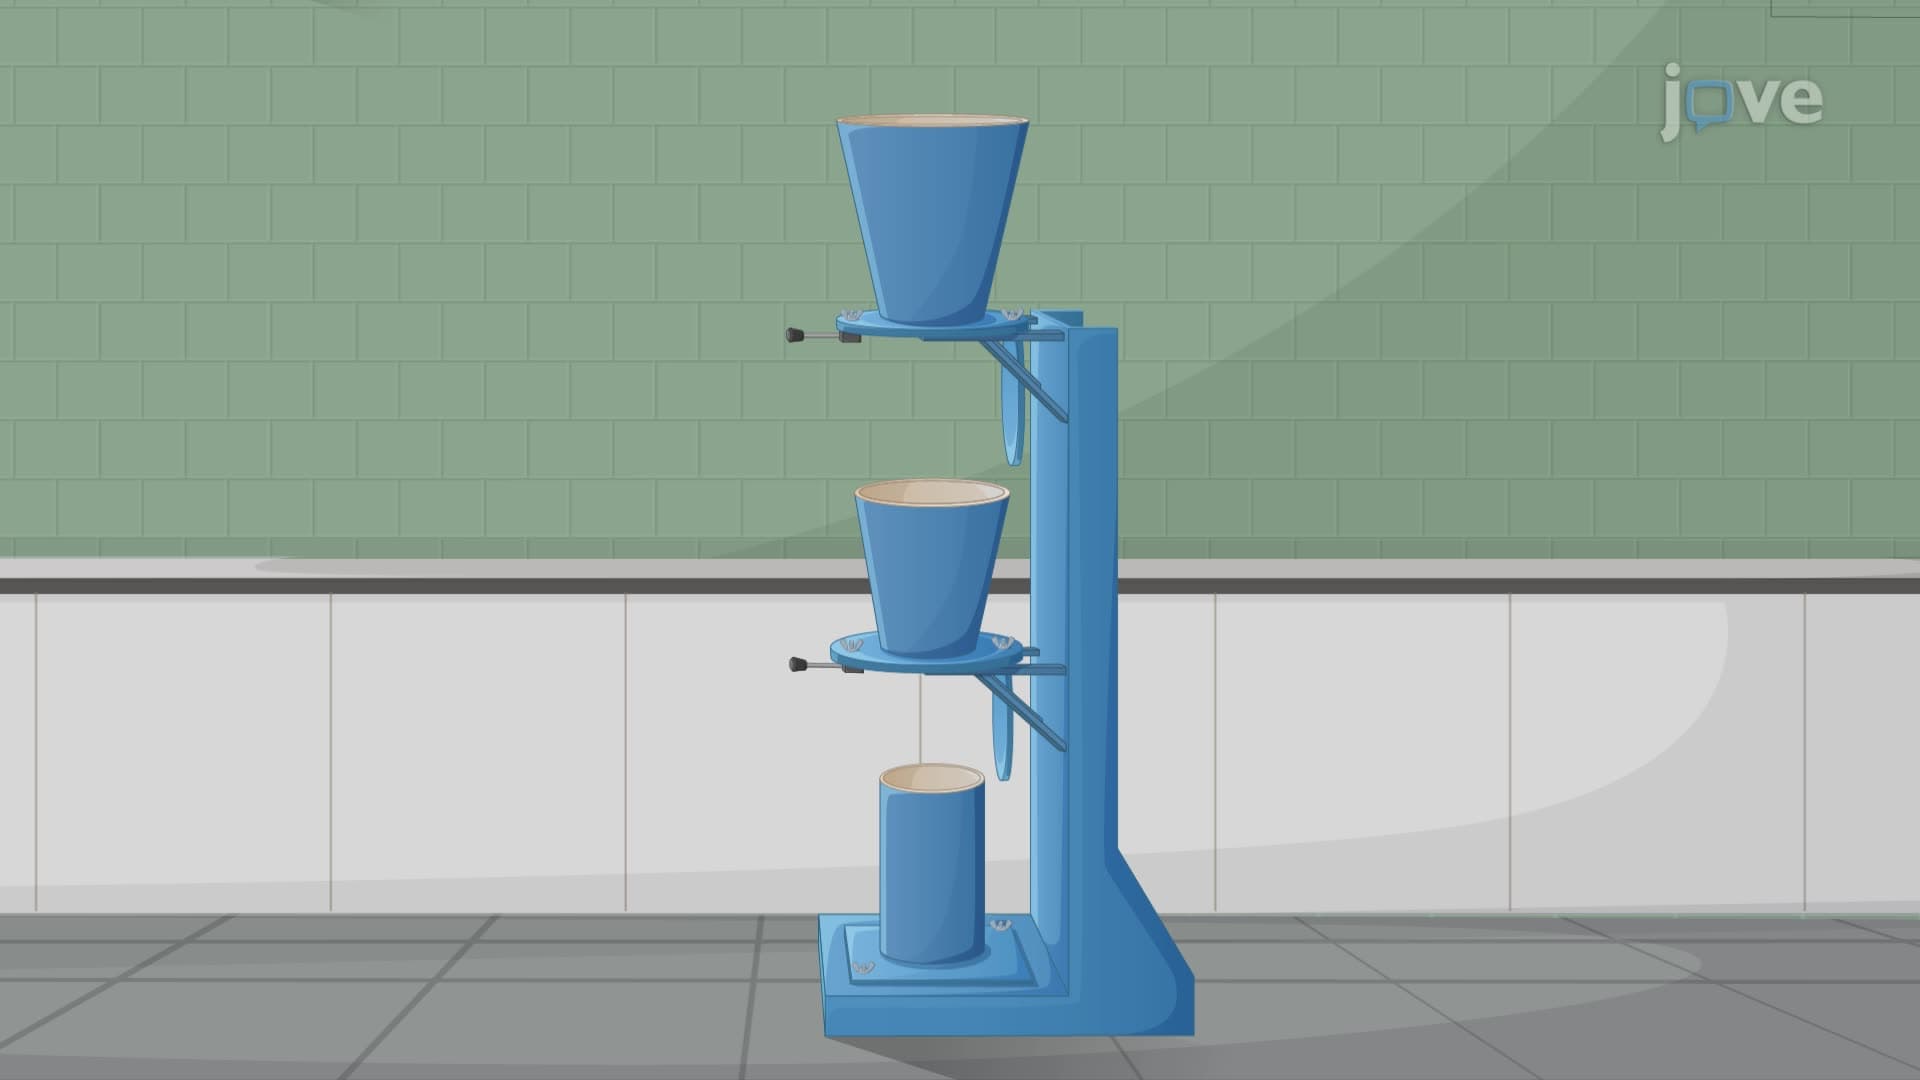
Compacting Factor test
The procedure begins by placing concrete into the upper hopper without any compaction. Once filled, the bottom door of this hopper is opened,...
 02:33
Lattice Centering and Coordination Number
Types of Unit Cells
Imagine taking a large number of identical...
 02:04
Covalently Linked Protein Regulators
These groups modify specific amino acids in a protein.
02:04Covalently Linked Protein Regulators
These groups modify specific amino acids in a protein.