Related Experiment Video
Updated: Jun 19, 2026

Exploring Sequence Space to Identify Binding Sites for Regulatory RNA-Binding Proteins
Published on: August 9, 2019
The hinge domain of the cleavage stimulation factor protein CstF-64 is essential for CstF-77 interaction, nuclear
J Andrew Hockert1, Hsiang-Jui Yeh, Clinton C MacDonald
1Department of Cell Biology and Biochemistry, Texas Tech University Health Sciences Center, Lubbock, Texas 79430-6540, USA.

Abstract:
Because polyadenylation is essential for cell growth, in vivo examination of polyadenylation protein function has been difficult. Here we describe a new in vivo assay that allows structure-function assays on CstF-64, a protein that binds to pre-mRNAs downstream of the cleavage site for accurate and efficient polyadenylation. In this assay (the stem-loop luciferase assay for polyadenylation, SLAP), expression of a luciferase pre-mRNA with a modified downstream sequence element was made dependent upon co-expression of an MS2-CstF-64 fusion protein. We show here that SLAP accurately reflects CstF-64-dependent polyadenylation, confirming the validity of this assay. Using SLAP, we determined that CstF-64 domains involved in RNA binding, interaction with CstF-77 (the "Hinge" domain), and coupling to transcription are critical for polyadenylation. Further, we showed that the Hinge domain is necessary for CstF-64 interaction with CstF-77 and consequent nuclear localization, suggesting that nuclear import of a preformed CstF complex is an essential step in polyadenylation.
Related Concept Videos
 01:45
Regulation of Nuclear Protein Sorting
 01:20
Cotranslational Protein Translocation
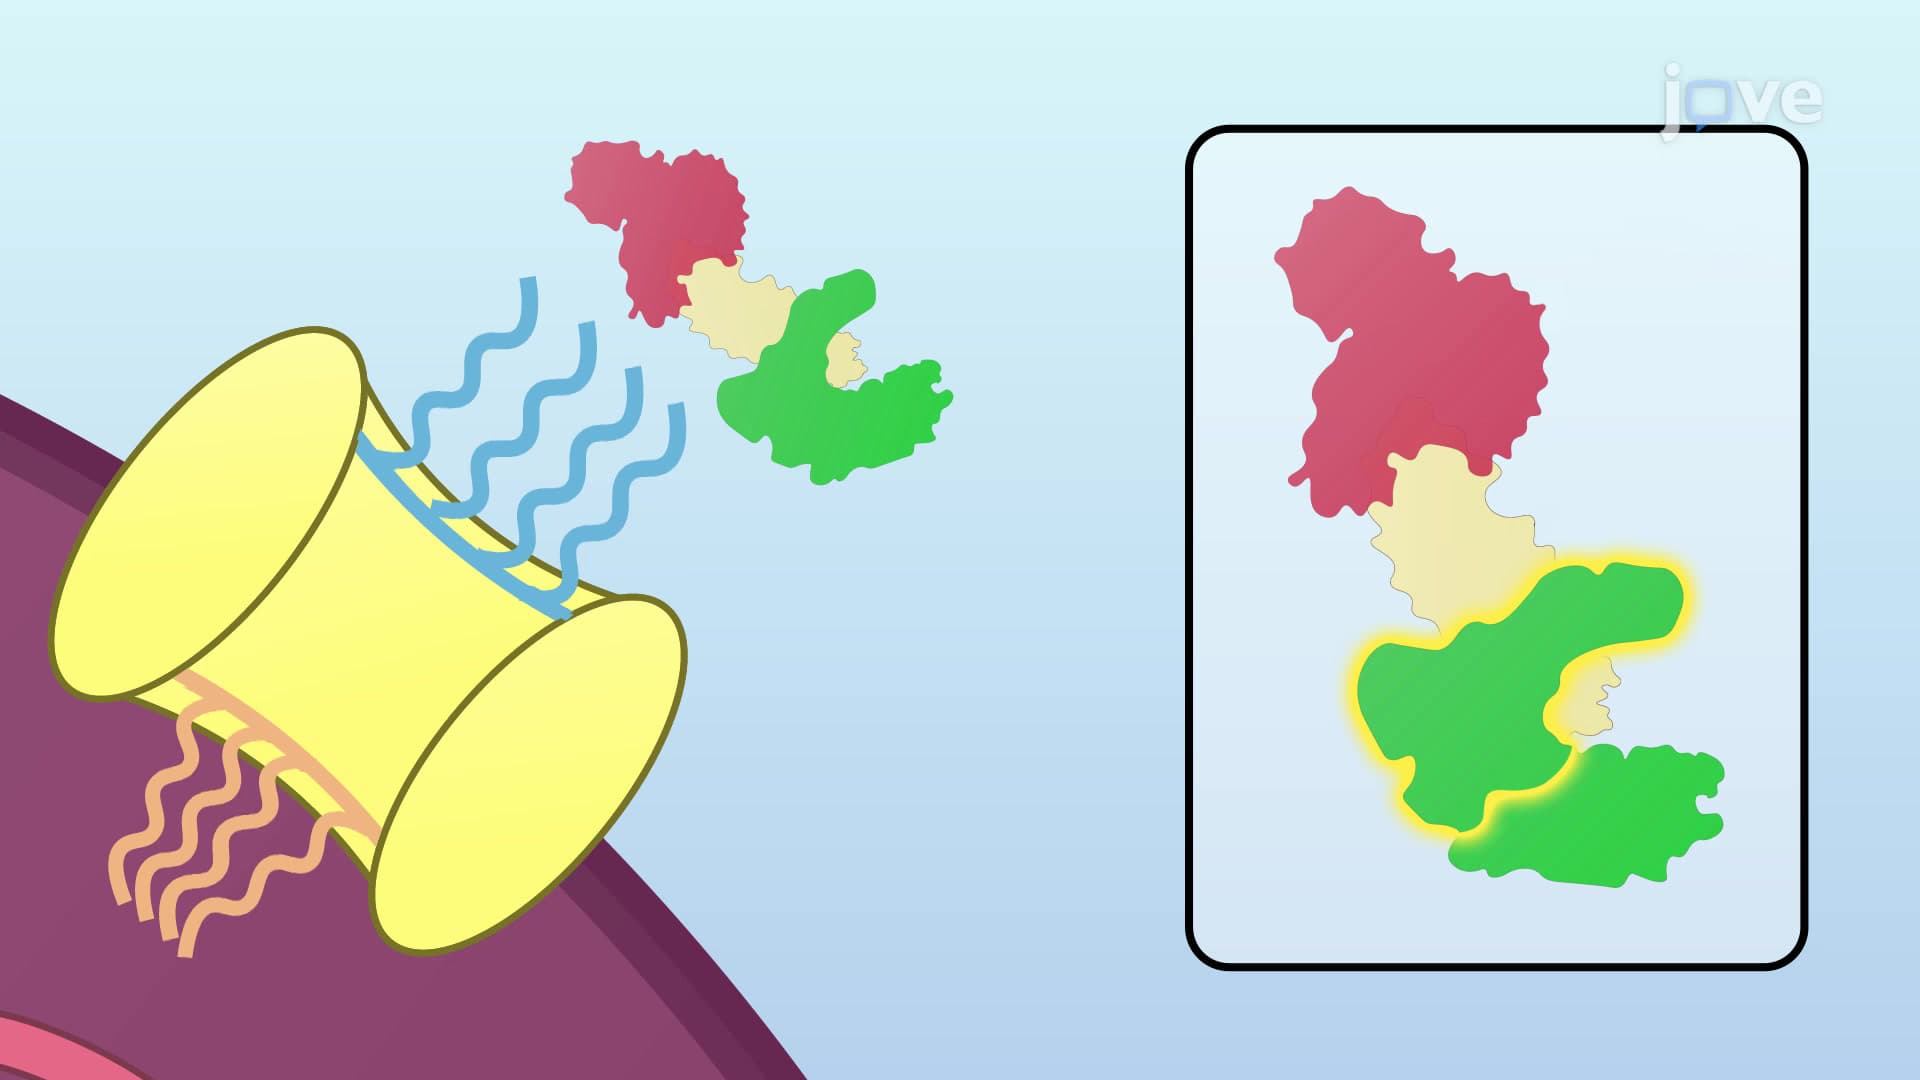
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
 01:46
Nuclear Localization Signals and Import
 01:45
Tail-anchoring of Proteins in the ER Membrane
 01:33
Coat Assembly and GTPases
Coat assembly depends on the local availability of phosphatidylinositol phosphates or PIPs and GTP-binding proteins. Adaptor proteins, which link the coat proteins to the membrane, bind to these PIPs and play a crucial role in controlling...
 01:30
Assembly of Signaling Complexes
Interaction domains in cell signaling
Interaction domains recognize exposed features of their binding partners containing post-translationally modified sequences,...