Related Experiment Video
Updated: Jun 17, 2026

Evaluation of Exon Inclusion Induced by Splice Switching Antisense Oligonucleotides in SMA Patient Fibroblasts
Published on: May 11, 2018
Alternatively spliced N-terminal exons in tropomyosin isoforms do not act as autonomous targeting signals
Claire Martin1, Galina Schevzov, Peter Gunning
1Oncology Research Unit, School of Medical Sciences, University of New South Wales, Sydney, NSW 2052, Australia.

Abstract:
Tropomyosin (Tm) polymerises head-to-tail to form a continuous polymer located in the major groove of the actin filament. Multiple Tm isoforms are generated by alternative splicing of four genes, and individual isoforms show specific localisation patterns in many cell types, and can have differing effects on the actin cytoskeleton. Fluorescently-tagged Tm isoforms and mutants were expressed in C2C12 cells to investigate the mechanisms of alternative localisation of high molecular weight (HMW) and low molecular weight (LMW) Tms. Fluorescently-tagged Tm constructs show similar localisation to endogenous Tms as observed by antibodies, with the HMW Tm3 relatively diminished at the periphery of cells compared to LMW isoforms Tm5b or Tm5NM1. Tm3 and Tm5b only differ in their N-terminal exons, but these N-terminal exons do not independently direct localisation within the cell, as chimeric mutants Tm3-Tm5NM1 and Tm5b-Tm5NM1 show an increased peripheral localisation similar to Tm5NM1. The lower abundance of Tm3 at the periphery of the cell is not a result of different protein dynamics, as Tm3 and Tm5b show similar recovery after photobleaching. The relative exclusion of Tm3 from the periphery of cells does, however, require interaction with the actin filament, as mutants with truncations at either the N-terminus or the C-terminus are unable to localise to actin stress fibres, and are present in the most peripheral regions of the cell. We conclude that it is the entire Tm molecule which is the unit of sorting, and that the alternatively spliced N-terminal exons do not act as autonomous targeting signals.
Related Concept Videos
 02:18
Alternative RNA Splicing
There are five types of alternative RNA splicing that vary in the ways the pre-mRNA segments are removed or retained in the mature mRNA. The first...
 01:19
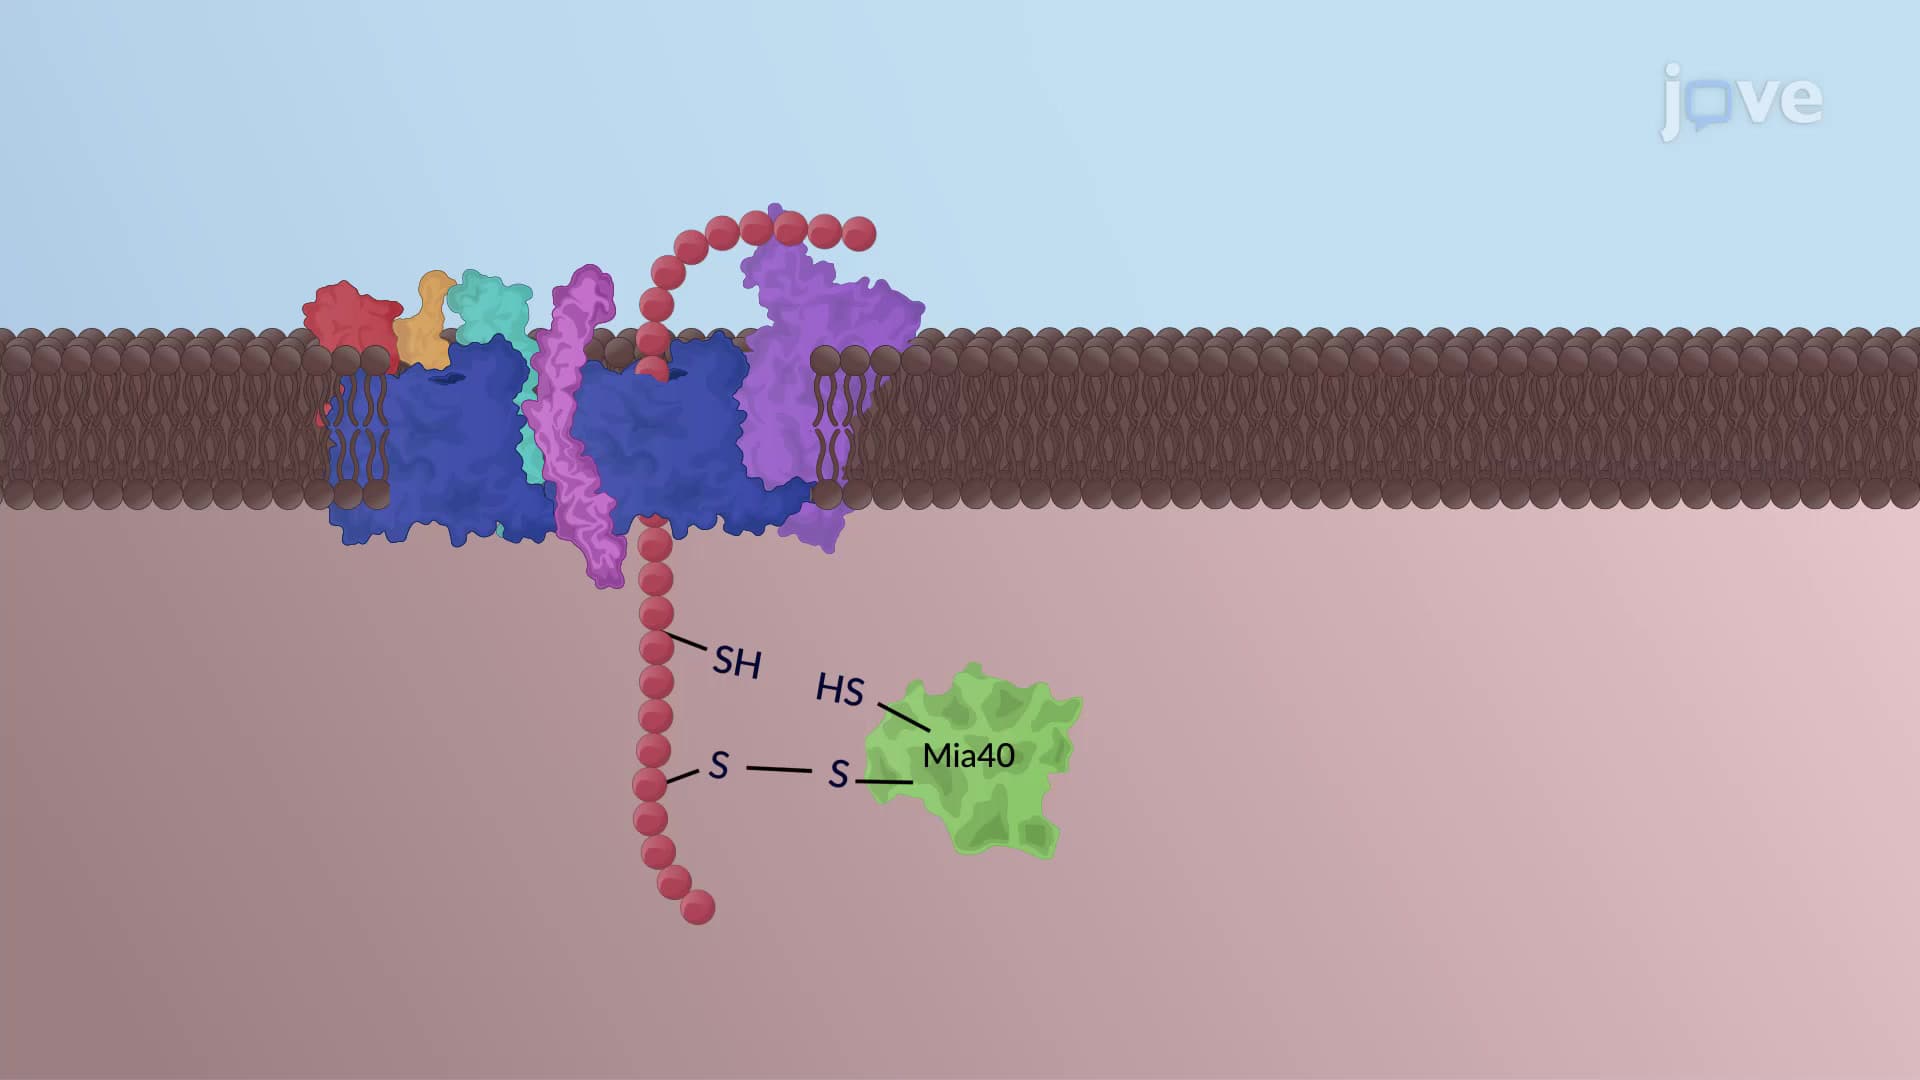
Translocation of Proteins into the Mitochondria
Sorting of outer membrane proteins:
Mitochondrial outer membrane proteins are of two types: the transmembrane, beta-barrel porins, and the membrane-anchored, alpha-helical proteins. Beta-barrel porin precursors are translocated by the TOM complex and inserted into the outer mitochondrial membrane by the SAM complex. In contrast,...
 01:32
RNA Splicing
 03:18
Non-LTR Retrotransposons
 02:27
Nonsense-mediated mRNA Decay
Usually, Upf3 binds to an Exon Junction Complex (EJC) at mRNA splice sites. If a ribosome fully translates the mRNA,...
 01:45
Tail-anchoring of Proteins in the ER Membrane