Related Experiment Video
Updated: Jun 17, 2026
Prospecting Microbial Strains for Bioremediation and Probiotics Development for Metaorganism Research and Preservation
Published on: October 31, 2019
Pathways and substrate specificity of DMSP catabolism in marine bacteria of the Roseobacter clade
Jeroen S Dickschat1, Claudia Zell, Nelson L Brock
1Institute of Organic Chemistry, Technical University of Braunschweig, Hagenring 30, 38106 Braunschweig, Germany. j.dickschat@tu-bs.de

Abstract:
The volatiles released by Phaeobacter gallaeciensis, Oceanibulbus indolifex and Dinoroseobacter shibae have been investigated by GC-MS, and several MeSH-derived sulfur volatiles have been identified. An important sulfur source in the oceans is the algal metabolite dimethylsulfoniopropionate (DMSP). Labelled [2H6]DMSP was fed to the bacteria to investigate the production of volatiles from this compound through the lysis pathway to [2H6]dimethylsulfide or the demethylation pathway to [2H3]-3-(methylmercapto)propionic acid and lysis to [2H3]MeSH. [2H6]DMSP was efficiently converted to [2H3]MeSH by all three species. Several DMSP derivatives were synthesised and used in feeding experiments. Strong dealkylation activity was observed for the methylated ethyl methyl sulfoniopropionate and dimethylseleniopropionate, as indicated by the formation of EtSH- and MeSeH-derived volatiles, whereas no volatiles were formed from dimethyltelluriopropionate. In contrast, the dealkylation activity for diethylsulfoniopropionate was strongly reduced, resulting in only small amounts of EtSH-derived volatiles accompanied by diethyl sulfide in P. gallaeciensis and O. indolifex, while D. shibae produced the related oxidation product diethyl sulfone. The formation of diethyl sulfide and diethyl sulfone requires the lysis pathway, which is not active for [2H6]DMSP. These observations can be explained by a shifted distribution between the two competing pathways due to a blocked dealkylation of ethylated substrates.
Related Concept Videos
 01:18
Deep Sea Microbial Ecology
 01:30
Marine Microbial Ecology
 01:29
Microbes and the Sulfur Cycle
 01:25
Lipid Catabolism
 01:28
Carbon-dioxide Fixation
 01:24
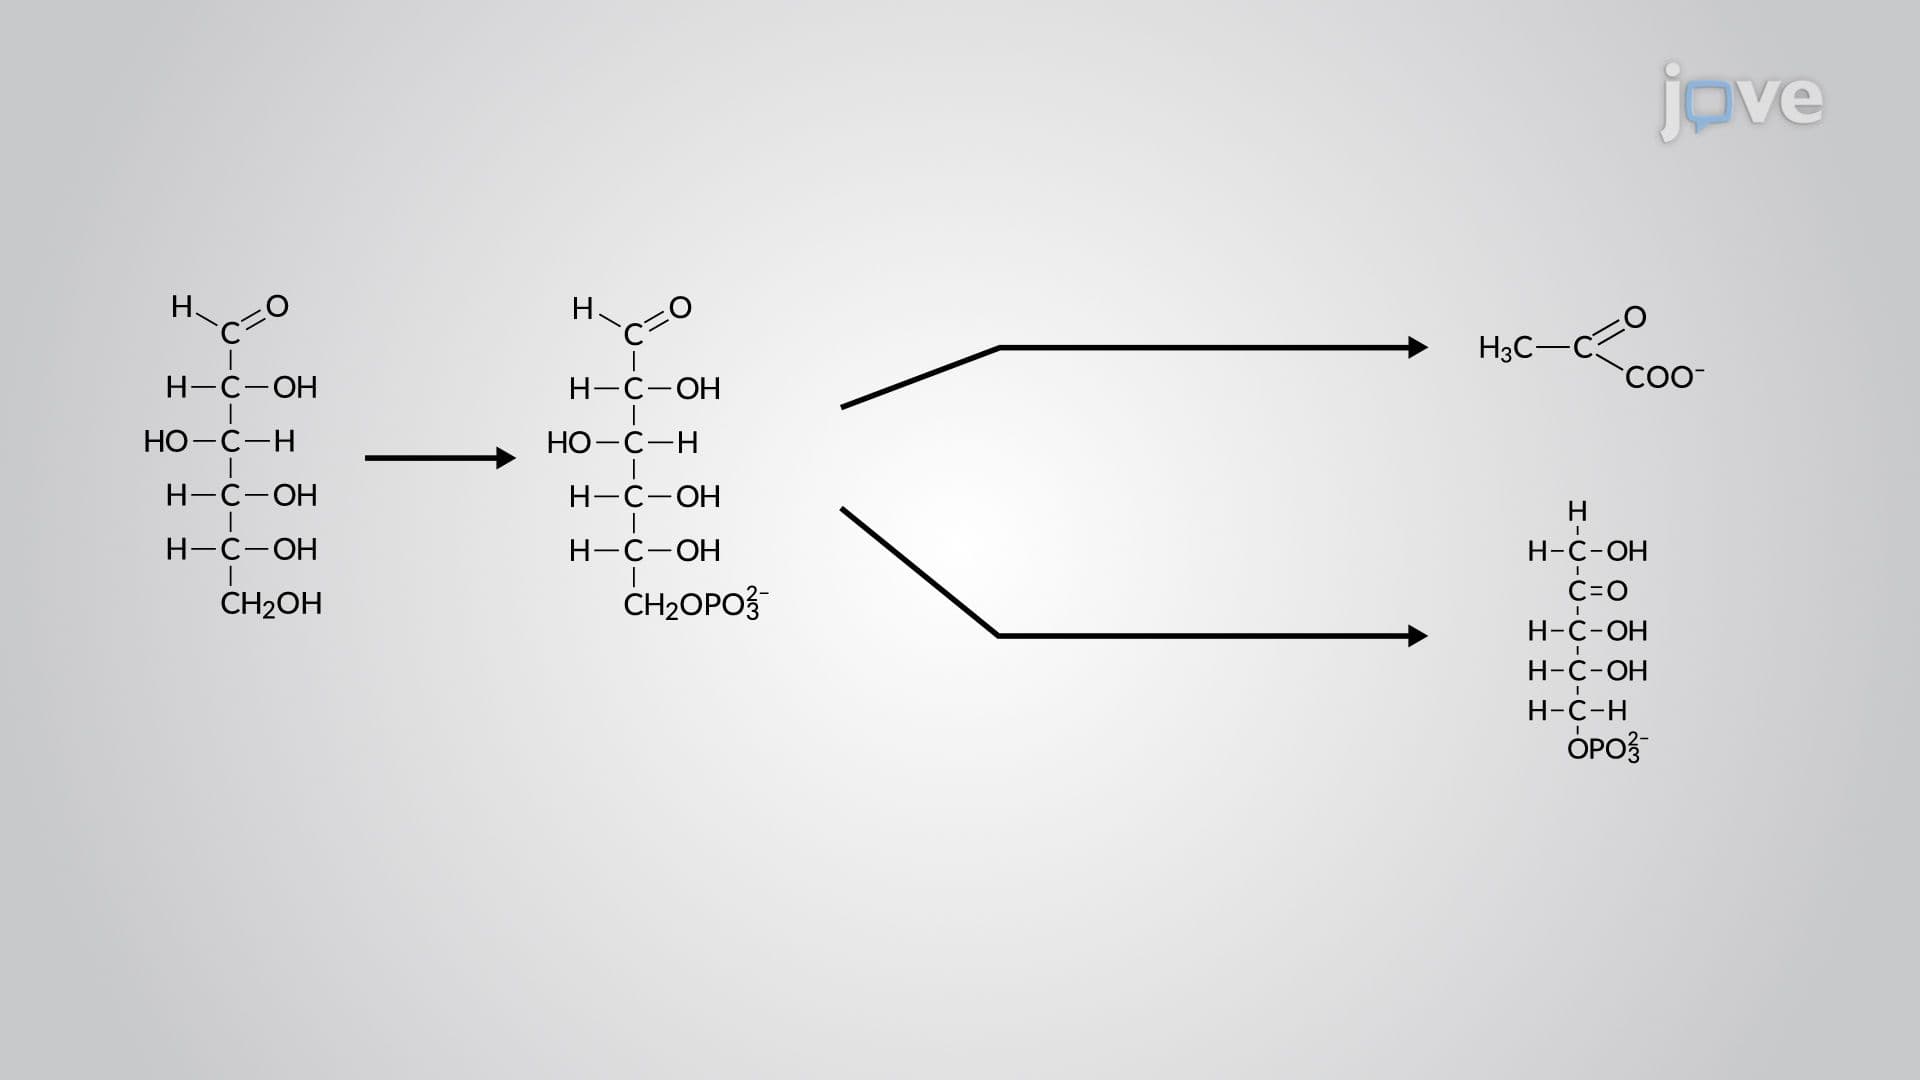
Other Glycolytic Pathways