
Molecular recognition of vesicles: host-guest interactions combined with specific dimerization of zwitterions
Jens Voskuhl1, Tassilo Fenske, Marc C A Stuart
1Organic Chemistry Institute, Westfälische Wilhelms-Universität Münster, Corrensstrasse 40, 48149 Münster, Germany.

Abstract:
The aggregation of beta-cyclodextrin vesicles can be induced by an adamantyl-substituted zwitterionic guanidiniocarbonylpyrrole carboxylate guest molecule (1). Upon addition of 1 to the cyclodextrin vesicles at neutral pH, the vesicles aggregate (but do not fuse), as shown by using UV/Vis and fluorescence spectroscopy, dynamic light scattering, zeta-potential measurements, cryogenic transmission electron microscopy, and atomic force microscopy. Aggregation of the vesicles is induced by a twofold supramolecular interaction. First, the adamantyl group of 1 forms an inclusion complex with beta-cyclodextrin. Second, at neutral pH the guanidiniocarbonylpyrrole carboxylate zwitterion dimerizes through the formation of hydrogen-bonded ion pairs. Because the dimerization of 1 depends on the zwitterionic protonation state of 1, the aggregation of the cyclodextrin vesicles is also pH dependent; the cyclodextrin vesicles do not interact at pH 5 or 9, at which 1 is either cationic or anionic and, therefore, not self-complementary. These observations are consistent with molecular recognition of the vesicles through a combination of two different supramolecular interactions, that is, host-guest inclusion and dimerization of zwitterions, at the bilayer membrane surface.
Related Concept Videos
 01:43
SNAREs and Membrane Fusion
SNAREs exist in pairs that symmetrically interact and catalyze the fusion of the lipid bilayers in vesicle and target organelle. v-SNARE in the vesicle membrane are single polypeptide chains that bind to a complementary t-SNARE, composed of 2...
 01:12
Clathrin Coated Vesicles
 01:14
Rab Proteins
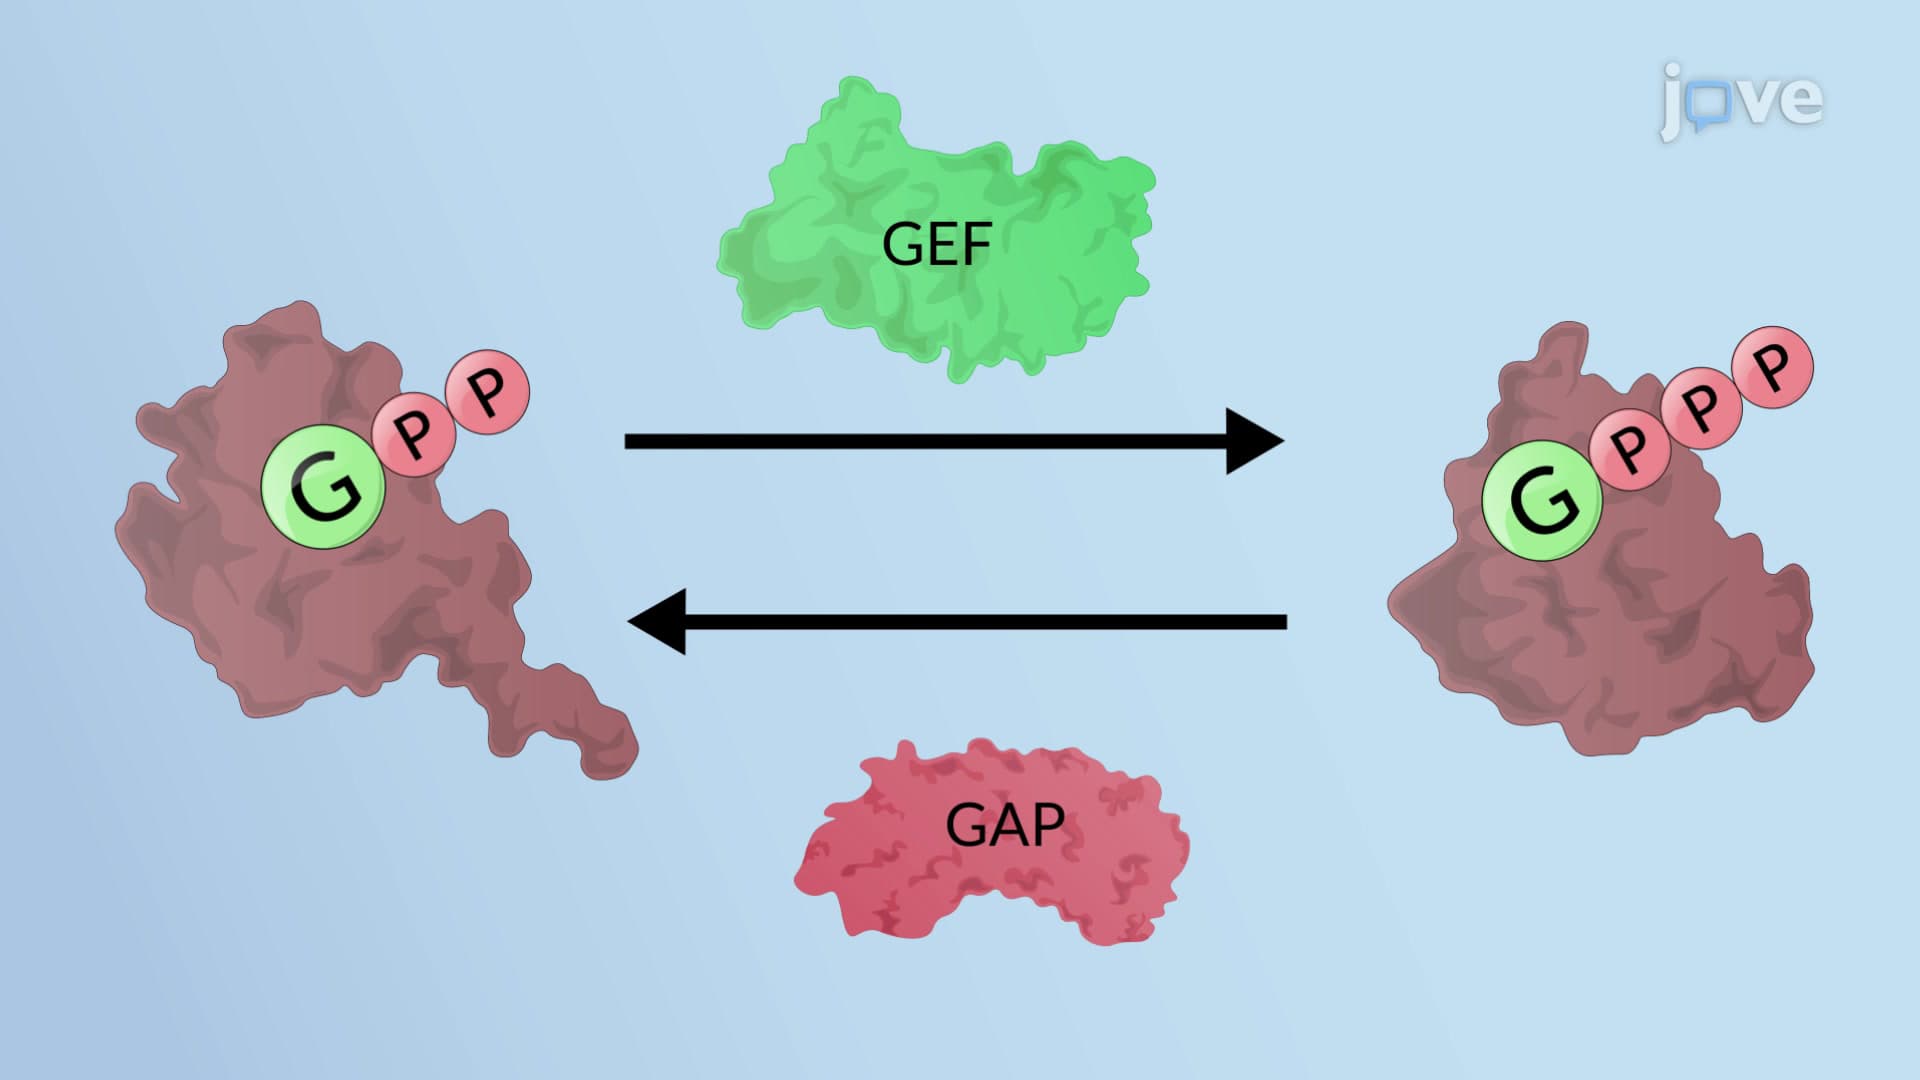
Rab proteins switch between a cytosolic, GDP-bound inactive state and a membrane-anchored, GTP-bound active state. By themselves, Rabs show slow rates of GDP/GTP exchange and GTP hydrolysis. Thus, Rab proteins are considered...
 01:43
The Movement of Organelles and Vesicles
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...
 01:32
Pinching-off of Coated Vesicles