Related Experiment Video
Updated: Jun 8, 2026

Method to Visualize and Analyze Membrane Interacting Proteins by Transmission Electron Microscopy
Published on: March 5, 2017
Long-range protein coupling mediated by critical low-energy modes of tubular lipid membranes
Sylvain Monnier1, Sergei B Rochal, Andrea Parmeggiani
1Laboratoire de Physique Théorique et Astroparticules, CNRS, Université Montpellier II, Pl. E. Bataillon, 34095 Montpellier Cedex 5, France.

Abstract:
We develop a theory of a resonant effect in protein-membrane coupling taking place in the vicinity of instabilities in tubular lipid membranes (TLMs) under longitudinal force and pressure difference constraints. Two critical low-energy modes defining the stability domain boundaries are found. We show that these modes mediate long-range TLM-protein coupling and interactions between absorbed proteins. Besides, TLM mechanical instabilities strongly influence protein desorption and protein cluster nucleation on TLMs. Model predictions can be tested over a large spectrum of mechanochemical conditions.
More Related Videos
 08:55
Single-Molecule Imaging of Lateral Mobility and Ion Channel Activity in Lipid Bilayers using Total Internal Reflection Fluorescence (TIRF) Microscopy
Published on: February 17, 2023
 07:49
Spontaneous Formation and Rearrangement of Artificial Lipid Nanotube Networks as a Bottom-Up Model for Endoplasmic Reticulum
Published on: January 22, 2019
Related Concept Videos
 01:24
Protein Diffusion in the Membrane
 00:59
Mechanisms of Membrane Domain Formation
Another mechanism for membrane domain formation involves membrane proteins interacting with cytoskeletal...
 01:20
Cotranslational Protein Translocation
Sec61 channel partners for cotranslational translocation
During cotranslational translocation, the Sec61 channel partners with the signal recognition particle (SRP), the signal recognition particle receptor (SR), and the ribosomes to transport the nascent polypeptide chain...
 01:09
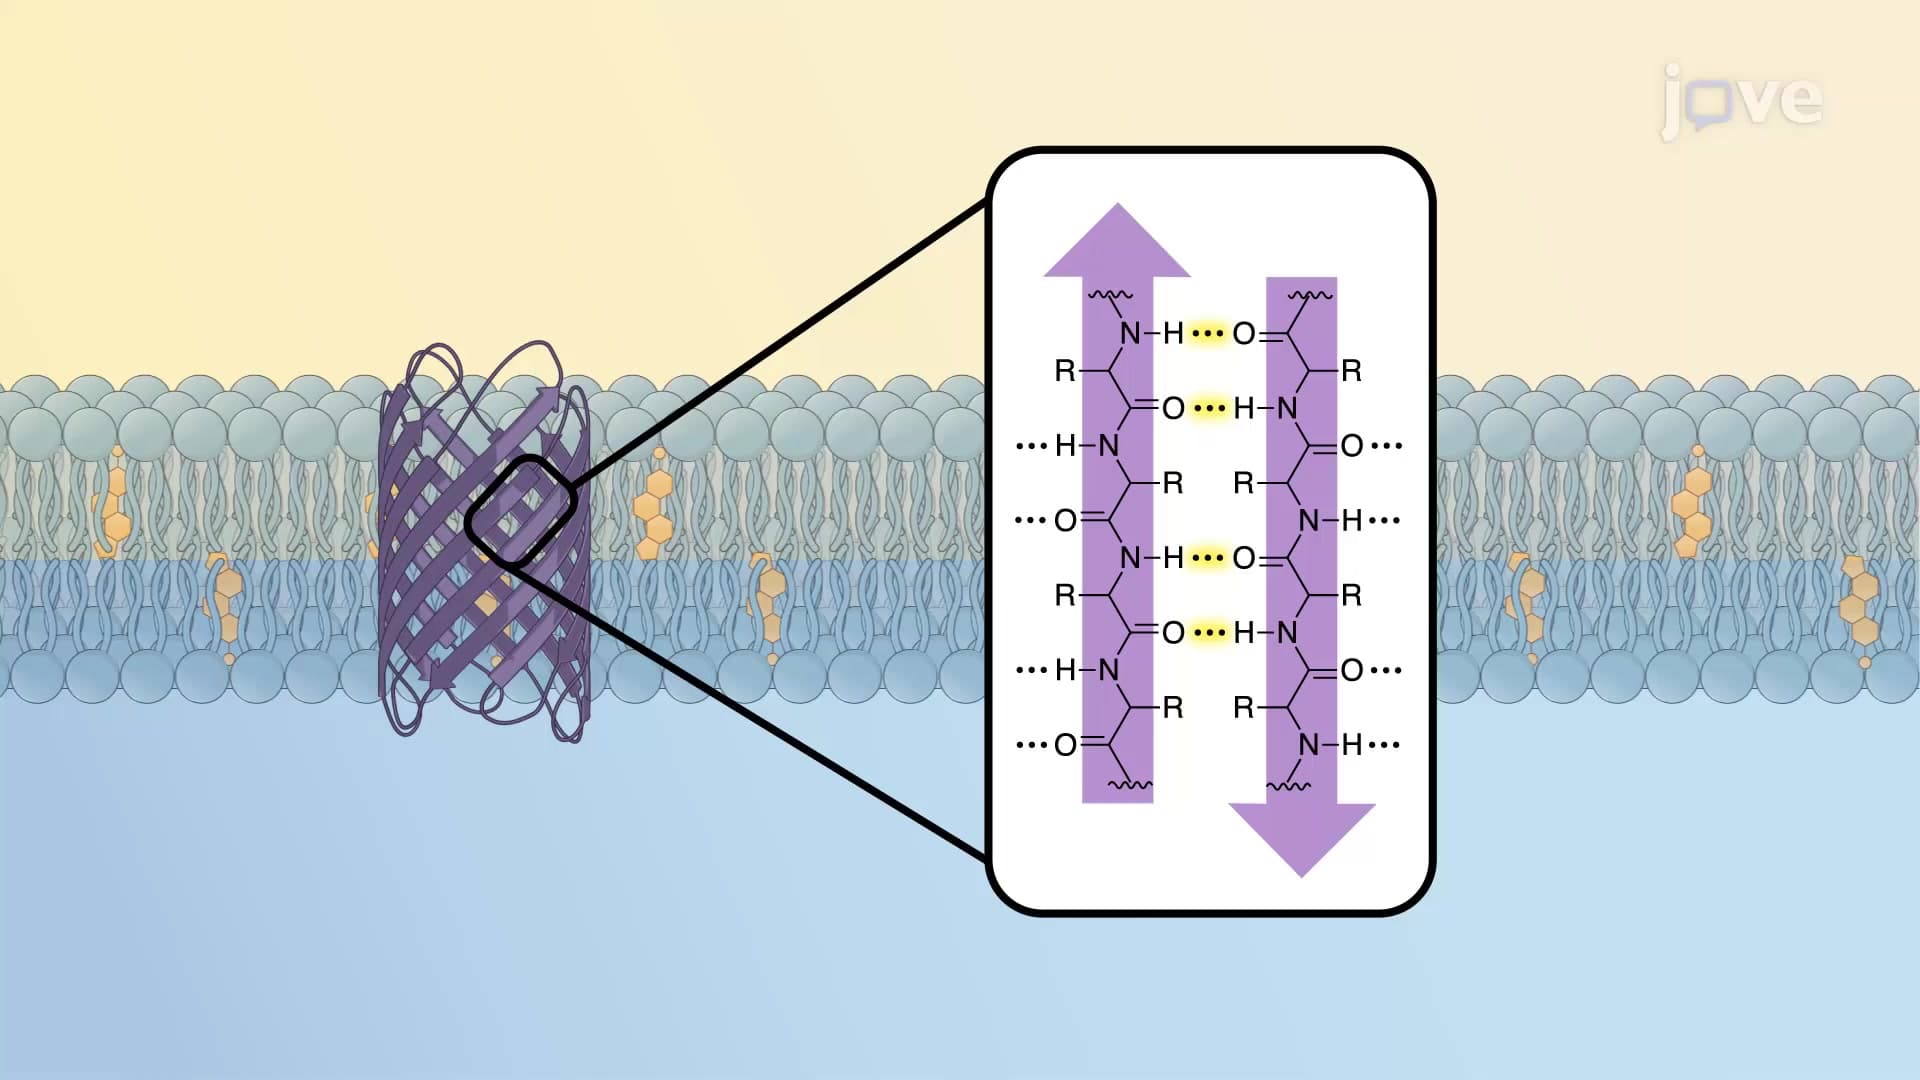
Multi-pass Transmembrane Proteins and β-barrels
α-Helix containing multi-pass transmembrane proteins
Multi-pass transmembrane proteins such as G-protein-linked receptors (GPCRs) and...
 01:28
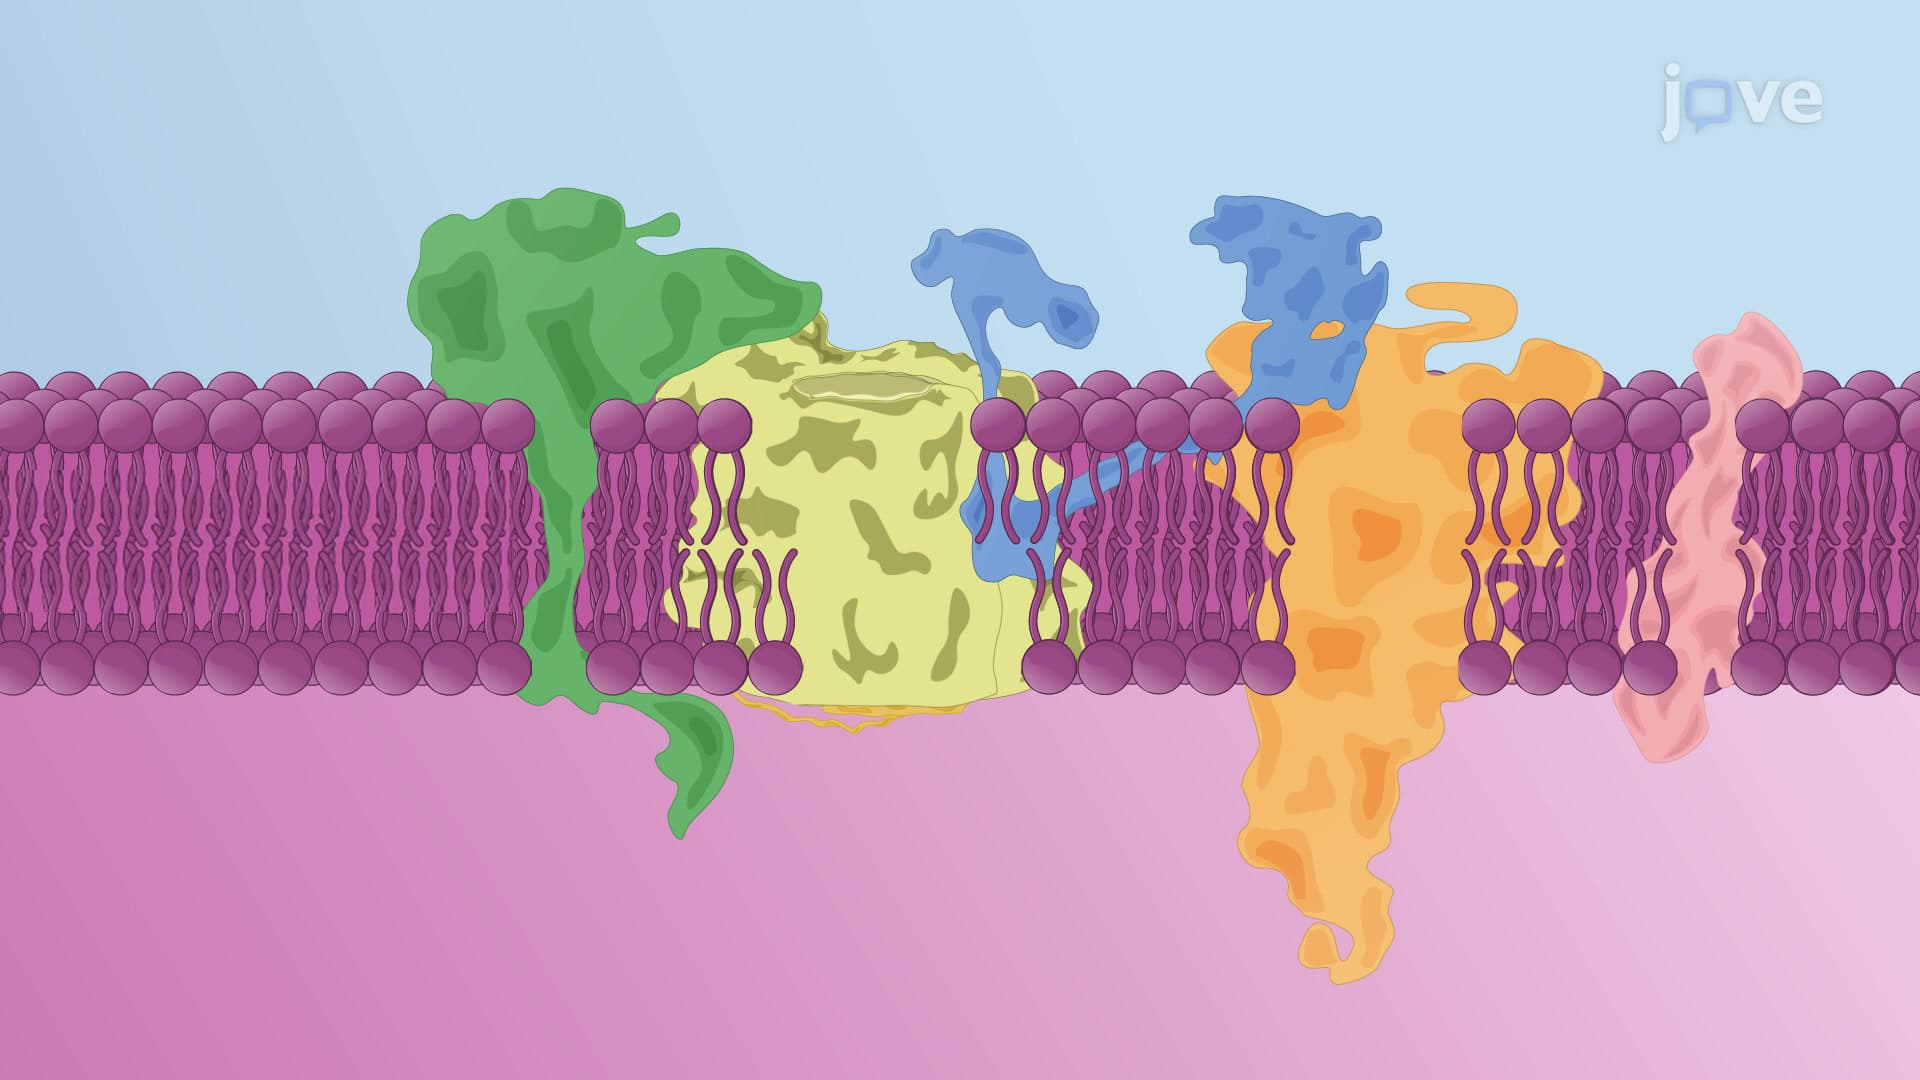
Protein Translocation Machinery on the ER Membrane
Sec61 protein conducting channel
In eukaryotes, the translocon complex comprises a core heterotrimeric translocator channel called the Sec61 complex. This channel includes three transmembrane proteins, Sec61α, Sec61β, and Sec61γ, and is the largest subunit of the translocon complex.
 01:15
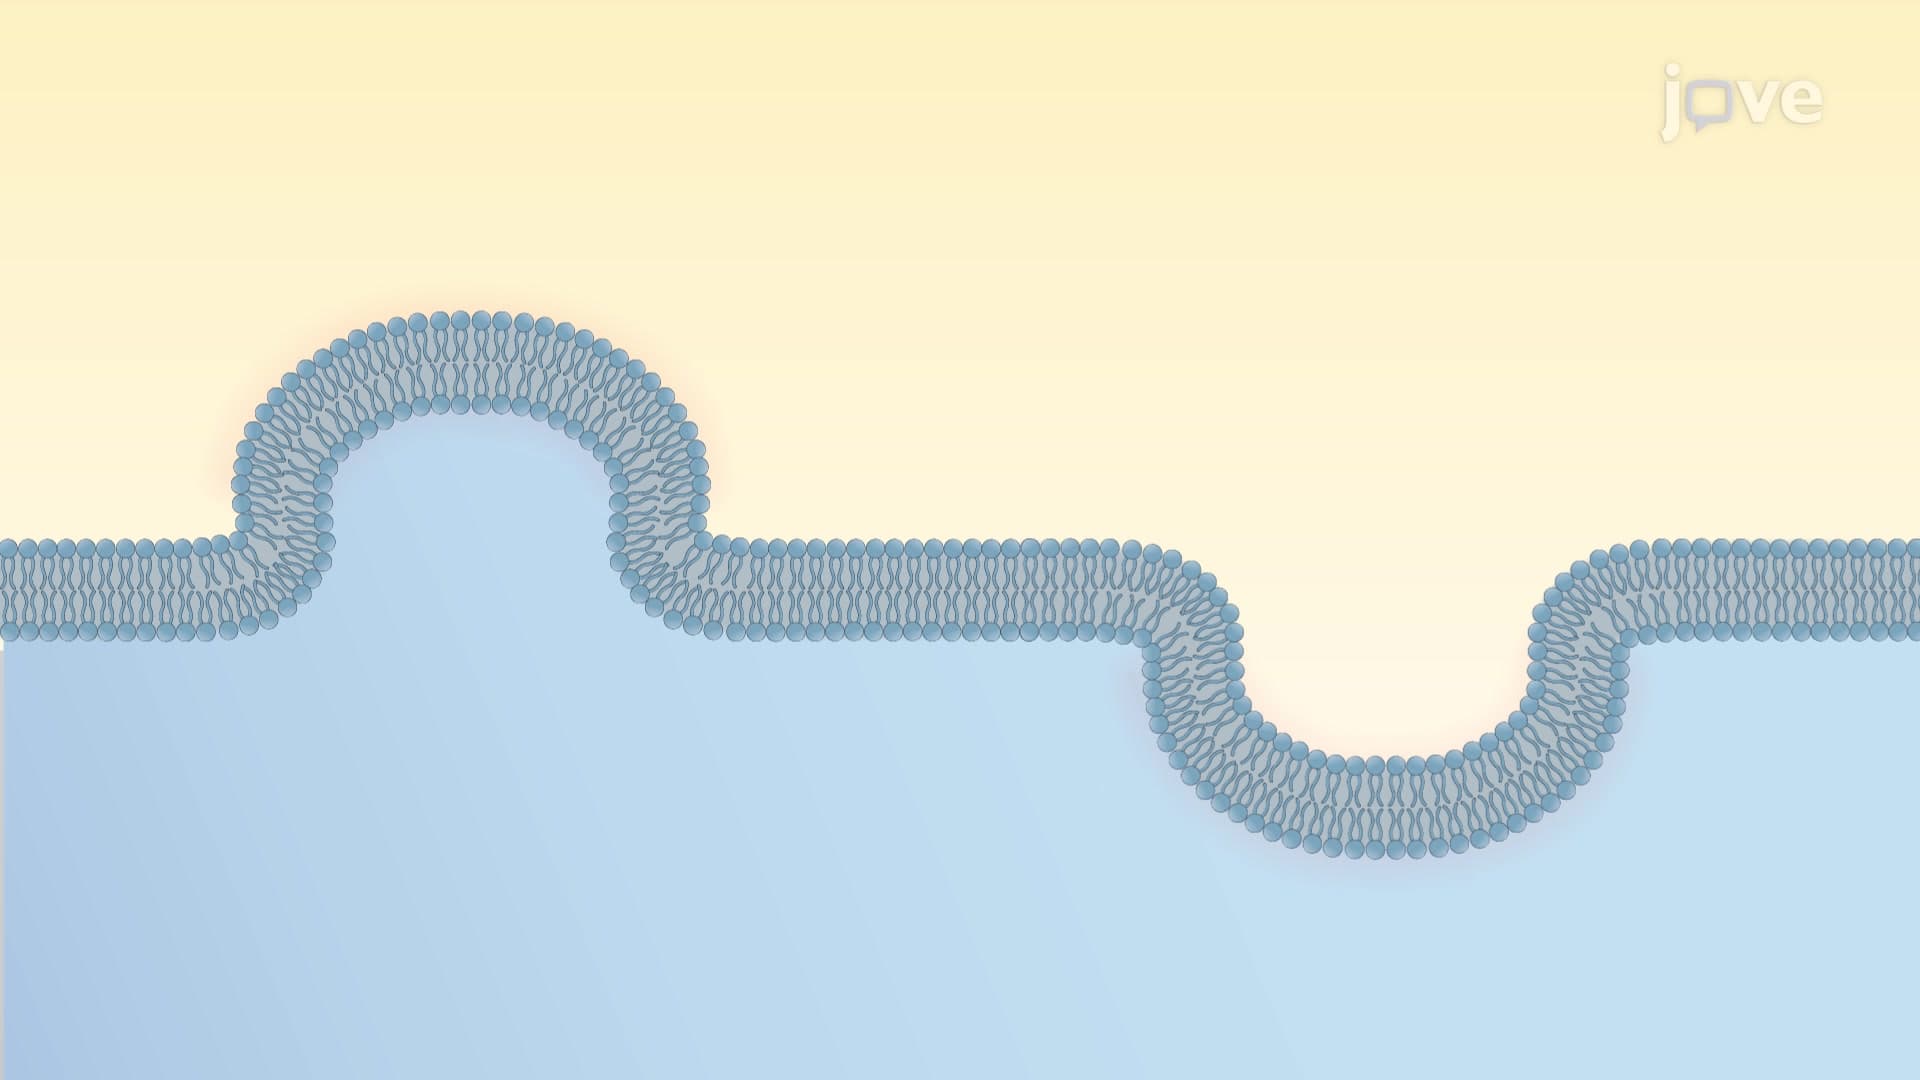
Mechanisms of Membrane-bending
Membrane bending can happen due to intrinsic changes in lipid composition or extrinsic association with different proteins. The proteins involved...