Related Experiment Video
Updated: Jun 8, 2026
From Constructs to Crystals – Towards Structure Determination of β-barrel Outer Membrane Proteins
Published on: July 4, 2016
NMR and X-ray structures of the putative sterol carrier protein 2 from Thermus thermophilus HB8 show conformational
Alexander K Goroncy1, Kazutaka Murayama, Mikako Shirouzu
1RIKEN Systems and Structural Biology Center, Yokohama, Kanagawa, Japan.

Abstract:
Sterol carrier protein 2 (SCP-2), also known as nonspecific lipid transfer protein, is a ubiquitous intracellular ~13 kDa protein found in mammals, insects, plants, archaea, and bacteria. Vertebrate SCP-2 has been implicated in a wide range of lipid-related functions in vitro, although its actual physiological role is still unknown. Tunnels in the protein serve as fatty acid binding vehicles. Here we report the first putative SCP-2 structure from a bacterium: specifically, the NMR and X-ray structures of the TTHA0401 protein (also designated as TT1886) from the extremely thermophilic bacterium Thermus thermophilus. The NMR structure and the two chain structures (chain A and chain B) of the asymmetric crystallographic unit (space group (P2(1)2(1)2(1))) revealed an internal cavity. However, this cavity is open to the outside, forming a tunnel, in only one of those structures (chain A, X-ray). The location of this tunnel is different from the one found in other SCP-2 proteins, and inaccessible cavities have not been seen before in SCP structures. We present evidence that at physiological concentrations, TTHA0401 likely exists as a monomer in equilibrium between open and closed conformations. This equilibrium is influenced by temperature-dependent dynamics, and is likely to be very different at the high temperatures preferred by this hyperthermophilic bacterium. Alternatively, another protein binding to TTHA0401 may induce a conformational change, which would constitute an intriguing metabolic regulation method in bacteria.
More Related Videos
Related Concept Videos
 01:15
¹H NMR of Conformationally Flexible Molecules: Variable-Temperature NMR
 01:09
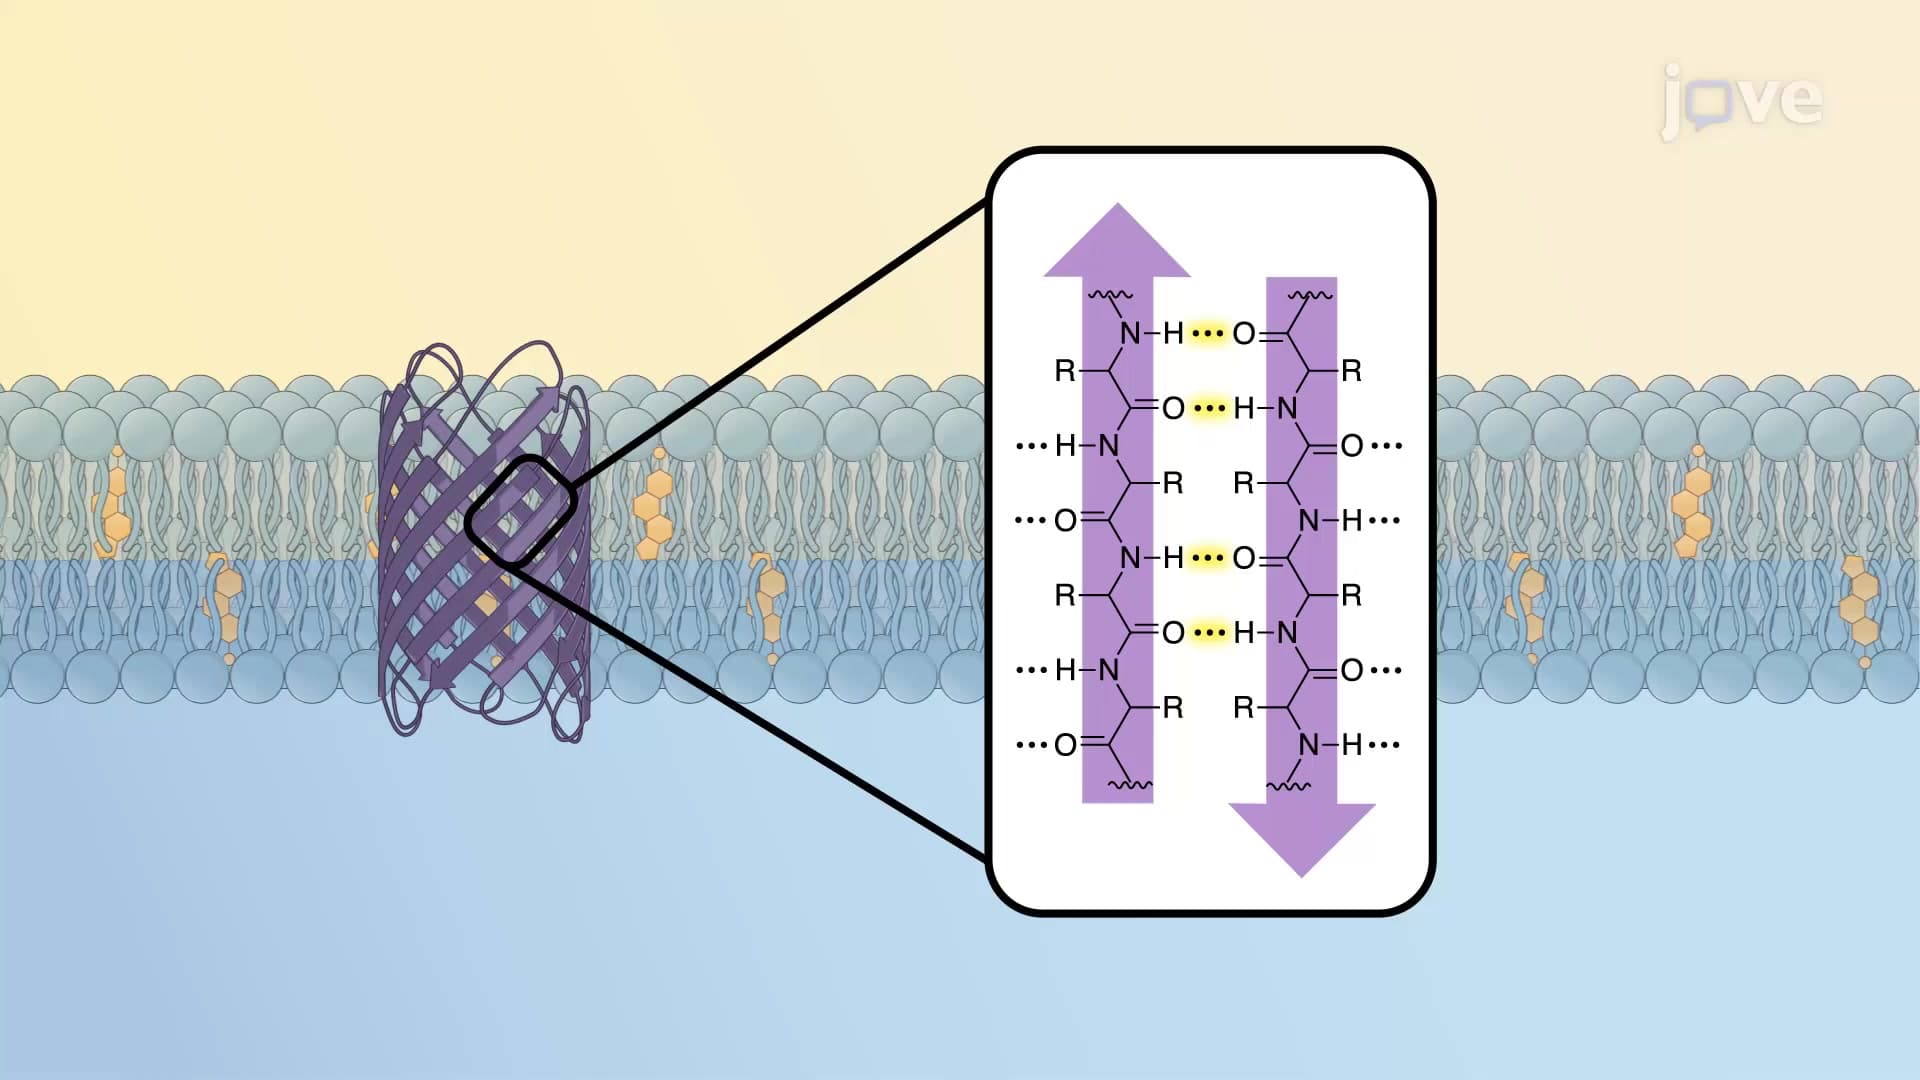
Multi-pass Transmembrane Proteins and β-barrels
α-Helix containing multi-pass transmembrane proteins
Multi-pass transmembrane proteins such as G-protein-linked receptors (GPCRs) and...
 00:52
¹H NMR of Conformationally Flexible Molecules: Temporal Resolution
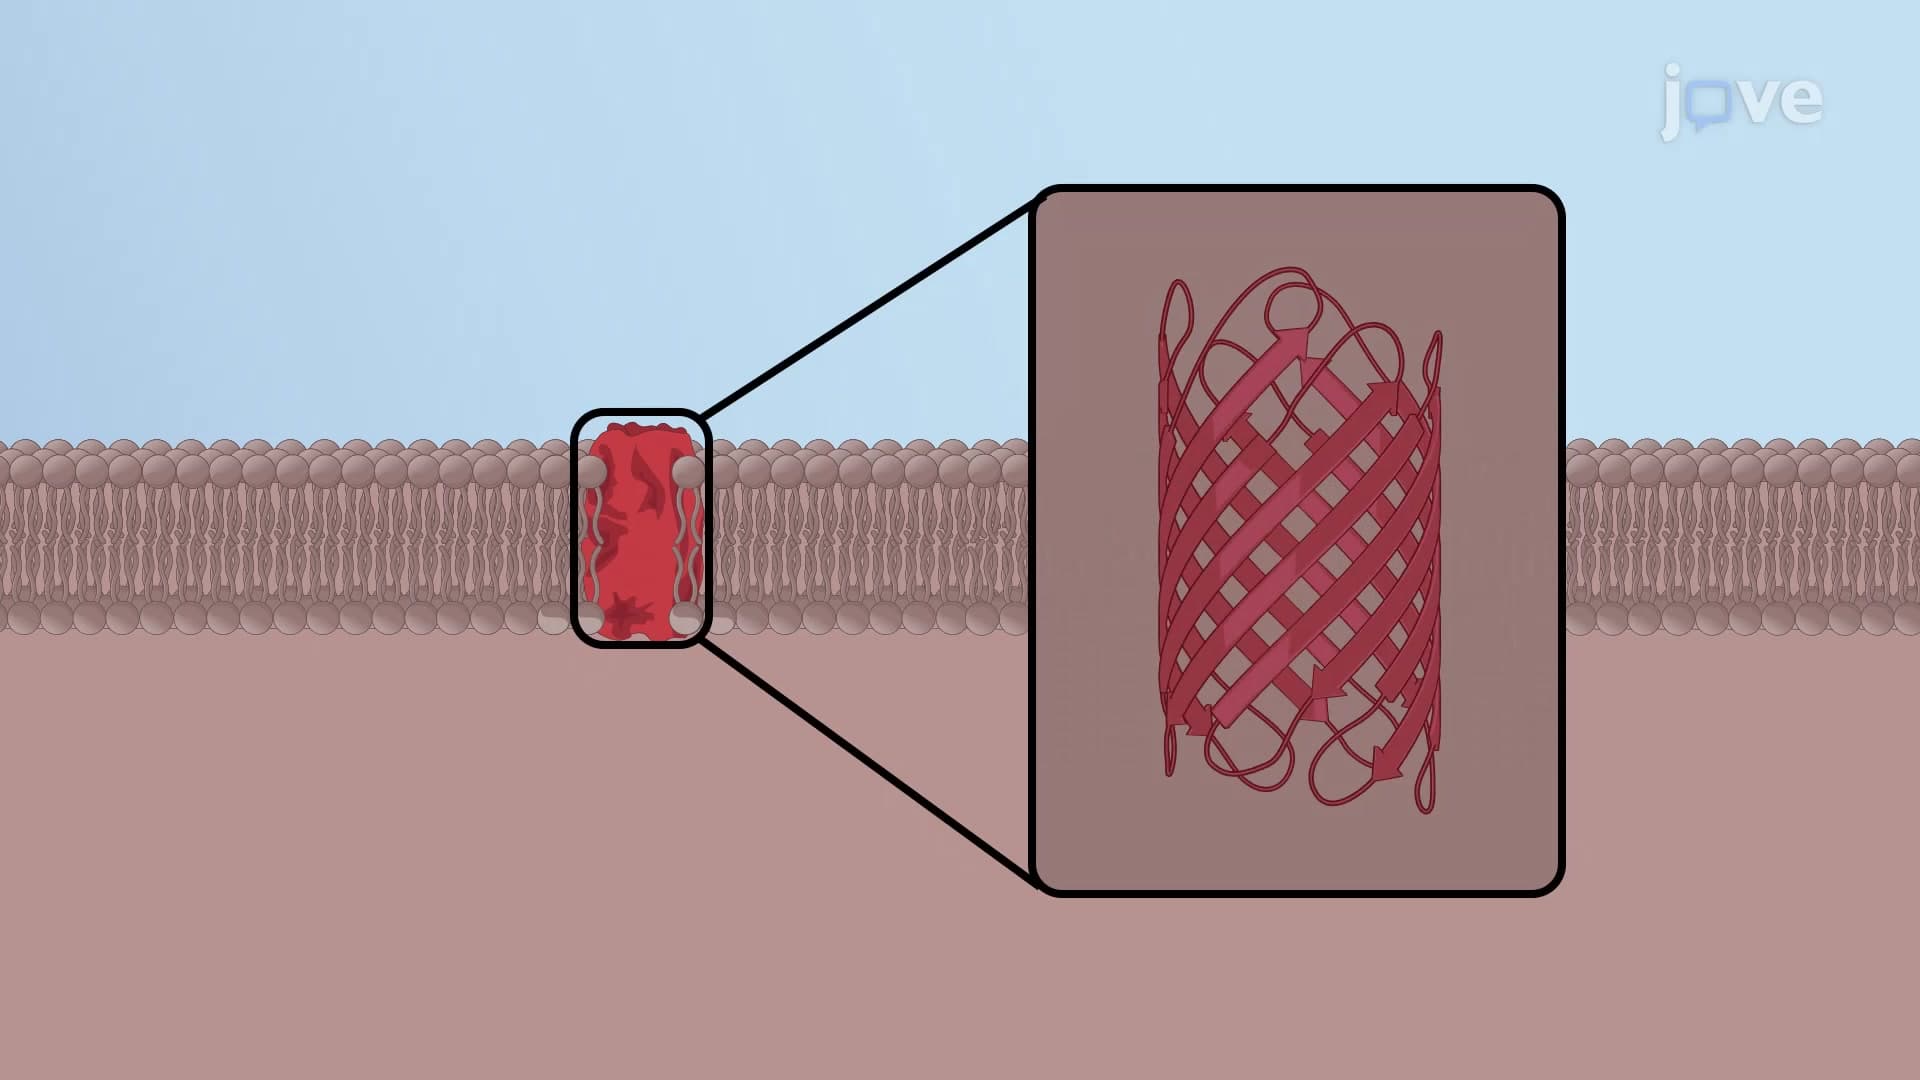 01:21
Structure of Porins
 01:45
Regulation of Nuclear Protein Sorting
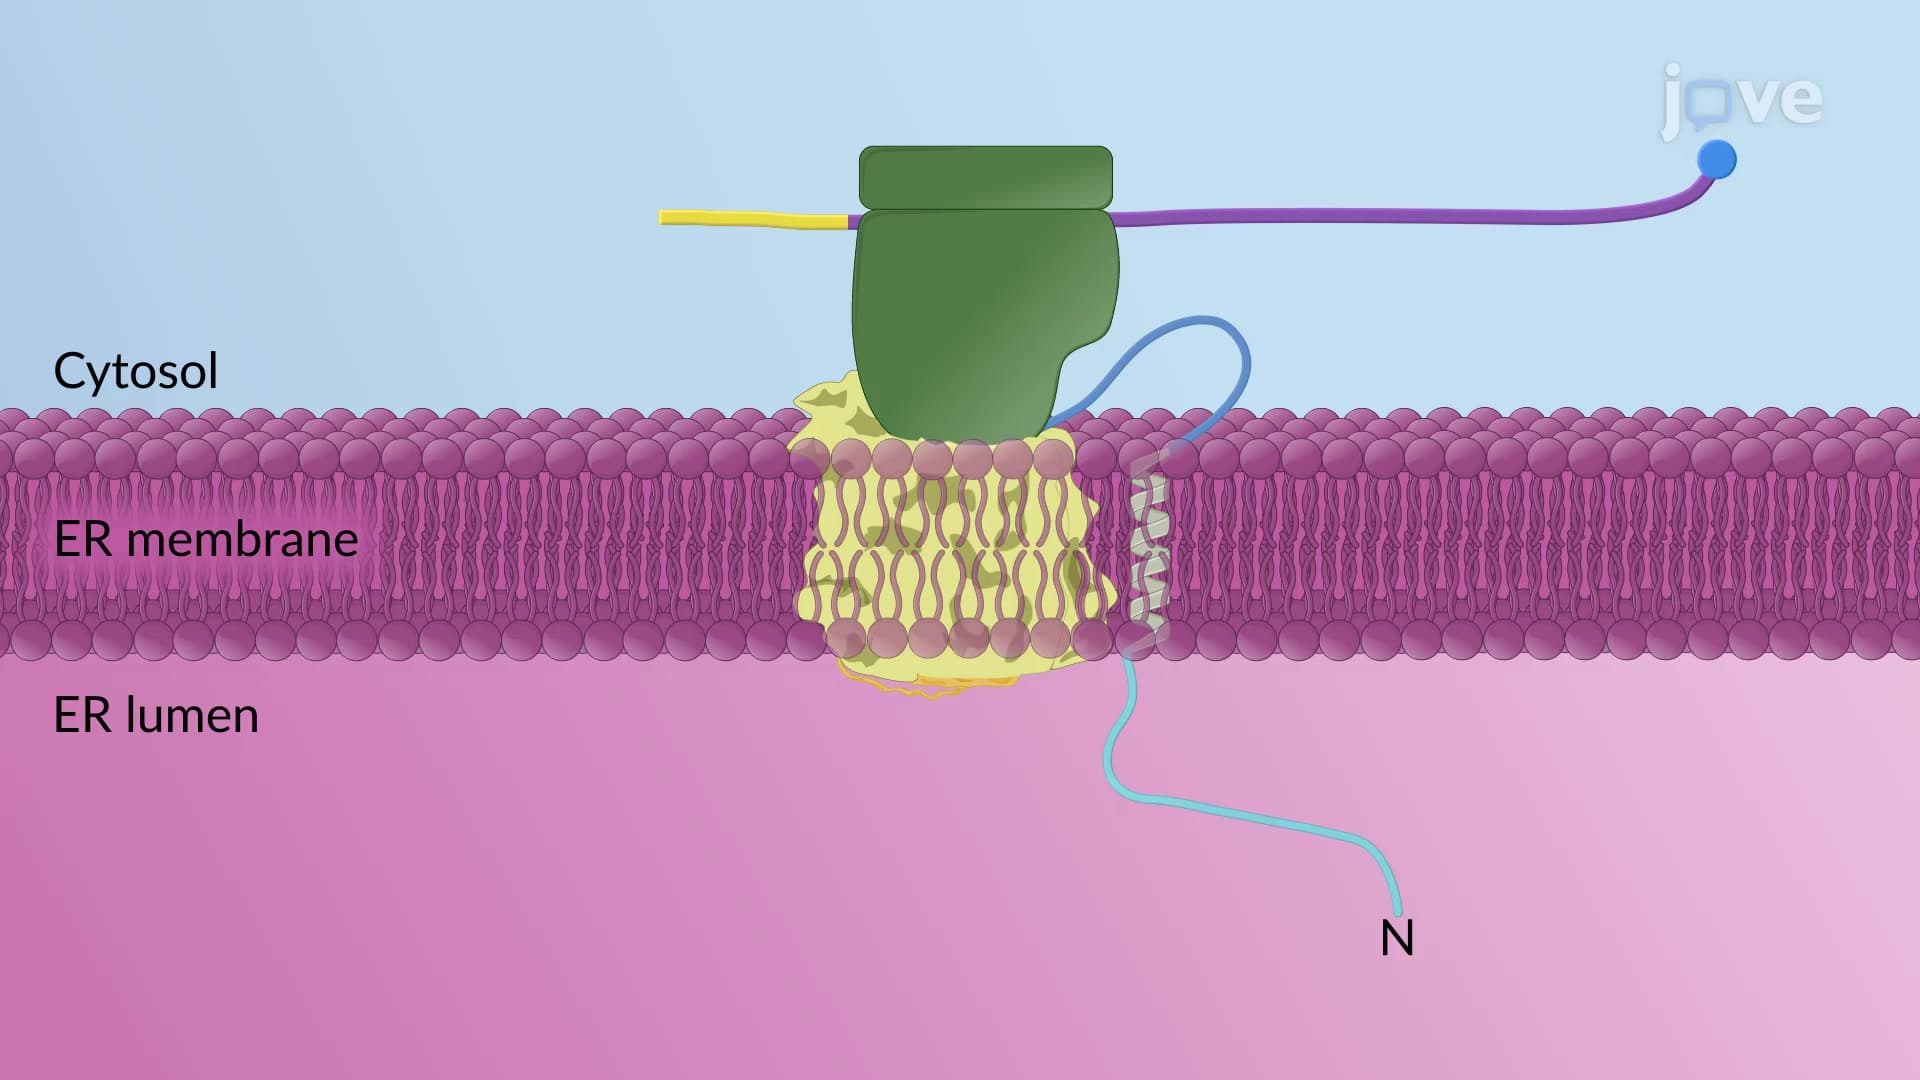 01:26
Insertion of Single-pass Transmembrane Proteins in the RER
Integral transmembrane proteins possess transmembrane and extra membrane domains. The transmembrane domains are primarily made of 20-25 hydrophobic amino acids arranged in a helical secondary confirmation. These...